Topics (384k) Articles (398k) Users (410) Discussions (242) Comments (383) Files (13k) New article
A monosaccharide is a single-unit carbohydrate that cannot be split into smaller sugars by hydrolysis. Ribose, deoxyribose, and glucose are examples. The unit is a whole molecule containing many chemical atoms; a disaccharide instead contains two linked monosaccharide units.[ref]
25.1 Classification of Carbohydrates. McMurry, Organic Chemistry, §25.1: simple and complex carbohydrates
Classification combines carbon count with open-chain connectivity. An aldose has an aldehyde group; a ketose has a ketone group. Thus glucose is an aldohexose, while fructose is a six-carbon ketose. These names describe the open-chain reference forms even when cyclic forms predominate in water.[ref]
25.1 Classification of Carbohydrates. McMurry, Organic Chemistry, §25.1: aldoses, ketoses and carbon-count classification
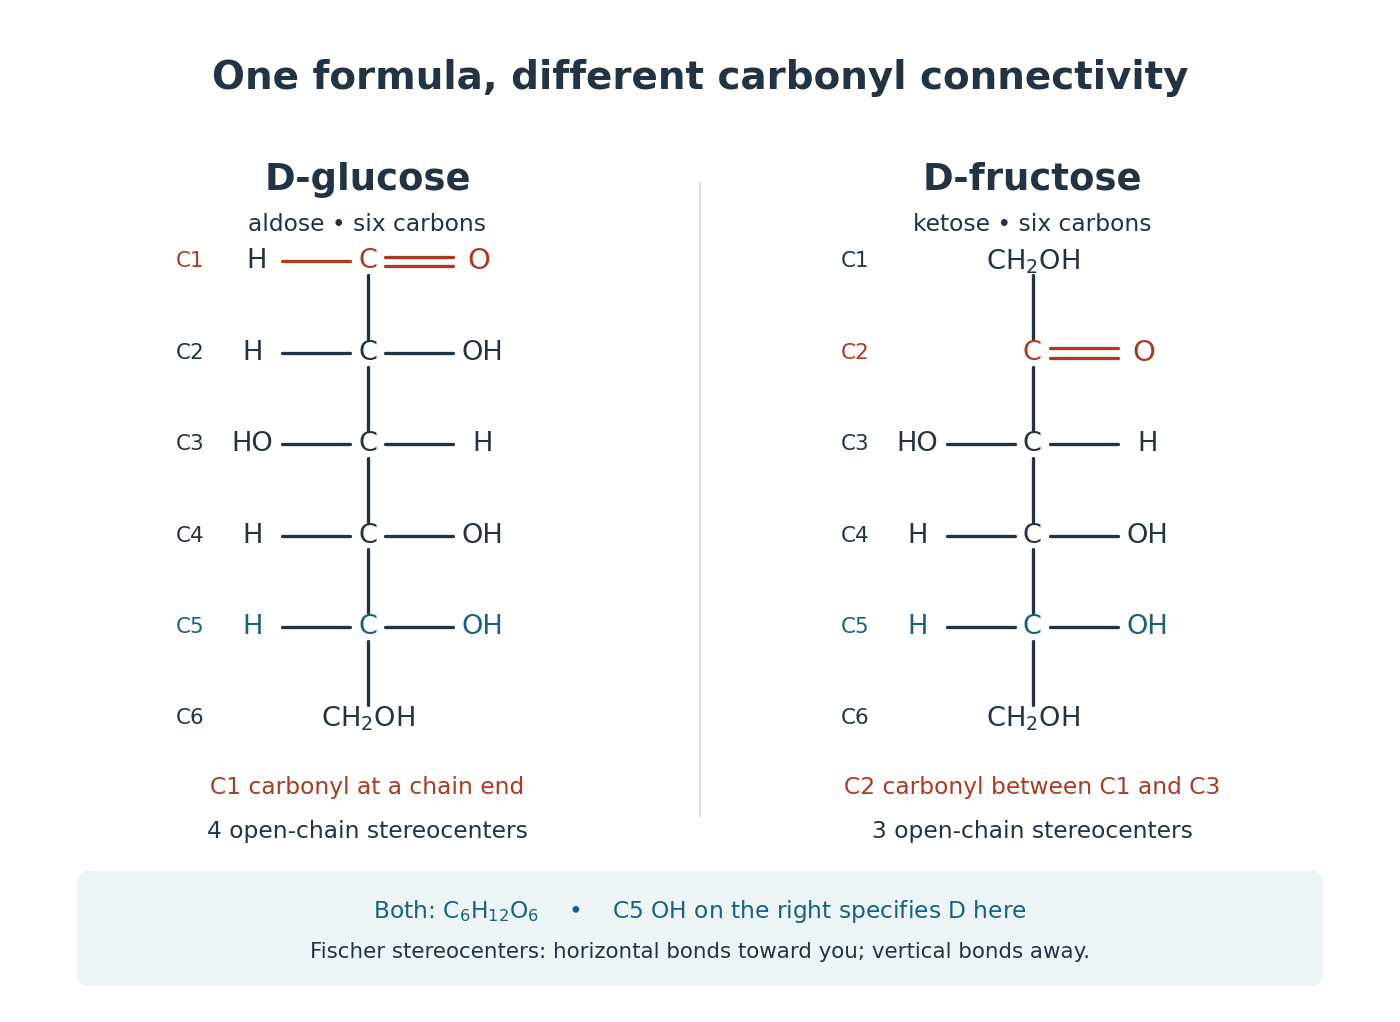
Open-chain D-glucose and D-fructose: the same molecular formula, different carbonyl group connectivity
. Original numbered Fischer projections. At tetrahedral stereocenters, horizontal chemical bonds point toward the viewer and vertical chemical bonds away. The carbonyl group carbon is not a tetrahedral stereocenter. The C5 hydroxy group on the right specifies D here; D does not specify the sign of optical rotation. These reference structures do not show relative abundances in water. Details.Check the distinction by counting the groups in the drawings. Open-chain glucose contains one , four and one group. Open-chain fructose contains two , three and one group. The respective hydrogen totals are and ; each structure also has six carbon and six oxygen chemical atoms. Their shared molecular formula therefore cannot identify the carbonyl group position or the stereochemistry.
The beauty is that a familiar sugar name can embrace an interconverting family of forms. Monosaccharide ring-chain interconversion connects those drawings to mutarotation, a change visible with polarimetry. Spatial arrangement also matters to biology: an enzyme's active site encounters a particular arrangement of hydroxy groups, rather than merely an inventory of chemical atoms. The existing enzyme and chirality articles explain that recognition principle.
Glucose is a monosaccharide with molecular formula . Its familiar biological form, D-glucose, is an aldohexose. In the open-chain Fischer projection, is at the top and at the bottom; the hydroxy groups at C2, C3, C4, and C5 point right, left, right, right. This full pattern distinguishes D-glucose from other six-carbon aldehyde sugars. See McMurry, Organic Chemistry, 25.4: configurations of the aldoses.
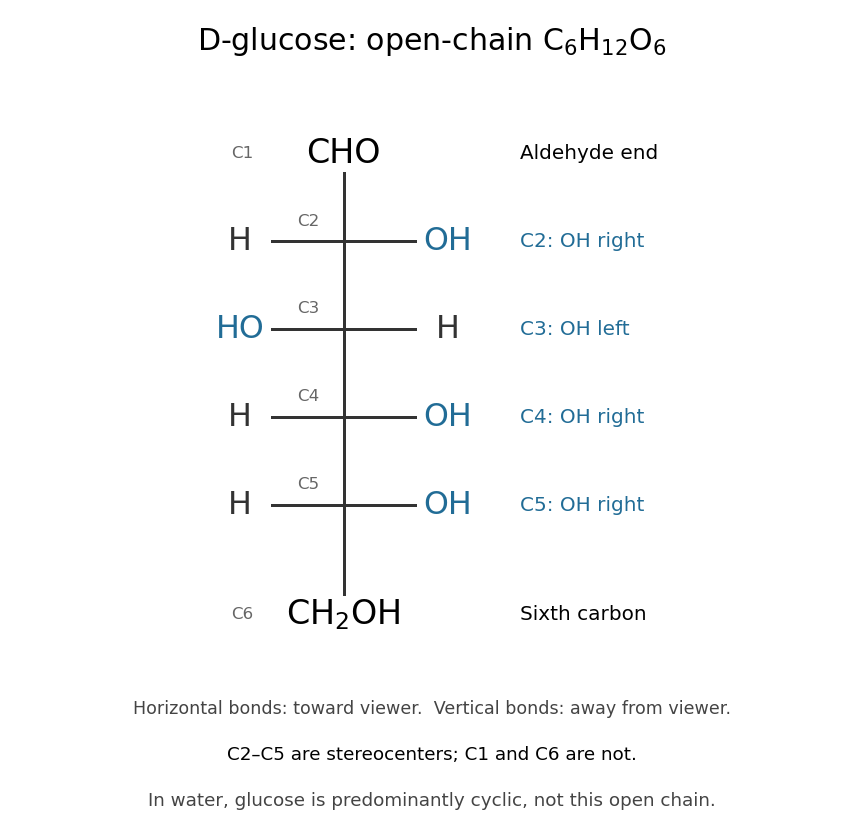
The molecular formula can be checked directly: one group, four groups, and one group give six carbon, twelve hydrogen, and six oxygen chemical atoms. All four interior carbon positions are stereocenters in this open-chain structure. Neither their orientations nor the arrangement of chemical bonds can be recovered from the molecular formula alone.
In water, glucose exists mainly in six-membered rings in chemical equilibrium with a small amount of open-chain glucose. Ring closure connects the hydroxy group at C5 to the aldehyde carbon at C1; the ring contains five carbon chemical atoms and one oxygen, with C6 outside it. No chemical atoms are lost, so the molecular formula remains . See McMurry, Organic Chemistry, 25.5: cyclic structures of monosaccharides.
Glucose is useful both as a substrate in cellular metabolism and as a building block of polysaccharides. Cellulose chains assembled from glucose units help support plant cell walls. The same small sugar thus connects chemical fuel to a structural material; its role depends on how it is transformed or linked. See Cooper, The Cell: A Molecular Approach, the molecular composition of cells.
In the usual DNA context, deoxyribose means 2-deoxy-D-ribose, a five-carbon monosaccharide with molecular formula . Relative to D-ribose, the hydroxy group at C2 is replaced by hydrogen. The locant 2 matters: it identifies which position loses its oxygen. See Favre and Powell, IUPAC Blue Book, P-102.5.3: deoxy sugars and IUPAC: nucleic acids and their component sugars.
The paired Fischer projections in ribose make the change concrete. C2 has hydrogen on both sides, while C3 and C4 retain their hydroxy groups on the right. C2 is therefore not a stereocenter: exchanging its two identical hydrogen substituents cannot produce a distinct configuration. The unchanged C3 and C4 still carry stereochemical information.
Replacing by removes one oxygen but leaves the total hydrogen count unchanged: the hydrogen belonging to the removed hydroxy group is replaced by a hydrogen bonded directly to carbon. Thus becomes . This comparison describes structures, rather than a complete chemical reaction or its mechanism.
In DNA, deoxyribose is incorporated as a ring in each nucleotide, with phosphate connections building the backbone. Its C2′ bears hydrogen where RNA's ribose bears a hydroxy group. This small local difference lets the sugar structure identify the two kinds of nucleic acid; the nucleobases supply their sequence information. See Alberts et al.: nucleotides as the subunits of DNA and RNA.
Ribose is a monosaccharide with molecular formula . Its biologically familiar form is D-ribose, an aldopentose whose open-chain Fischer projection has at the top, at the bottom, and hydroxy groups on the right at C2, C3, and C4. The opposite horizontal substituents are hydrogen. See McMurry, Organic Chemistry, 25.3: D-ribose and D-glucose configurations.
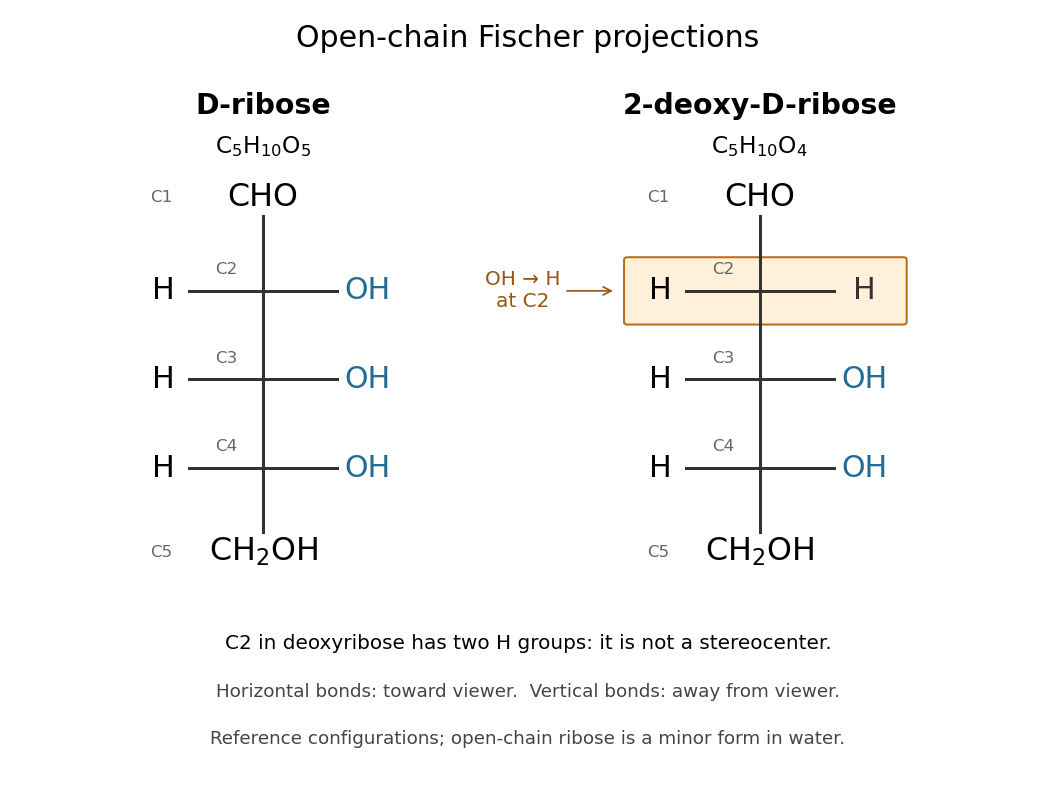
Read the drawing by counting groups: contributes , three groups contribute , and contributes . Their sum is . The count checks composition; the right/right/right pattern additionally specifies the stereochemistry of D-ribose.
In RNA, ribose occurs as a ring within each nucleotide, joining a nucleobase to the phosphate-linked backbone. Its C2 position retains a hydroxy group, unlike deoxyribose in DNA. In a nucleotide, the sugar positions carry primes, so this is C2′. See Alberts et al.: nucleotide sugars in RNA and DNA. Free ribose in water is also predominantly cyclic, with several ring forms in chemical equilibrium and very little open-chain form; the Fischer projection is valuable for comparing configurations, not for estimating their abundances. See Mason et al., The Conformation of a Ribose Derivative in Aqueous Solution: A Neutron Scattering and Molecular Dynamics Study (2013), introduction.
A statistic is ancillary for a statistical model if its probability distribution is the same for every parameter value. Its marginal law carries no information about the parameter, but its observed value can identify the precision or configuration of the experiment. Fisherian conditional inference uses the conditional distribution of an informative statistic given the observed ancillary value. Ancillarity does not mean that the ancillary is independent of every informative statistic.
For an infinite square well initially on , a normalized ground state is . If the endpoints change instantaneously to , with , the sudden approximation leaves the wave function unchanged, extended by zero outside the old well. Its overlap with the new normalized ground state is . The Born rule squares this probability amplitude; for the result is , and the limit as is .
A quantum quench changes a quantum system's control parameters rapidly and studies the subsequent unitary time evolution. In the ideal sudden limit, write an initial energy eigenstate using a complete final orthonormal eigenbasis:The Born rule probabilities for a nondegenerate final energy measurement are , with . For a degenerate energy eigenvalue, sum the probabilities over its orthonormal energy eigenstates. Subsequent relative quantum phases can alter other measurement probabilities even though these final energy populations stay fixed. A quench need not begin in an energy eigenstate; the same expansion applies to any initial pure state.
Quantum state continuity at a finite Hamiltonian step by  Codex 0 Created 2026-10-14 Updated 2026-10-18
For a fixed Hilbert space, a bounded self-adjoint Hamiltonian operator with a finite step at does not deliver an instantaneous rotation of the quantum state. Integrating the Schrödinger equation across a short interval givesFor a normalized quantum state and in operator norm, the difference has norm at most , which tends to zero. The time derivative can jump even though the quantum state is continuous. Here is the reduced Planck constant. An instantaneous replacement of the eigenbasis changes coordinates, not the vector being represented.
For a real switch occupying , remove any real scalar contribution that produces only a global phase, and write . The same integral argument gives the sufficient bounded-model estimateThus controls the sudden approximation up to a global phase. For any normalized final energy eigenstate, its probability amplitude differs from the instantaneous-switch value by at most , and its Born rule probability differs by at most . These are sufficient error bounds, not necessary criteria. For the fixed-gap two-level sudden quench, any switching path with a unit vector has operator norm , giving .
This estimate is deliberately for bounded Hamiltonian operators. An unbounded energy spectrum does not supply a finite global ; relevant quantum states, operator domains and excited energy eigenvalues require separate control. The adiabatic theorem also requires hypotheses about the path and its spectral gaps; there is no universal switch-duration criterion covering all spectra. The cold-atom collapse and revival after a lattice quench illustrates how a single switch can be sudden for one degree of freedom and slow for another.
For a real one-dimensional Sturm-Liouville problem with separated self-adjoint boundary conditions and discrete simple spectrum, the eigenfunction for the th eigenvalue has exactly interior zeros, numbering from zero. For a confining real Schrödinger operator on the line, the same ordering makes the ground state nodeless and the first excited state have one node. If the potential is even, uniqueness and reflection symmetry imply that these states are respectively even and odd.
Hydrochloric acid is an aqueous chemical solution of hydrogen chloride. The glycine titration model treats its dissociation into hydronium and chloride as complete, retaining both ions in the electric charge balance.
An S-duality relates descriptions at different coupling strengths. In type IIB superstring theory, acts on the axion-dilaton and string charge doublets.
For signature and , the convention gives the displayed tensor. Varying the inverse metric yields the derivative product, while varying the volume element yields the term proportional to . A homogeneous field has energy density and pressure .
The metric variational stress tensor is defined by the matter action's response to a metric change. With signature and the corresponding usual matter-action signs, the displayed convention means . Fix the independent matter variables while varying the metric. Sign conventions must be matched to the action; copying a mostly-plus stress formula into this convention can reverse its energy density.
For a steady axisymmetric compressible fluid flow, mass conservation permits this representation. The mass flow through an annulus between two stream surfaces is . In a steady adiabatic wind without magnetic forces, the specific entropy, specific angular momentum and Bernoulli function are locally functions of on connected regular stream surfaces.
The incompressible planar field has the displayed stream function under and vorticity . In rotated coordinates , , . For positive parameters its nonstationary streamlines are closed ellipses if , hyperbolas and straight separatrices if , and parallel straight lines with a stationary diagonal if .
Using , the displayed stream function gives . Its streamlines are level sets of . At , the Jacobian matrix is , so the points are saddle equilibria. At the eigenvalues are , giving center equilibria surrounded by closed streamlines. The grid lines and form heteroclinic orbits between adjacent saddles; circulation alternates between cells.
For a discrete space and , the continuous extension of to remains idempotent by density, so it takes values in . Its one-set is the clopen closure of . If is any open set in , density gives , so this closure is clopen as well. Thus is an extremally disconnected space. For infinite , this does not imply that every subset of has open closure.
Clopen separation in discrete Stone-Čech compactifications by Codex 0 Created 2026-10-14 Updated 2026-10-31
Codex 0 Created 2026-10-14 Updated 2026-10-31In the Stone-Čech compactification of a discrete space, the closure of each subset of is clopen, because its indicator extends to a continuous zero-one-valued function. For disjoint closed sets , choose on and on by Urysohn's lemma. Then and are disjoint clopen sets containing and , respectively. Density proves these containments.
Polycondensation is step-growth polymerization in which joining reactions eliminate small molecules. Its chain-bearing molecule count excludes those byproducts; otherwise two chains joining while releasing one small product would misleadingly appear to conserve the counted population.[ref]
IUPAC Compendium of Chemical Terminology, fifth edition (Gold Book) by International Union of Pure and Applied Chemistry. polycondensation, P04722, definition and growth-step equation
Pinned article: Introduction to the OurBigBook Project
Welcome to the OurBigBook Project! Our goal is to create the perfect publishing platform for STEM subjects, and get university-level students to write the best free STEM tutorials ever.
Everyone is welcome to create an account and play with the site: ourbigbook.com/go/register. We belive that students themselves can write amazing tutorials, but teachers are welcome too. You can write about anything you want, it doesn't have to be STEM or even educational. Silly test content is very welcome and you won't be penalized in any way. Just keep it legal!
Intro to OurBigBook
. Source. We have two killer features:
- topics: topics group articles by different users with the same title, e.g. here is the topic for the "Fundamental Theorem of Calculus" ourbigbook.com/go/topic/fundamental-theorem-of-calculusArticles of different users are sorted by upvote within each article page. This feature is a bit like:
- a Wikipedia where each user can have their own version of each article
- a Q&A website like Stack Overflow, where multiple people can give their views on a given topic, and the best ones are sorted by upvote. Except you don't need to wait for someone to ask first, and any topic goes, no matter how narrow or broad
This feature makes it possible for readers to find better explanations of any topic created by other writers. And it allows writers to create an explanation in a place that readers might actually find it.
Figure 1. Screenshot of the "Derivative" topic page. View it live at: ourbigbook.com/go/topic/derivativeVideo 2. OurBigBook Web topics demo. Source. - local editing: you can store all your personal knowledge base content locally in a plaintext markup format that can be edited locally and published either:This way you can be sure that even if OurBigBook.com were to go down one day (which we have no plans to do as it is quite cheap to host!), your content will still be perfectly readable as a static site.
- to OurBigBook.com to get awesome multi-user features like topics and likes
- as HTML files to a static website, which you can host yourself for free on many external providers like GitHub Pages, and remain in full control

Figure 2. You can publish local OurBigBook lightweight markup files to either OurBigBook.com or as a static website.
Figure 3. Visual Studio Code extension installation.
Figure 5. . You can also edit articles on the Web editor without installing anything locally. Video 3. Edit locally and publish demo. Source. This shows editing OurBigBook Markup and publishing it using the Visual Studio Code extension. 
- Infinitely deep tables of contents:




All our software is open source and hosted at: github.com/ourbigbook/ourbigbook
Further documentation can be found at: docs.ourbigbook.com
Feel free to reach our to us for any help or suggestions: docs.ourbigbook.com/#contact