Topics (384k) Articles (398k) Users (410) Discussions (242) Comments (383) Files (13k) New article

A neuronal firing threshold specifies the condition for initiating an action potential. The leaky integrate-and-fire model uses a prescribed membrane potential ; real initiation involves active voltage-gated ion channels and depends on recent activity and recording site. A threshold drawn on a passive voltage trace is a comparison criterion, not a simulated action potential.
Temporal summation is overlap of responses to inputs arriving at different times. It can occur at one repeatedly activated synapse or across several synapses; it is not defined by reuse of a particular contact. For prescribed electric current inputs in a passive compartment, residual depolarization from earlier pulses changes the voltage reached by later pulses. The membrane time constant sets how rapidly that residual decays, while the duration of synaptic conductance and spatial filtering by a passive dendritic cable can add other timescales.
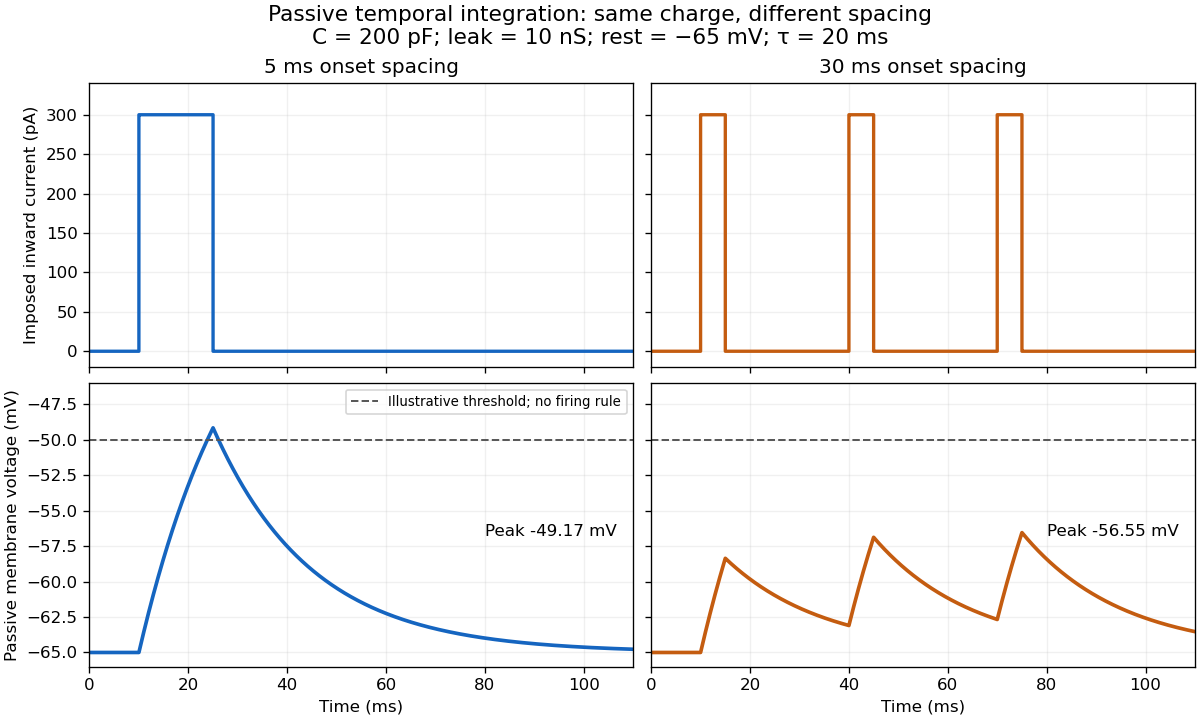
For the diagram, write , choose inward-positive imposed electric current , and use the ordinary differential equationA rectangular pulse of amplitude and duration , starting from rest, ends withAfterwards its contribution decays as . The superposition principle therefore gives, at the end of the third pulse with onset spacing ,For this is , so the peak membrane potential is . For it is , giving . Both protocols inject of electric charge; equal charge does not imply equal peak voltage because the leak drains charge while it is delivered.
In the adjacent-pulse case, the illustrative neuronal firing threshold is crossed at . A leaky integrate-and-fire model would emit its first event there and reset, so its later trajectory would differ from the passive diagram. The widely spaced train never reaches that threshold. Thus changing input timing alone can change whether an event occurs. A real neuron's neuronal firing threshold is also state-dependent, and synaptic conductance pulses are not prescribed electric current pulses.[ref]
Measured responses to repeated presynaptic action potentials may also change through synaptic plasticity. A larger second response can therefore reflect a stronger second input as well as residual postsynaptic voltage. To isolate passive temporal summation, compare known injected electric current waveforms with their single-pulse responses under stable recording conditions; to test actual synapses, measure whether input efficacy changes. These are proposed discriminating comparisons, not additional controls claimed for the slice experiment.[ref]
Spatial summation combines inputs arriving at different synapses. Location matters because a dendrite has axial electrical resistance and leaky membrane capacitance: a local synaptic potential need not arrive at the soma with its original amplitude or time course. A passive dendritic cable makes this attenuation explicit. The superposition principle applies to fixed electric current inputs in a linear passive model, but adding synaptic conductances changes the model's coefficients. Compare voltage changes relative to the same baseline, rather than adding absolute membrane potentials.
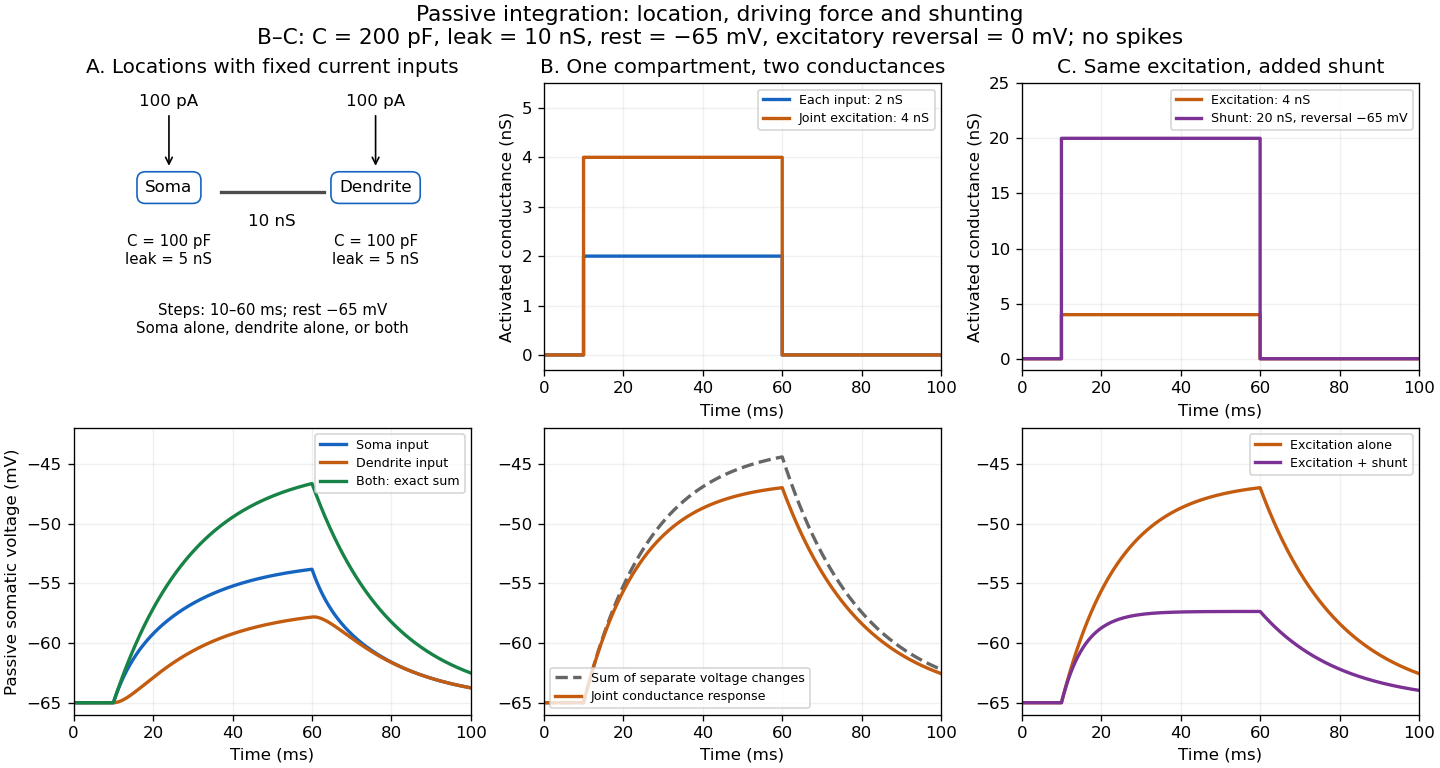
A motivating experiment. A 2004 study used – cortical slices from –-day-old rats at –. Somatic whole-cell recordings measured EPSPs in layer-5 pyramidal neurons. Two fine stimulating electrodes were positioned beside imaged dendrites; calcium-sensitive dye localized activation. Each site was stimulated alone, then both together, usually with paired pulses apart. Comparing the combined voltage trace with the sum of individual changes tested the summation rule. Nearby inputs on one branch showed strong amplification at intermediate strengths; inputs on different branches were approximately linear.[ref]
Computational subunits in thin dendrites of pyramidal cells by Alon Polsky and others. pp. 622–623, Figures 1–2; p. 626, Methods
Blocking both excitatory receptor classes eliminated voltage and calcium responses, checking against direct electrical activation. NMDA receptor blockers eliminated or markedly reduced amplification; comparisons with inhibition intact and blocked addressed inhibitory contributions. These controls support local active integration. Passing axons could still recruit unintended synapses; somatic voltage does not measure every local membrane potential. The study tested subthreshold slice responses and pairs of branches, not arbitrary activity in an intact brain.[ref]
Computational subunits in thin dendrites of pyramidal cells by Alon Polsky and others. pp. 622–624: controls; pp. 625–626: limitations
A synaptic potential is a postsynaptic change in membrane potential caused by activity at a synapse. Unlike the regenerative action potential, a passive synaptic potential is graded: its size depends on input strength, the initial membrane potential and the receiving cell membrane's properties. Local voltage changes can decay before reaching the soma; their timing and overlap help determine whether an action potential follows. See Ion Channels and the Electrical Properties of Membranes.
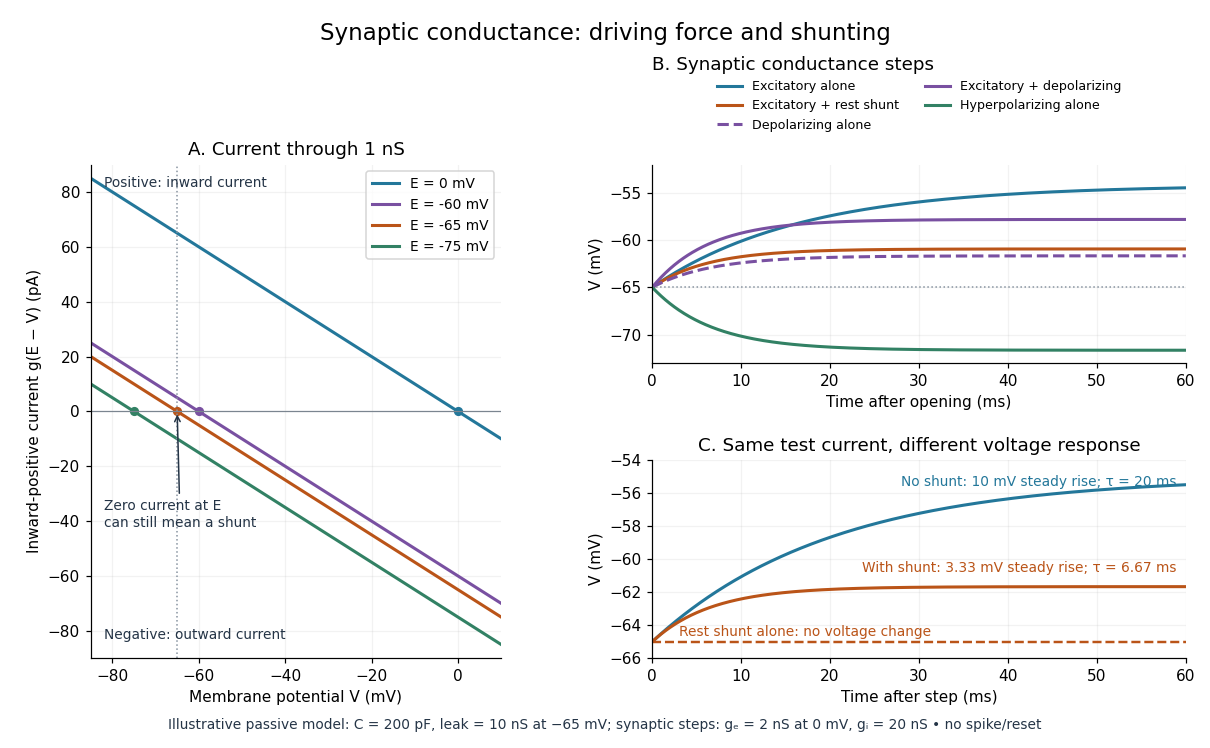
Depolarization means that the interior becomes less negative relative to the exterior; hyperpolarization means that it becomes more negative. Excitation and inhibition instead describe whether an input promotes or opposes postsynaptic action potential generation. An inhibitory postsynaptic potential can be depolarizing, and shunting inhibition can occur with no voltage change at rest. The receptor, permeating ions, ionic gradients and reversal potential matter. See Purves and colleagues: excitation, inhibition and depolarizing inhibition.
A worked passive model treats the receiving membrane as one compartment with capacitance , leak conductance , and activated synaptic conductances :All electric currents are inward-positive. Each term vanishes at its reversal potential ; . With constant parameters, the ordinary differential equation hasHere is total conductance, is effective electrical resistance, is the steady state and the time constant. Without imposed electric current, is a conductance-weighted average of the reversal potentials. This approximation omits spatial structure, changing ionic gradients and active voltage-gated ion channels; it calculates passive voltage responses, not actual action potential waveforms. See 3.1 Synapses for the mechanism behind the terms; the inward-positive convention here reverses that source's synaptic-current sign.
Take the same illustrative leak and capacitance as under shunting inhibition, start at and set . Opening with gives and . Its initial inward electric current is . Adding with changes to and . This is shunting inhibition of the same excitatory drive.
For comparison, with alone gives : hyperpolarization. With instead, it alone gives : depolarization. Yet adding this depolarizing conductance to the excitatory drive lowers that drive's from to . At an illustrative firing threshold , its electric current is , opposing threshold approach. The combined trace initially rises faster than the excitatory drive alone, before settling below it. Thus the sign of a voltage change at rest alone does not determine excitation or inhibition; a claim about firing must specify input strength, timing and the neuron's state.
An electrical synapse passes ionic electric current directly between neurons through gap junctions, whose paired channels connect the two cytoplasms. It does not require synaptic vesicle release and postsynaptic neurotransmitter binding. Transmission across the junction is very fast; the receiving cell membrane's capacitance and other conductances still determine its voltage response. Electrical coupling can coordinate the timing of activity across neurons. See Purves and colleagues: electrical synapses and gap junctions.
For a passive junction with constant conductance , the inward electric current into cell 2 iswhere each is the cell's membrane potential, measured against a common extracellular reference. Taking , and gives into cell 2 and the equal opposite electric current into cell 1. Exchanging the voltages reverses the electric current. Both depolarization and hyperpolarization can therefore be transmitted; an electrical synapse is not inherently an excitatory connection.
Many electrical synapses conduct in both directions, but this does not guarantee equal voltage responses: the cells can have different effective electrical resistance and capacitance. Some junctions rectify, meaning they conduct preferentially in one direction, so the constant- formula is insufficient. A concrete molecular example is the original study [ref]
https://pmc.ncbi.nlm.nih.gov/articles/PMC7455501/. Shui and colleagues, 2020: Molecular basis of junctional current rectification at an electrical synapse
. Bidirectionality is thus a common property with important qualifications, rather than part of the definition.A chemical synapse transmits a signal by releasing neurotransmitter from a presynaptic neuron to act on postsynaptic receptors across a synaptic cleft. The two cell membranes remain separate. A typical fast transmission sequence is:
- An arriving action potential produces presynaptic depolarization, opening voltage-gated ion channels selective for calcium.
- Calcium ions enter down their electrochemical gradient. The local rise in calcium concentration activates release machinery, allowing already prepared synaptic vesicles to fuse with the presynaptic cell membrane by exocytosis.
- Released neurotransmitter crosses the synaptic cleft by diffusion and binds postsynaptic receptors.
- Ionotropic receptors directly gate an ion channel; metabotropic receptors activate an intracellular signaling pathway that can alter ion channels indirectly. Changed synaptic conductance changes electric current and usually produces a synaptic potential.
See Chemical Synapses and 3.1 Synapses. The fast pathway uses synaptic vesicles prepared near release sites; it does not require a distant synaptic vesicle to travel across the terminal after every action potential. See Basic Neurochemistry: calcium entry and vesicles at release sites. Some chemical synapses release neurotransmitter in response to graded presynaptic membrane potential changes rather than action potentials.
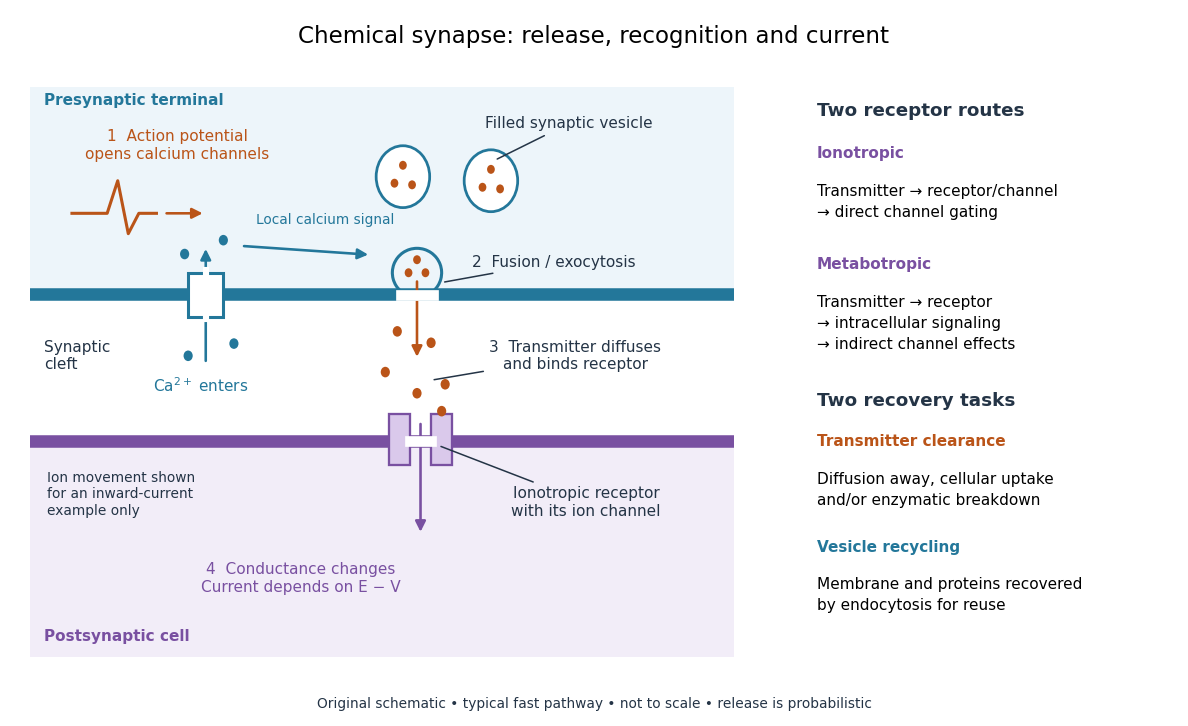
Neurotransmitter clearance limits how long released neurotransmitter remains available. Depending on the neurotransmitter and location, diffusion away, uptake through membrane transport proteins into the sending or neighboring biological cells, and breakdown by enzymes contribute. Receptor binding and unbinding also affect response duration. Recovering synaptic vesicle membrane is a separate recycling task; uptake of released neurotransmitter is not the return of an intact synaptic vesicle. See General Principles of Cell Communication.
This electrical-to-chemical-to-electrical sequence offers several places to adjust a signal: synaptic release probability, receptor availability and neurotransmitter clearance can change its strength or duration. It helps explain why synaptic plasticity can modify communication between neurons, and why an arriving action potential need not cause a postsynaptic action potential.
Otto Loewi's 1936 Nobel lecture describes his 1921 experiment: fluid from a frog heart whose nerves had been stimulated produced the corresponding response when transferred to another heart. The transferable substance established chemical mediation in that preparation. This was evidence for released chemical signaling, not yet an identification of synaptic vesicle fusion and not a claim that every synapse is chemical. See Loewi, The Chemical Transmission of Nerve Action, Nobel lecture, 12 December 1936.
Here is a product of power-sum symmetric functions and for part multiplicities . The Frobenius characteristic map identifies this product with the ordinary character inner product. Schur functions are orthonormal, and the adjoint of multiplication by is . These properties turn a power-sum multiplication formula into the Murnaghan–Nakayama rule.
For an integer partition , sums the distinct monomials whose positive exponent multiset is . No multiplicity is attached to repeated parts. The functions of fixed total degree form a basis of the symmetric functions of that degree, since finite variable permutations identify precisely these monomial orbits.
The Fundamental theorem of symmetric polynomials gives freely generated elementary functions, so sending each to defines an algebra homomorphism. For and , . Applying the homomorphism shows , hence . Taking logarithms of gives the displayed action on power sums. It preserves the Hall inner product of symmetric functions because each power-sum basis vector acquires only a sign.
Expand each factor as a geometric series indexed by a nonnegative matrix. The RSK correspondence preserves its row and column contents, changing the sum to pairs of Semistandard Young tableaux of the same shape and proving the displayed formal identity. Its kernel is also . These are dual-basis kernels for the Hall inner product of symmetric functions, so the Schur expansion proves orthonormality. Applying the symmetric-function involution in one alphabet gives the dual identity .
Relative survival compares observed survival in a diseased cohort with expected survival derived from a suitable reference population. A useful individual model adds a known background mortality hazard to a common excess hazard. Reference mortality can depend on age, sex and calendar time. The comparison avoids classifying each death by cause, but its interpretation depends on the reference population being appropriate. An excess-survival ratio is not automatically the effect of a causal intervention removing one cause of death.
Survival data describe the time from a specified origin to an event, together with covariates and the observation mechanism. Under right censoring, the observed exit time is and the event indicator is . With left truncation, an entry time is also recorded and subjects are observed only if . Recording the time origin, entry, exit and event indicator is essential for constructing valid risk sets.
A cure model mixes an individual class with identically zero hazard function and a susceptible class with survivor function . For , its representation as a proportional frailty model with is with probability and otherwise, with baseline hazard . The frailty law is a mixture of two Dirac measures, rather than an ordinary density. Its Laplace transform evaluated at gives the displayed survivor function. The limiting survival equals when ; otherwise the plateau also includes susceptible individuals who never experience the event.
For a broad, thin oil lens below a flat ice-water interface, define the effective interfacial energy from the relevant surface tensions. At fixed oil volume , the energy is . Setting its derivative to zero gives for , and the positive second derivative proves a minimum. A contact angle measured through the oil gives . Oil-ice tension alone does not determine this effective quantity. Complete wetting or rough underside pockets invalidate this finite, flat-lens approximation. With densities and , a lens below requires .
The Bond number compares hydrostatic stress over a length with capillary stress. For a gas bubble of radius and negligible density, . Small Bond number is the usual sufficient criterion for capillarity to resist gravity-scale deformations. For a clean spherical bubble with negligible internal dynamic viscosity settling in creeping flow, the capillary number is . This last relation uses the clean-bubble terminal velocity; it does not apply at arbitrary Reynolds number or to an interface immobilized by surfactants.
Wetting describes how a liquid maintains contact with or spreads over a solid in the presence of another phase, usually a gas. The competition among solid-liquid, solid-gas and liquid-gas interfacial free energies determines the equilibrium contact angle. For an ideal smooth homogeneous surface, Young's contact-angle equation giveswith measured through the liquid.
A small water drop that spreads over clean glass but beads on a water-repelling surface provides a simple comparison. A low contact angle indicates stronger spreading within this partial-wetting description; complete spreading requires considering the associated interfacial free-energy change. Surface roughness, contamination and contact-angle hysteresis can make the observed angle depend on preparation and whether the contact line is advancing or receding, so one photograph need not determine an equilibrium material constant.
For a liquid interface with constant surface tension , the mechanical surface energy is the energy associated with its surface area :The additive constant does not affect the work needed to change surface area. For several interfaces with the same surface tension, means their total surface area; the two faces of a thin soap film must both be counted. [ref]
https://arxiv.org/html/2011.11403v2. Tomas Bohr and Bernhard Scheichl, Surface Tension and Energy Conservation in a Moving Fluid, equation (13)
With assumed , creating of one interface requires of reversible work. In the sliding-rim example illustrated under surface tension, moving a rim outwards by creates across the two faces and requires . Independently, multiplying its holding force by the displacement gives the same work.
This makes the preference for a round isolated droplet precise. At fixed volume , the three-dimensional isoperimetric inequality giveswith equality for a sphere. Thus a sphere minimizes surface energy among sufficiently regular closed shapes enclosing the same volume, when surface tension is uniform and other energy contributions are negligible. This is an application of the isoperimetric inequality, rather than a proof of it. Walls, wetting, and gravity can change the shape by adding constraints or other energy contributions. [ref]
https://math.hmc.edu/funfacts/isoperimetric-inequality/. Francis E. Su et al., Isoperimetric Inequality, Math Fun Facts
The differential rule integrates directly to because surface tension is constant. At fixed liquid volume, decreasing surface area can drive viscous fluid flow; the released surface energy can supply viscous dissipation. This mechanical bookkeeping is useful for predicting which deformations can release energy. If surface tension depends on temperature or composition, distinguish this mechanical area-work relation from the complete interfacial thermodynamic free energy and internal energy.
Dynamical supersymmetry breaking occurs when quantum dynamics produces a vacuum that does not preserve supersymmetry. An asymptotically free hidden sector can generate the displayed exponentially small scale through dimensional transmutation. This supplies a possible origin of a hierarchy, but strong coupling by itself does not prove breaking: the vacuum equations and dynamics must exclude a supersymmetric vacuum.
// Target: supersymmetry.bigb
Pinned article: Introduction to the OurBigBook Project
Welcome to the OurBigBook Project! Our goal is to create the perfect publishing platform for STEM subjects, and get university-level students to write the best free STEM tutorials ever.
Everyone is welcome to create an account and play with the site: ourbigbook.com/go/register. We belive that students themselves can write amazing tutorials, but teachers are welcome too. You can write about anything you want, it doesn't have to be STEM or even educational. Silly test content is very welcome and you won't be penalized in any way. Just keep it legal!
Intro to OurBigBook
. Source. We have two killer features:
- topics: topics group articles by different users with the same title, e.g. here is the topic for the "Fundamental Theorem of Calculus" ourbigbook.com/go/topic/fundamental-theorem-of-calculusArticles of different users are sorted by upvote within each article page. This feature is a bit like:
- a Wikipedia where each user can have their own version of each article
- a Q&A website like Stack Overflow, where multiple people can give their views on a given topic, and the best ones are sorted by upvote. Except you don't need to wait for someone to ask first, and any topic goes, no matter how narrow or broad
This feature makes it possible for readers to find better explanations of any topic created by other writers. And it allows writers to create an explanation in a place that readers might actually find it.
Figure 1. Screenshot of the "Derivative" topic page. View it live at: ourbigbook.com/go/topic/derivativeVideo 2. OurBigBook Web topics demo. Source. - local editing: you can store all your personal knowledge base content locally in a plaintext markup format that can be edited locally and published either:This way you can be sure that even if OurBigBook.com were to go down one day (which we have no plans to do as it is quite cheap to host!), your content will still be perfectly readable as a static site.
- to OurBigBook.com to get awesome multi-user features like topics and likes
- as HTML files to a static website, which you can host yourself for free on many external providers like GitHub Pages, and remain in full control

Figure 2. You can publish local OurBigBook lightweight markup files to either OurBigBook.com or as a static website.
Figure 3. Visual Studio Code extension installation.
Figure 5. . You can also edit articles on the Web editor without installing anything locally. Video 3. Edit locally and publish demo. Source. This shows editing OurBigBook Markup and publishing it using the Visual Studio Code extension. 
- Infinitely deep tables of contents:




All our software is open source and hosted at: github.com/ourbigbook/ourbigbook
Further documentation can be found at: docs.ourbigbook.com
Feel free to reach our to us for any help or suggestions: docs.ourbigbook.com/#contact