
A diffusion cloud chamber continuously supplies vapor from a warmer reservoir toward a colder base. A temperature gradient permits supersaturated vapor in a layer near the base, where new ionization trails can continually form drops. There is no repeated bulk piston expansion cycle. The two instruments share ion-assisted condensation, but their sensitive regions and timing differ.
CERN's modern teaching apparatus uses alcohol-soaked felt, a sealed transparent container, a dark metal base cooled with dry solid carbon dioxide, and a side light. The view is a thin sensitive region near the cold base, rather than a chamber-wide expansion photograph.[ref][ref]
Bringing Particle Physics to Life: Build Your Own Cloud Chamber by Francisco Barradas-Solas and Paloma Alameda-Meléndez. Barradas-Solas and Alameda-Meléndez, Bringing particle physics to life: build your own cloud chamber (29 April 2010), “The continuously sensitive diffusion cloud chamber” and “Method”, steps 5–6
The central mechanism is a competition between two falling pressures: expansion reduces the actual water partial pressure, but cooling can reduce the equilibrium vapor pressure still faster. The ratio can therefore rise above one even though the gas becomes more dilute. The cloud-chamber expansion model below makes that comparison explicit.
A climate model is a mathematical description of the mechanisms and statistics of a planet's climate change and variability. A useful hierarchy starts with conservation of energy in a zero-dimensional planetary energy balance, adds vertical radiative transfer and convection in a radiative-convective climate column, and can resolve three-dimensional fluid mechanics and ocean circulation. Each level answers different questions. A column can explain why changing an absorber changes surface temperature; it cannot locate tomorrow's storm.
Three questions should be kept distinct: what sets an average temperature, how fast does it respond to radiative forcing, and how large are its unforced fluctuations? Climate sensitivity concerns the first, heat capacity controls response times, and the Hasselmann stochastic climate model illustrates the third. An observational test must compare a predicted observable with an instrument's actual readout, as in the satellite test of greenhouse spectral change.
Hans Adolf Krebs described the experimental reasoning in his 1953 Nobel lecture. Pigeon breast skeletal muscle retained strong oxidative activity after preparation in a Latapie mincing mill and suspension in aqueous medium. Small fumarate additions increased oxygen uptake by more than complete oxidation of the added fumarate could explain; added four-carbon acids could still be detected afterward. His Table 1 compares the increase in uptake with that calculated from complete consumption of the addition. These comparisons challenge the interpretation that the addition merely supplied extra fuel.[ref]
The citric acid cycle by Hans Adolf Krebs. The citric acid cycle, Nobel Lecture, 11 December 1953, printed pp. 400–401 and Table 1: minced-muscle preparation, uptake comparison and retained acid; authored transcript also available at studyres.com/doc/1333386/hans-a.-krebs---nobel-lecture
The lecture identifies the preparation apparatus but does not describe the gas-measuring instrument behind Table 1. The result supports regeneration, not a unique complete reaction mechanism. Its later discussion combines citrate formation from oxaloacetate with breakdown back toward the four-carbon intermediates to close the cycle. Competitive inhibition supplies another comparison: malonate inhibits succinate dehydrogenase, and succinate accumulates. Such evidence links a blocked step to the surrounding metabolic pathway; damaged tissue and restricted inhibitor access can complicate interpretation.[ref]
The citric acid cycle by Hans Adolf Krebs. The citric acid cycle, printed pp. 401–404, Figures 1–2 and malonate discussion: cyclic interpretation and inhibitor-access limitation; p. 399, preparation damage
An increase above the added fuel's own oxygen demand is a particularly revealing control on the explanation: it compares the proposed cause with the largest effect that simple consumption could produce. The modern mitochondrial oxygen electrode assay asks a different question about a prepared mitochondrion, testing respiratory control through ADP additions. Neither an oxygen uptake signal nor an accumulating intermediate is by itself a direct measurement of ATP production.
Net stoichiometry does not identify individual chemical atoms. In the ordinary forward citric acid cycle, neither entering acetyl group carbon is released in that same first turn: both released carbon dioxide carbon chemical atoms came from the starting oxaloacetate. The entering carbon remains in regenerated intermediates.[ref]
The Citric Acid Cycle (Boston University lecture slides). The Citric Acid Cycle, slide numbered 4, Origin of C-Atoms in CO2: entering acetyl carbons retained and released carbons from starting oxaloacetate
Consider a chosen ideal first-turn experiment, with negligible natural carbon-13 abundance and no exchange, side pathways, repeated turns or isotope effects. Supply of initially unlabelled oxaloacetate and of acetyl-CoA, of which has both acetyl group carbon positions labelled with carbon-13. The other has neither position labelled. The label refers only to the acetyl group, not to coenzyme A.
The input contains of labelled carbon chemical atoms. The of citrate initially formed contains of carbon chemical atoms, so its labelled-carbon fraction is . After exactly one forward traversal per starting oxaloacetate, the of released carbon dioxide has zero label, while the regenerated of oxaloacetate contains all of labelled carbon chemical atoms among total: .
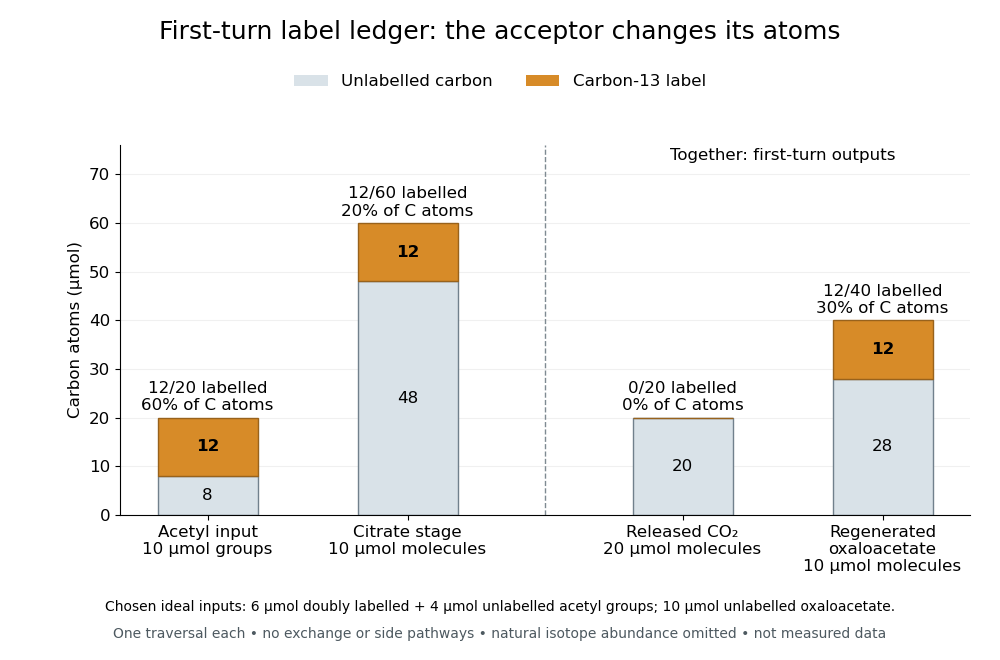

The conservation check is for total carbon and for label. In this model, of regenerated oxaloacetate molecules carry label, distinct from the labelled-carbon fraction. The regenerated oxaloacetate is the same chemical species and the same amount of substance as the initial acceptor pool, but its chemical atom identities have changed. Saying that the cycle oxidizes an acetyl group to two carbon dioxide is a net ledger, not a claim that those exact two incoming chemical atoms immediately leave. Later-turn label release requires positional tracking and mixing assumptions; the first-turn balance alone does not determine it.
The carbon sequence is oxaloacetate plus an acetyl group to citrate , then isocitrate , alpha-ketoglutarate , succinyl-CoA , succinate , fumarate , malate and back to oxaloacetate . The numbers count the cycling carbon skeleton, excluding coenzyme A. Two carbon dioxide releases accompany the changes .[ref]
Biology 2e by Mary Ann Clark and others. §7.3, Steps in the Citric Acid Cycle, steps 1–8 and Figure 7.11
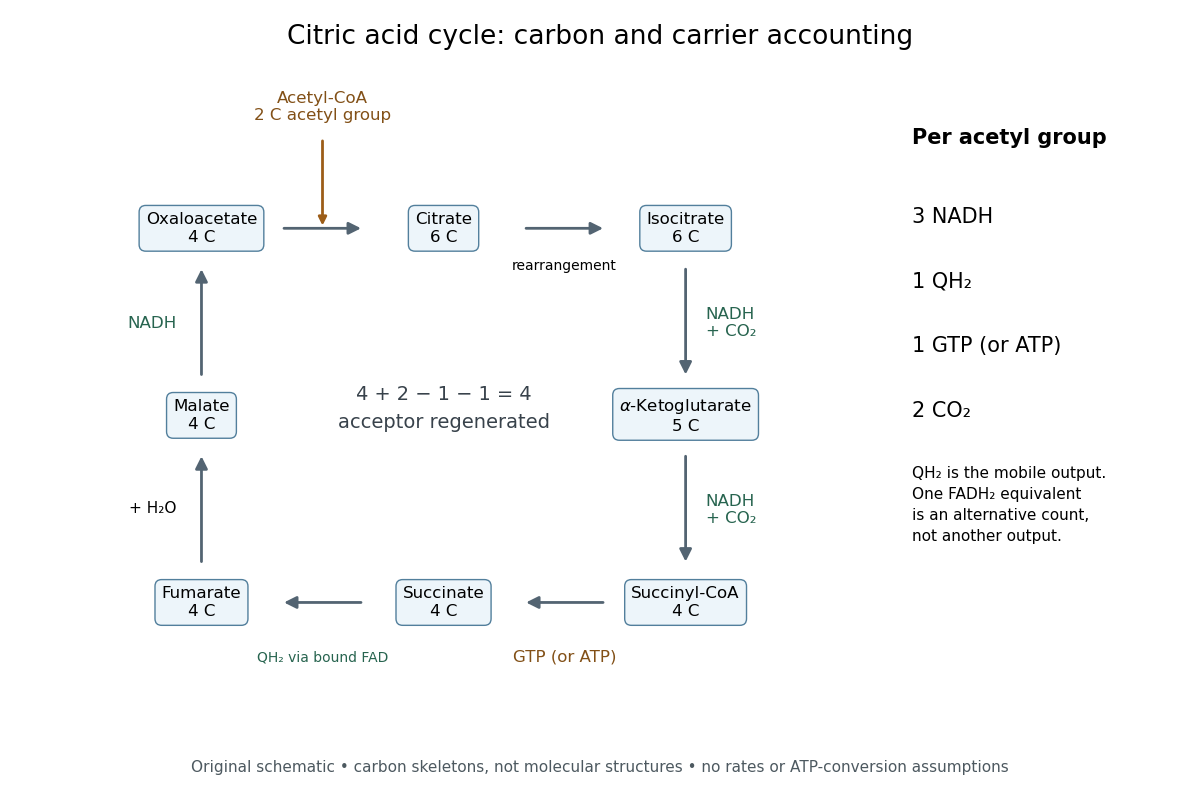

Per acetyl group: three NADH, one FADH2 equivalent, one GTP or ATP by substrate-level phosphorylation, and two carbon dioxide. Succinate dehydrogenase retains FADH2 and transfers its electrons to ubiquinone, forming ubiquinol. The FADH2 equivalent and ubiquinol count the same electron pair.[ref]
Biology 2e by Mary Ann Clark and others. §7.3, Citric Acid Cycle and Steps in the Citric Acid Cycle, steps 3–8, especially step 6, enzyme-bound reduced carrier; §7.4, Q and Complex II: ubiquinone reduction to QH2
A useful check adds the stepwise changes. The carbon count is ; the NADH count is . Each NADH carries two electrons, and the succinate dehydrogenase route supplies another pair, so one turn exports electrons. This arithmetic is an accounting identity, not an ATP yield calculation. Converting it to ATP requires the separate energy coupling and transport assumptions discussed under oxidative phosphorylation.
For a chosen ideal conversion of of acetyl groups, multiplication gives of NADH, of ubiquinol, of GTP and of carbon dioxide. The electron output is . If all these electrons subsequently reach oxygen with no competing sinks, four electrons per oxygen molecule require of oxygen. That is consumption by the connected electron transport chain; it is not an oxygen term in the cycle's own substrate ledger.
No cycle step directly consumes molecular oxygen. In ordinary aerobic mitochondrial operation, however, the mitochondrial respiratory chain must reoxidize NADH and ubiquinol to restore the oxidized electron carriers. Without that outlet, a finite oxidized-carrier pool cannot sustain continued turnover. Other electron acceptors and other forms of metabolism require their own analysis.[ref]
How Cells Obtain Energy from Food. Molecular Biology of the Cell, 4th edition by Bruce Alberts and others; Chapter 2, How Cells Obtain Energy from Food, The Citric Acid Cycle Generates NADH by Oxidizing Acetyl Groups to CO2: lack of direct O2 consumption and need to regenerate NAD+
The pyruvate dehydrogenase complex acts upstream: one three-carbon pyruvate gives one two-carbon acetyl group, one carbon dioxide and one NADH. These are additional to the cycle ledger.[ref] Consequently, processing one pyruvate through both stages gives three carbon dioxide and four NADH, while the succinate dehydrogenase contribution and the substrate-level phosphorylation contribution each remain one. Counting the upstream step inside the cycle would obscure where the extra carbon dioxide and NADH arise.
The signed accumulated rotation about a specified fixed axis. Unlike an angle specified only modulo , angular displacement counts complete revolutions as well as the final orientation. Its derivative with respect to time is angular velocity. The displayed formula therefore follows from the fundamental theorem of calculus.
An arithmetic circuit is a directed acyclic graph whose input nodes are variables or constants in a field, and whose internal gates perform addition, subtraction, or multiplication. Gates may reuse earlier outputs, so the circuit can represent a polynomial without listing all its monomials.
The space between the two chloroplast envelope membranes.
It is topologically distinct from both the chloroplast stroma and the thylakoid lumen. Naming the compartments prevents a transport measurement across one barrier from being mistaken for transport across the entire chloroplast membrane system. [ref]
Molecular Biology of the Cell, 4th edition by Bruce Alberts and others. Chapters 12, 18 and 19, compartments, division and cell junctions
Separates chloroplast intermembrane space from chloroplast stroma.
Its selective transport systems help maintain the distinct composition of the chloroplast stroma. The thylakoid membrane is a separate internal membrane, so an imported molecule reaching the stroma has not automatically reached the thylakoid lumen. [ref]
Molecular Biology of the Cell, 4th edition by Bruce Alberts and others. Chapters 12, 18 and 19, compartments, division and cell junctions
Separates surrounding cytosol from chloroplast intermembrane space.
Together with the inner chloroplast envelope membrane, it defines the boundary of the chloroplast. Crossing the envelope and entering the thylakoid lumen are different transport problems because the thylakoid system supplies an additional membrane barrier. [ref]
Molecular Biology of the Cell, 4th edition by Bruce Alberts and others. Chapters 12, 18 and 19, compartments, division and cell junctions
There are unlisted articles, also show them or only show them.