Past exam of the zoology course of the University of Cambridge 2025 Paper zl6 6 a Solution by  Codex 0 2026-10-20
Polarity proteins generate tissue form by controlling where cells build surfaces, place junctions and divide. Their morphogenetic roles can be separated experimentally from a wholesale loss of epithelial identity. Three examples illustrate different outputs: positioning a single lumen, orienting neighbour exchange, and limiting tube dimensions.
The first example is Cdc42-dependent lumen formation in three-dimensional Caco-2 epithelial cysts. Cells in a normal cyst coordinate their apical-basal polarity so that apical surfaces face one central lumen. During growth, a correctly oriented spindle apparatus places daughter cells into the epithelial wall rather than establishing inappropriate internal cell arrangements. Cdc42 depletion disrupts spindle orientation and produces abnormal, often multiple, luminal spaces. Importantly, the cells can still establish apical membrane identity: in this model the crucial defect is the coordination and positioning of apical surfaces during division, rather than an absolute inability to make any apical surface. This distinguishes tissue-level organization from polarity within an isolated cell.[ref]
Cdc42 controls spindle orientation to position the apical surface during epithelial morphogenesis by Aron B. Jaffe and others. Caco-2 three-dimensional cysts, Cdc42 depletion and spindle-orientation analysis
Mechanistically, Cdc42 connects cortical organization to the PAR polarity complex, polarized trafficking and spindle-positioning machinery. However, the relative contributions depend on the model: a Cdc42 trafficking phenotype in another epithelial line cannot simply be substituted for the Caco-2 spindle result. A convincing test combines live-cell imaging of division and the first ectopic lumen with apical and basal markers, verifies target depletion and rescues with functional Cdc42. Compare the total number and viability of cells, because a dying cell population can also produce abnormal cavities. A perturbation that restores spindle positioning while leaving other outputs of Cdc42 impaired would help isolate the causal route. These controls make the single-lumen phenotype an interpretable morphogenetic output.
The second example is Bazooka, the fly PAR-3 protein, during Drosophila germband extension. This uses planar cell polarity within the epithelial sheet as well as apical-basal organization. Bazooka and junctional components become enriched at a complementary set of cell interfaces to myosin II. Spatially patterned gene activity organizes this planar asymmetry, and loss of Bazooka disrupts normal polarized cell behaviour and extension. Thus a protein associated with epithelial junction assembly is redeployed to make different junctions behave differently in the same sheet.[ref]
Patterned gene expression directs bipolar planar polarity in Drosophila by Jennifer A. Zallen and Eric Wieschaus. Planar distributions of Bazooka and myosin and dependence on patterned gene expression
Oriented junction shrinkage and new-junction formation permit cell intercalation while maintaining epithelial continuity. The important geometry is that junctions separating anterior and posterior neighbours shrink and resolve into interfaces with the complementary orientation, producing extension along the body axis. Junction names can be confusing because they may describe either the neighbours or the line itself; tracking vertices and neighbour exchange avoids this ambiguity. Bazooka is a spatial organizer, not itself the force-generating motor. To test its contribution, quantify its localization, myosin localization, junction lifetimes, cell rearrangements and tissue strain after an acute or mosaic perturbation that leaves enough epithelial structure for movement to occur. A general epithelial collapse would establish an essential structural role but would not isolate its role in planar coordination.
The third example is control of fly tracheal tube size by the apical determinant Crumbs and basolateral regulators including Yurt and Coracle. Crumbs promotes the apical domain, so restricting its activity helps constrain the amount of luminal cell surface and hence tube dimensions. Mutations in yurt produce overlong tracheal tubes, and reducing Crumbs dosage suppresses important length defects; Crumbs overexpression has the opposite tendency. This genetic interaction connects the balance of apical and basolateral regulators to organ geometry rather than simply to the presence of an epithelial sheet.[ref]
Epithelial polarity proteins regulate Drosophila tracheal tube size in parallel to the luminal matrix pathway by Patrick Laprise and others. Tube measurements, Crumbs dosage suppression and Vermiform secretion controls
The luminal extracellular matrix is a crucial control in this example. Septate-junction-associated proteins can also affect delivery of the matrix-modifying protein Vermiform, potentially changing tube shape indirectly. Yet yurt mutants retain Vermiform secretion, and reducing Crumbs can suppress coracle length defects without restoring the secretion defect. Scribble mutants also show long tubes but are not equivalently rescued by the tested Crumbs reduction. The result supports parallel and partly distinct routes, rather than a universal linear pathway in which every basolateral protein merely inhibits Crumbs. Compare cell number, apical area, tube length and diameter independently: a longer tube need not result from extra divisions. Quantitative dosage interactions and rescue are particularly informative because they can reveal a size-control function while preserving much of epithelial organization.
Together, these examples link polarity to three separable operations. Cdc42 coordinates the location of new apical surfaces during division; Bazooka contributes to directional junction remodelling within a sheet; and the Crumbs-regulator balance sets the extent of a luminal surface. Conversely, changing forces and geometry can alter junctional organization, so the relationship is reciprocal. The common principle is that epithelial polarity supplies spatial constraints on growth and rearrangement. It is a dynamic component of morphogenesis, not merely a static property to be established before morphogenesis starts.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl6 3 b Solution by Codex 0 2026-10-20
Codex 0 2026-10-20reactive oxygen species can alter competitive fitness, but neither high ROS nor an antioxidant response universally identifies a loser. cell competition is relative: cells that survive in one neighbourhood are preferentially lost in another, with fitter neighbours occupying their place. An experiment showing oxidant-induced death in a homogeneous tissue establishes toxicity, not necessarily cell competition. In epithelia, loss can occur through apoptosis, extrusion or differentiation followed by departure from a proliferative layer.
reactive oxygen species include superoxide and hydrogen peroxide, which differ in reactivity, localization and transport. They can arise from mitochondrial metabolism or regulated oxidase activity. At controlled levels they participate in redox signalling; excess or poorly buffered production damages DNA, proteins and membranes. Competitive fitness can therefore change through altered damage, stress responses, growth or differentiation. NRF2 and its fly counterpart CncC regulate antioxidant and detoxification programmes. Their activation is an integrated response to cellular conditions, not a direct quantitative measurement of one ROS species.
An instructive fly study compared prospective losers carrying a ribosomal-protein defect or loss of Mahjong protein. Both activated antioxidant-response genes before elimination. In ribosomal-protein-deficient cells, two ROS dyes did not reveal a uniform increase, whereas reduced-thiol staining was lower. Mild CncC activation was tolerated across an entire disc but caused boundary-enriched death in clones surrounded by normal cells; those clones survived better among less-fit neighbours. Conversely, reducing CncC impaired stressed-cell survival. Thus a protective response can also confer relative loser status. The study separated this module from JNK signalling effects on growth and from JAK-STAT signalling effects on tissue expansion; it did not establish a compulsory linear chain from ROS through JNK to elimination.[ref]
Chronic activation of JNK JAK/STAT and oxidative stress signalling causes the loser cell status by Iwo Kucinski and others. Figures 5–7, redox measurements and neighbourhood-dependent CncC experiments
This distinction prevents two errors. First, a high antioxidant-response reporter can coexist with successful buffering and relatively low measured oxidant levels. Second, knocking down a protective factor may kill cells autonomously, making their apparent competitive loss worse even if that factor also participates in neighbour-dependent recognition. To identify a competitive mechanism, compare the same genotype in a homogeneous tissue, in a mosaic with normal neighbours and in a mosaic with an alternative neighbour genotype. Quantify clone growth, death at boundaries and in centres, and replacement by neighbours, normalized to the corresponding cell numbers or areas. A clone that is small because its cells divide slowly has not necessarily been actively eliminated.
The adult mammalian oesophagus supplies a striking environmental example. In transgenic mouse epithelium, low-dose ionizing radiation induced an oxidative response that shifted normal basal cells toward differentiation. Cells carrying mutant p53 were relatively insensitive and expanded at their neighbours' expense. Combining antioxidant treatment with irradiation reversed the population outcome, promoting normal-cell proliferation and mutant-cell differentiation. The selective advantage was consequently conditional on the redox environment, not a fixed property of the mutation. This also shows that competitive replacement need not be executed primarily by apoptosis.[ref]
A separate mouse experiment generated a mosaic of NRF2-deficient and NRF2-intact oesophageal cells. Deficient cells persisted under unstressed conditions but accumulated damage and were preferentially lost during exposure to the carcinogen 4-nitroquinoline 1-oxide. Tumours predominantly arose from the surviving NRF2-intact population. This supports a context-dependent role for stress protection in population selection, while not proving that every disappearing cell was directly recognized and killed by a neighbour. Carcinogen detoxification and DNA damage are additional variables, so the experiment is not a chemically pure ROS titration.[ref]
Cellular Nrf2 Levels Determine Cell Fate during Chemical Carcinogenesis in Esophageal Epithelium by Makoto Horiuchi and others. Mosaic deletion, unstressed controls and 4NQO exposure experiments
To test a proposed ROS mechanism in an epithelial mosaic, image a calibrated, compartment-targeted redox biosensor before clone loss, along with cell boundaries, a proliferation readout and a death or differentiation reporter. Include sensor controls for pH, expression level and dynamic range; general oxidant dyes have loading, localization and chemical-specificity limitations. Perturb the source and scavenging machinery independently and restrict the perturbation to prospective losers or winners. For example, a validated catalase manipulation tests peroxide buffering, while a source-specific perturbation tests whether that peroxide is required. A matched rescue should restore both the measured redox change and the competitive outcome. Monitor cellular energy and survival in homogeneous controls because a mitochondrial perturbation can affect fitness independently of ROS. Perturb downstream stress signalling separately to distinguish oxidant production, stress detection and execution of cell loss.
The tissue consequences can be beneficial or harmful. Elimination of damaged cells can preserve a barrier, but a stress-resistant mutant can also exploit environmental oxidants to displace normal cells. Persistent stress signals from damaged or dying cells may alter neighbour proliferation and inflammation, producing further changes in fitness. The experimentally supported conclusion is that redox state reshapes the conditions under which cells persist, differentiate or are eliminated. A universal prescription to raise ROS or administer antioxidants does not follow: the relevant species, tissue compartment, neighbour genotype and exposure history determine the direction of selection.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl6 3 a Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Epithelial cell fate plasticity is a context-dependent change in developmental potential or differentiated identity. It includes dedifferentiation toward a progenitor cell state, transdifferentiation between differentiated identities, and reversible intermediate states. It is distinct from selecting a pre-existing rare stem cell, and from ordinary progression down a lineage. epithelial-mesenchymal plasticity is one important form, but changing epithelial subtype without losing epithelial organization is also cell fate plasticity.
The strongest physiological rationale is that a tissue needs both stable specialization and reserve routes for replacement. During ordinary adult tissue homeostasis, a stem-cell hierarchy can efficiently supply predictable cell types. After injury removes a component of that hierarchy, local signals and newly available stem-cell niche space may permit a committed descendant to reacquire self-renewal. In mouse intestine, Alpi marked enterocyte-lineage progenitor cells normally generate short-lived absorptive descendants. After targeted ablation of Lgr5 positive intestinal stem cells, labelled progenitor cells can generate long-lived crypt-villus lineages with renewed stem-cell output. Comparing the same labelled population before and after ablation distinguishes injury-dependent cell fate plasticity from its normal fate. The experiment concerns progenitor cells in the enterocyte lineage; it should not be generalized to every terminally mature villus enterocyte.[ref]
A complementary model is the mouse airway. Genetic depletion of basal stem cells, combined with prior lineage tracing of luminal secretory cells, revealed secretory-cell descendants that acquired basal-cell properties and sustained subsequent epithelial production. Experiments with isolated cells and cocultures further showed that contact with basal cells inhibits this conversion. cell fate plasticity is therefore regulated by the tissue environment, not simply an intrinsic capacity unmasked whenever a marker changes. Its interpretation requires controls for residual basal cells and for whether the secretory-lineage driver labelled basal cells before injury.[ref]
Dedifferentiation of committed epithelial cells into stem cells in vivo by Purushothama Rao Tata and others. Basal-cell ablation, secretory-cell lineage tracing and contact-dependent suppression
Development provides additional contexts. Embryonic epithelia can undergo epithelial-to-mesenchymal transition during processes such as gastrulation, and mesenchymal-to-epithelial transition can subsequently assemble epithelial structures. These are regulated changes in adhesion, cell polarity, motility and gene expression, rather than a simple binary switch read from E-cadherin alone. In wound repair, transient relaxation of epithelial organization can facilitate migration while retaining intercellular contacts. A partially migratory repair state need not entail a complete mesenchymal conversion or a permanent change of lineage. Following wound closure, restoration of barrier function and polarized architecture is as important as the initial ability to move.
The most convincing experimental design labels a defined starting population irreversibly before the inducing event, allows the inducer to clear, then follows labelled descendants through the transition. Check immediate labelling specificity, include no-inducer and uninjured controls, quantify labelling efficiency and rule out ectopic driver activation after injury. Demonstrate the new state with multiple markers, morphology and function, and persistence after the inducing signal is removed. Serial epithelial production or a second injury challenge tests stable self-renewal; a transient appearance of a basal marker does not. Sparse labelling and continuous live-cell imaging help distinguish conversion from contamination, cell fusion or selective expansion of a rare initially unrecognized progenitor cell.
single-cell RNA sequencing can identify intermediate cell states and candidate regulators, but inferred trajectories are not lineage histories. Combine it with genetic barcodes, spatial localization and timed perturbation of candidate transcription factors or niche signals. Organoids offer defined media, prospective cell isolation and manipulation of matrix stiffness. A sorted population's ability to make a structure in culture establishes potential under those conditions; dissociation and a permissive medium may induce a capacity rarely used in vivo. Compare culture results with intact-tissue fate mapping before claiming a normal physiological contribution.
The evolutionary argument is a trade-off, rather than a claim that every plastic response is an adaptation. Conditional access to alternative cell fates could buffer environmental injury and permit repair without maintaining a separate reserve stem-cell pool for every possible lesion. Conserved signalling modules can also be redeployed in new developmental contexts. These advantages must be weighed against loss of specialized function, energetic costs and the danger of inappropriate persistent growth. Comparative experiments should ask whether homologous lineages undergo similar transitions under comparable injuries; shared expression of a few regulators is insufficient to prove that an ancestral cell fate plasticity programme has been conserved. At the tissue level, cell fate plasticity supplies alternative states on which selection can act, but it does not itself establish heritable evolutionary change.
Clinically, controlled cell fate plasticity may improve epithelial repair, provide transplantable cells and make patient-derived disease models. The same capacity can undermine treatment: a tumour may switch to a less drug-sensitive lineage or regenerate a stem-like population after therapy. In carcinoma, epithelial-mesenchymal plasticity can contribute to invasion and treatment resistance, but neither a single EMT marker nor its absence establishes the mechanism of metastasis. In a lineage-traced mouse lung-cancer model, the tested EMT programme was dispensable for lung metastasis while contributing to chemoresistance; the conclusion is specific to that model and reporter coverage.[ref]
Epithelial-to-mesenchymal transition is not required for lung metastasis but contributes to chemoresistance by Kari R. Fischer and others. Lineage-tracing and chemotherapy experiments in mouse tumours
The useful clinical aim is therefore a defined, reversible transition that restores function, with evidence that it does not leave a persistently proliferative or malignant population. Past exam of the thermal and statistical physics course of the University of Cambridge 2016 Paper 1 4 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20For the ideal dilute Maxwell-Boltzmann gas implicit in a single-particle partition function, indistinguishability gives . With Stirling's approximation,Differentiate at fixed :This is a thermodynamic-limit ideal-gas result; arbitrary interacting classical gases do not have .
Equilibrium constraints and the Gibbs minimum. The open-system equilibrium contacts allow exchange of heat, volume and matter. For unconstrained contacts without external-field or interface corrections, equilibrium requires equal temperatures, pressures and each exchangeable species' chemical potentials across the contacts. These conditions follow by maximizing total entropy under conserved total energy, volume and species amounts.
The next minimization statement fixes the system's particle number. For a system in a reservoir at , with fixed and only pressure-volume work, the reservoir entropy change givesFor candidate states at the imposed , , the expression in parentheses is . Thus the Fixed-particle-number Gibbs minimum selects stable equilibrium at fixed , with stationary first variation and nonnegative allowed second variation. If particle exchange remains unconstrained, is not fixed and this minimization statement must be replaced by one incorporating the particle reservoir; it is not a justification for minimizing over arbitrary .
The simple-compressible-system first law givesFor a homogeneous extensive single-component phase, the Single-component Gibbs Euler relation follows from , yielding . For a mixture, the corresponding identities are and . Surface effects or other nonextensive contributions require additional terms.[ref]
Classical Thermodynamics by David Tong. Free energies, chemical potential and equilibrium with imposed reservoir variables
Reaction equilibrium. Let be an allowed reaction extent for the forward process, so and . At fixed ,For an interior equilibrium allowing both reaction directions, the coefficient vanishes:At fixed , minimizing gives the same condition. The reaction formula-unit conservation gives , not the total number of gas particles. This conservation law replaces fixed total particle number for the reacting mixture.
Using the stipulated single-particle functions,The number-based dissociation equilibrium ratio is thereforeThis number-based quantity has a factor of volume; the corresponding concentration ratio depends on temperature alone in the stated ideal model. A standard activity-based equilibrium constant would additionally specify reference states. No bond-energy factor is added to the functions given in the paper.
Define the dissociated fraction of original A formula units by . Then and , soThe dissociation fraction versus conserved density follows because the left side increases monotonically from zero to infinity on . At fixed , increasing decreases , hence decreases dissociation. Equivalently, at fixed compression raises and favours A. Association produces fewer independent translating particles; at high density the translational-entropy advantage of the two-particle side is smaller, so equilibrium shifts toward the one-particle side.
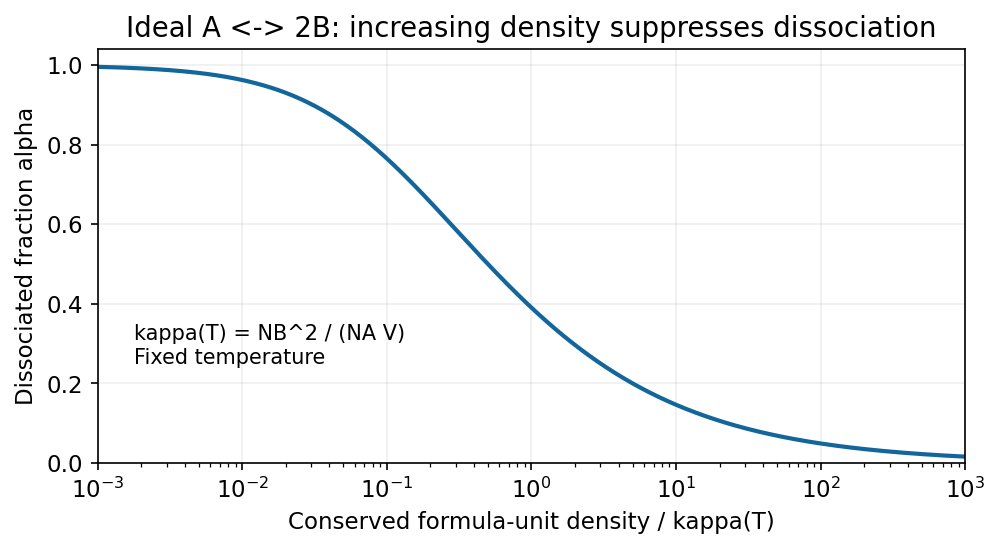
Past exam of the thermal and statistical physics course of the University of Cambridge 2016 Paper 1 3 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Measure energies from the single-particle ground state, and assume the three-dimensional ideal Bose gas in the large-particle-number limit. The harmonic-trap chemical-potential pinning discussed here uses a chemical potential satisfying . On cooling, it approaches zero; below the condensation temperature it remains at zero to leading thermodynamic order. Above that temperature it is negative. The detailed negative-chemical-potential branch shape is determined by the density of states; the figure uses the harmonic trap analysed below. The finite-size condensate chemical potential stays slightly below zero rather than being exactly pinned there.
A Bose-Einstein condensate has macroscopic occupation of a single quantum state. A dilute atomic gas needs low temperature and high phase-space density while remaining metastable against ordinary liquid or solid formation. Laser cooling followed by evaporative cooling of atoms in a weak trap can achieve the required regime. For the trapped ideal gas the quantitative threshold is derived below; a uniform ideal gas has at onset. An experimental signature is a narrow low-momentum component appearing within the broader thermal distribution after time-of-flight expansion, as observed in magnetically trapped rubidium-87.[ref]
Observation of Bose-Einstein Condensation in a Dilute Atomic Vapor by M. H. Anderson and others. 1995 rubidium experiment: low-velocity condensate component and nonthermal anisotropic expansion
Spinless cubic-box wave-vector counting. Impose periodic boundary conditions on a cube of side . The allowed vectors are with integer components. Each state occupies in wave-vector space. For a spinless particle, counting the spherical shell givesThere is no spin multiplicity. This is continuum shell counting; a finite box has discrete levels. Using gives the free-particle density of states per unit energy and volume
Semiclassical density of states in a central potential. At position , the available kinetic energy is . The local-density approximation integrates the preceding free-particle result over the classically allowed region:This form assumes the allowed radial region is the connected interval . A nonmonotonic potential would require integrating all allowed shells.
For the isotropic harmonic trap, . Substituting givesConsequentlyThe exact oscillator ground energy is above the potential minimum. The harmonic-trap energy-zero convention subtracts that constant, while the displayed density of states is the leading semiclassical continuum expression, neglecting the finite-level corrections produced by that shift. The discrete ground state must be counted separately.
Condensate population. Below the transition, use for the excited states. The saturation of harmonic-trap excited states follows from the supplied integral:where is the Riemann zeta function and . Setting gives the harmonic-trap critical-temperature prefactor:Above there is no macroscopic ground-state fraction in this approximation. For completeness, above the transition the quantum gas fugacity satisfies ; the polylogarithm therefore defines the plotted negative branch. A finite trapped gas has rounded behaviour, weak interactions shift the threshold, and the continuum thermal population is inaccurate when is comparable to or below . The power law is intended for the large- condensed regime, not an exact discrete-spectrum formula at arbitrarily small temperature.[ref]
Quantum Gases by David Tong. Section 3.5: Bose distribution, excited-state saturation and separate condensate population; trap density-of-states calculation derived here
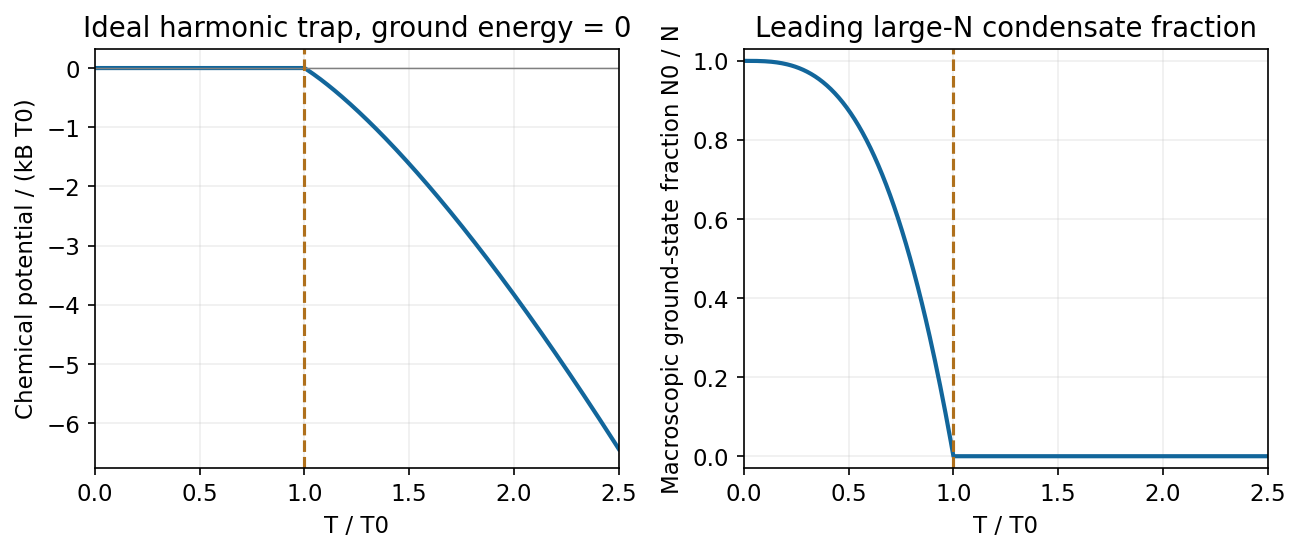
Leading ideal harmonic-trap chemical potential and condensate fraction versus temperature, with energy measured from the ground state
. Source. Details. Past exam of the thermal and statistical physics course of the University of Cambridge 2015 Paper 1 4 Solution by Codex 0 Created 2026-10-20 Updated 2026-10-20
Codex 0 Created 2026-10-20 Updated 2026-10-20Landau description. Introduce a macroscopic order parameter and expand an appropriate free energy analytically in that parameter, retaining terms permitted by the physical symmetries. Stable equilibrium minimizes this free energy globally; a local minimum with larger free energy is metastable. Coefficient changes with temperature can exchange the preferred minima. A continuous emergence from zero can produce a continuous transition, while competing separated minima can produce a first-order transition. Stability requires a positive highest retained even-power term. This local mean-field description neglects spatial fluctuations and nucleation dynamics unless gradient and dynamical terms are added; near a critical point those omissions can matter.
Local behavior at the origin. To determine constrained order-parameter boundary stability, note that and , the origin is a local minimum for and a local maximum for . At , the quadratic term vanishes, but for small positive . ThereforeThe equality case uses the stipulated domain . On an unrestricted real line, the nonzero cubic term would instead make it a stationary inflection point.
Global stability in both inline cases. For , complete the square in :The quartic coefficient guarantees a bounded global minimum. A negative value exists precisely when the minimum of this quadratic factor is negative. Hence case a, , has a nonzero globally stable phase with for every physical temperature. Case b, , has such a phase exactly forAt , the square's centre is at the boundary, but its negative constant still gives for small positive , so this endpoint is included.
At ,The two global minima have equal free energy, and . The coexistence barrier of a cubic-quartic Landau transition has its maximum at , with barrier height .
For locating the extrema away from coexistence,Retain only real positive roots; when both are positive, is a local maximum and a local minimum. For , only is positive. If , the pair first appears on cooling at ; if , a higher-free-energy nonzero minimum already exists at arbitrarily high temperature. These local-stability limits must not be mistaken for the global coexistence condition. The boundary also favors a nonzero minimum at every finite temperature, but has no finite .
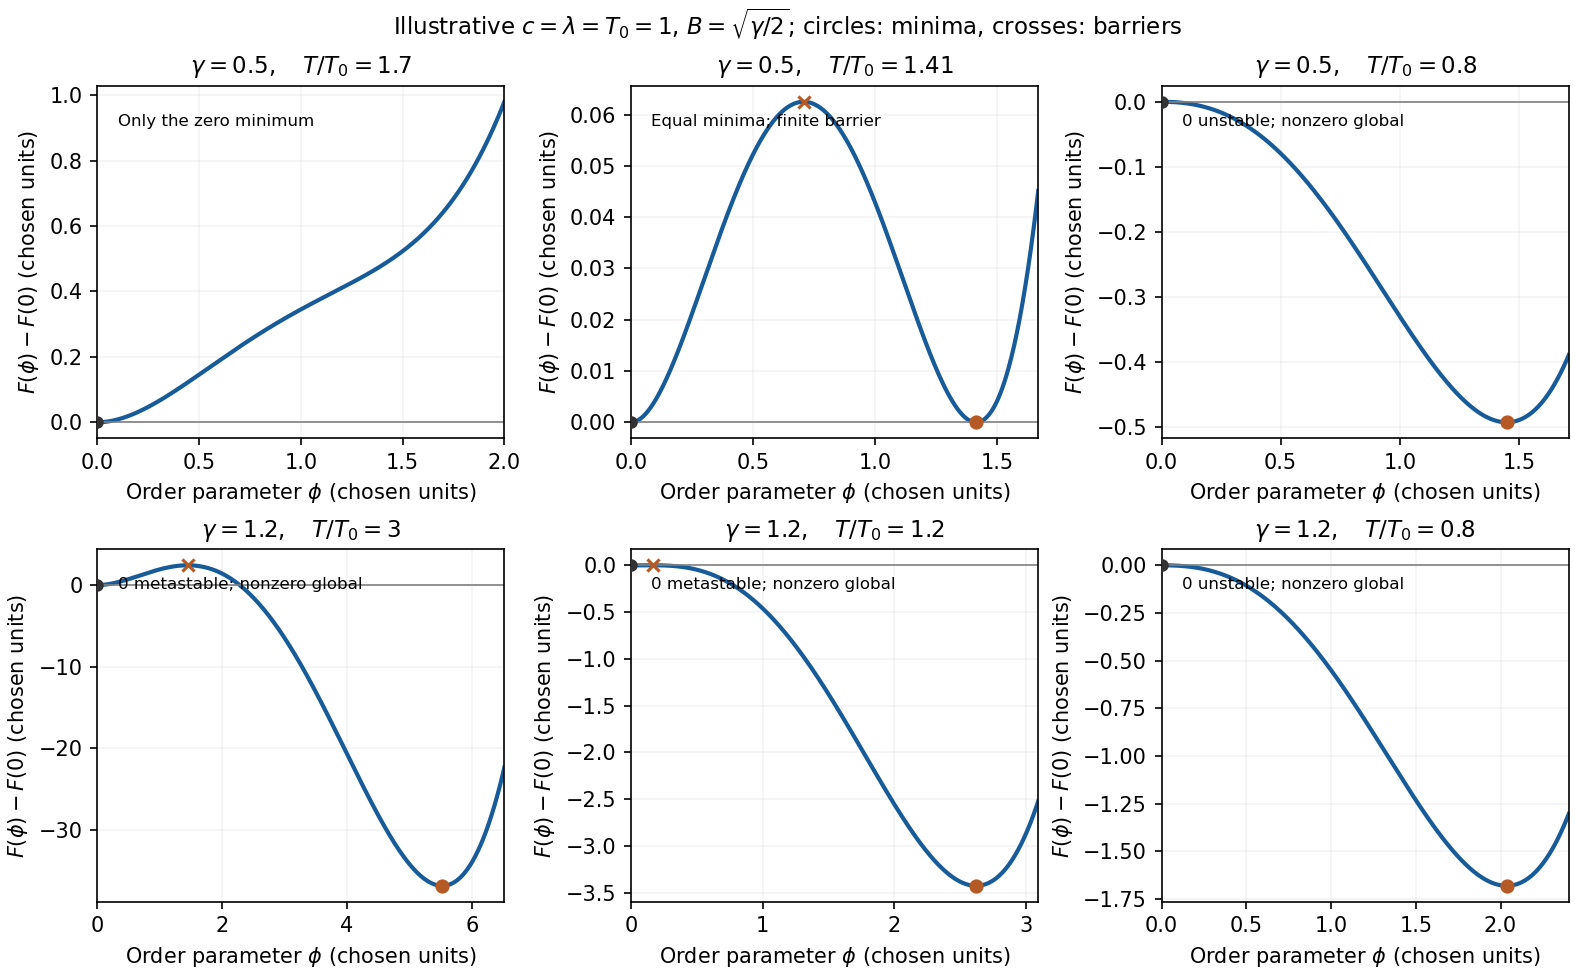


Cooling and transition temperature. For , equilibrium starts at the zero minimum at high temperature and switches to the nonzero minimum at . The jump is finite, , and there is a barrier between the coexisting states. This is a first-order transition. The latent heat of a temperature-dependent cubic-quartic Landau transition follows from differentiating the minimized free energy: the heat released on cooling isIf is an energy density rather than total energy, is likewise a density. An actual system can supercool below before nucleation, so is the equilibrium transition temperature.
For thermal symmetry nonrestoration in a cubic-quartic model, with , the equilibrium global minimum is nonzero already at arbitrarily high temperature. Following it does not force a transition. A system initially prepared in the metastable zero minimum can still leave it by nucleation while ; that minimum loses local stability at . This is the sense in which a change is possible rather than inevitable. There is no equilibrium coexistence temperature for in this model. A kinetic transition can depend on preparation and nucleation dynamics; is the limiting loss of local stability of the zero state, not a second coexistence temperature. Continuing to an imaginary value does not define a physical transition temperature.
Mass window in the specified electroweak phase transition model. For the mass window in a cubic electroweak transition model, put . The supplied ratios implyThe two strict conditions therefore requireSince is increasing for , the finite window isUsing the specified and givesAt u, , but . Thus 134 u lies outside the required window, failing the order-parameter-strength condition. This does not remove the polynomial model's finite first-order jump; it fails the additional requirement . The result is a bound within the specified simplified model, not a model-independent Higgs-mass bound.
Past exam of the thermal and statistical physics course of the University of Cambridge 2015 Paper 1 3 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Ensemble and applications. A grand canonical ensemble describes a system exchanging both energy and particles with a large reservoir. Its fixed control parameters are , while microstates with different have probabilitiesWeak coupling allows the system's energy levels to remain meaningful; equilibrium fixes the reservoir temperature and chemical potential. The grand potential is , with now the mean population. It generates entropy, pressure and mean particle number by differentiation. This ensemble is convenient for gases in contact with particle reservoirs, independently occupied quantum levels and surface adsorption; its particle-number fluctuations are part of the description, not an error in counting.
Classical single-level limit. For the single-level grand partition function in the dilute limit, put . Empty and singly occupied levels contribute and . In the dilute classical limit , higher occupancies contribute only at order or beyond:This truncation does not impose the Pauli principle on a classical gas. A fermion state has exactly , a boson state has , and Maxwell-Boltzmann occupancy weights give ; they all agree to this order. In particular, , with the classical Maxwell-Boltzmann result exactly .
grand potential and chemical potential. With , summing the single-level logarithms and using the stated density of states givesSubstitute , for whichCombining this with the density-of-states prefactor gives . ThusDifferentiating at fixed ,Similarly , so . This is the grand-canonical chemical potential of a classical ideal gas. The condition states the classical regime. The supplied density of states counts one internal state; extra internal degeneracies would have to be included consistently rather than inserted at only one stage.
One adsorption site. Take the free-vapour energy reference as zero and the binding energy as . A site is either empty or singly occupied; the latter has vibrational partition function . Its adsorption-site grand partition function and mean occupation areThe chemical potential of an adsorbed species on equivalent sites follows by inverting the occupation ratioThe factor is the vacant-site probability. The binding reference and the energies included in must be chosen consistently, so that vibrational zero-point energy is not counted twice.
Isotherm. The vibrational factor in a Langmuir equilibrium constant is fixed by adsorption equilibrium, . Neglecting vapour internal degrees of freedom and writing its number density as gives . ThereforeThis is the Langmuir isotherm: initially linear, increasing monotonically and concave down, approaching unit coverage. Half coverage occurs at . The coefficient has inverse-pressure units. It assumes equivalent independent sites, at most one molecule per site and no lateral interaction or multilayer adsorption. The molecular mass appropriate to the vapour determines .
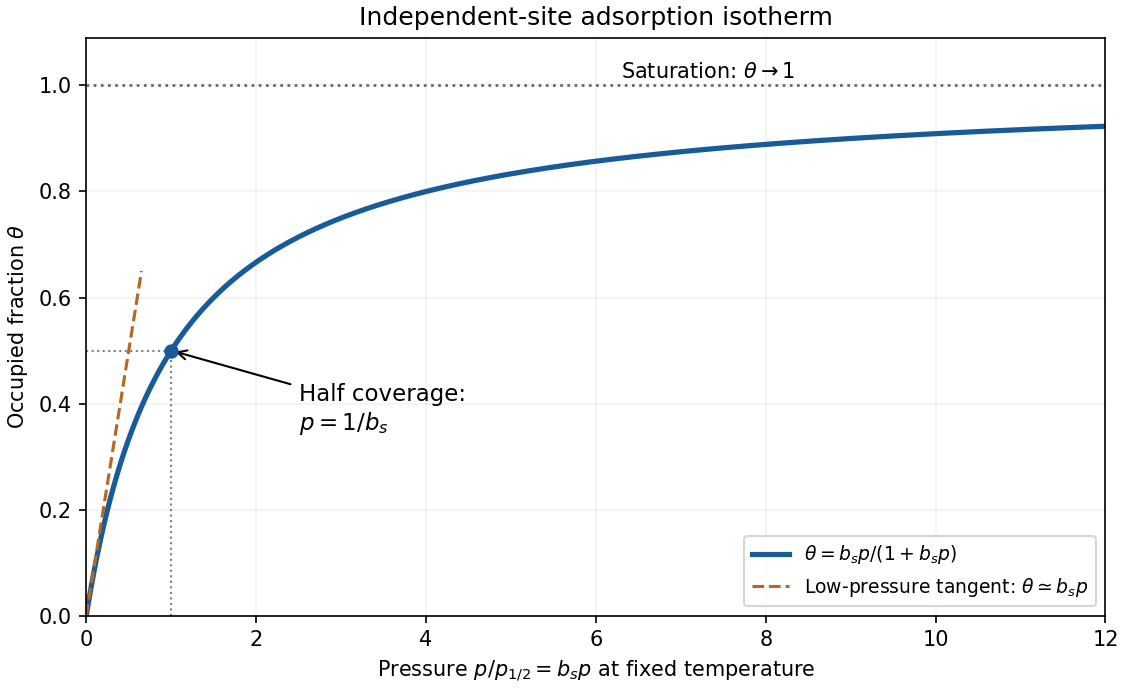
Original dimensionless Langmuir coverage curve with half-coverage and limiting behavior
. Details. 
A real uptake measurement must separate adsorbed molecules from free gas in the apparatus. Langmuir's original mica experiment compared a mica-containing bulb with a similar blank and inferred uptake from calibrated gas volumes and pressures. His stated blank contribution and bath-temperature drift limited the inferred adsorption; a saturating curve alone does not establish ideal equivalent sites.[ref]
The Adsorption of Gases on Plane Surfaces of Glass, Mica and Platinum by Irving Langmuir. pp. 1376–1378: mica apparatus and blank; p. 1385: limitations
Past exam of the thermal and statistical physics course of the University of Cambridge 2014 Paper 1 4 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Use for molar volume to distinguish it from the fluctuating parcel volume below. The equation is . The parameter models excluded volume, while models the reduction in pressure from attractive interactions.
Below the critical temperature, a raw isotherm has a loop. The positive-slope segment is mechanically unstable and surrounding metastable portions do not give the stable equilibrium mixture. Replace the loop by a constant coexistence pressure satisfying the Maxwell equal-area condition,The endpoints are liquid and vapour molar volumes; intermediate mean volumes correspond to phase mixtures with changing proportions. Above the critical temperature, liquid-like and gas-like states connect continuously without a coexistence plateau.
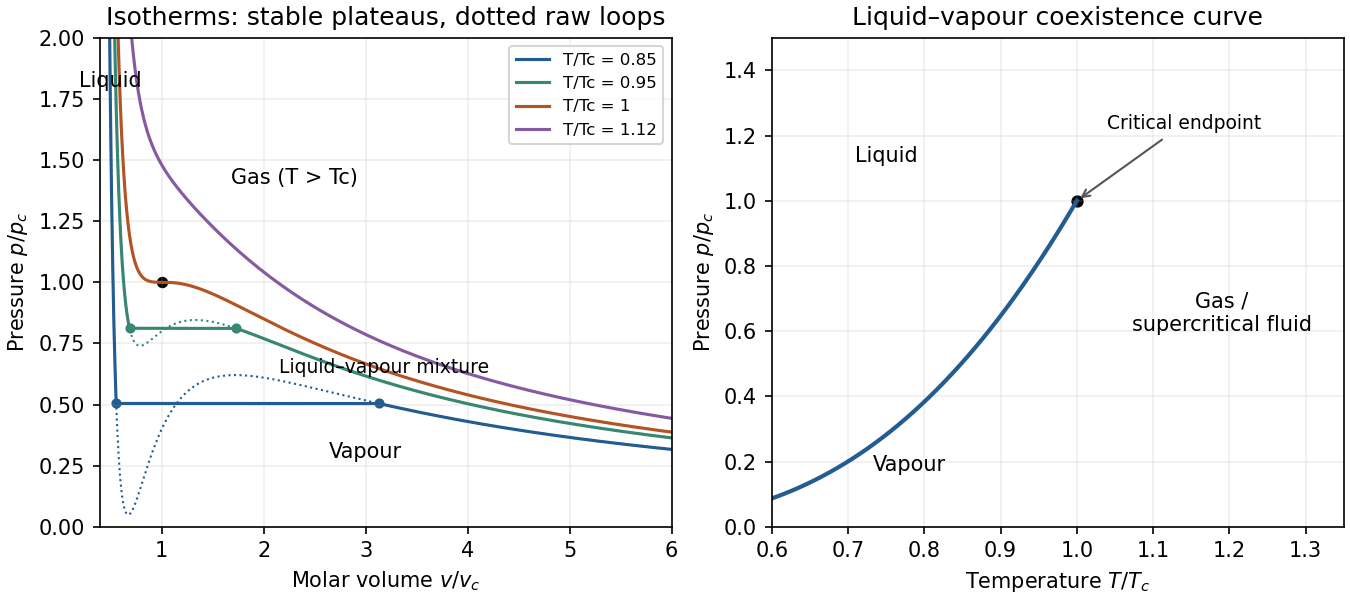
Original reduced van der Waals isotherms with computed Maxwell coexistence plateaus and the pressure–temperature coexistence curve ending at the critical point
. Details. 
In the pressure-temperature diagram, the liquid-vapour coexistence line ends at the critical point. Below it, the low-pressure side is vapour and the high-pressure side liquid. “Gas” conventionally denotes the region above the critical temperature, where compression alone cannot cross a liquid-vapour transition. The model has no solid phase.
The critical isotherm has an inflection: . Thuswhich giveFor fluctuations about a stable equilibrium value , the system plus reservoir has probability proportional to . Expanding availability,gives a Gaussian distribution and, to this order, withThis requires positive curvature and sufficiently small fluctuations; it is not exact when higher-order terms matter.
The whole cylinder's volume is fixed. For the volume fluctuations of a small fluid parcel, interpret the small quantity as a material parcel containing moles, whose volume can fluctuate against the much larger remainder. Its mean volume at the critical density is . At fixed temperature its availability is , soOn the critical isochore, approached from ,ConsequentlyEquivalently, , with . The mean-field variance diverges as , so its critical exponent is ; the root-mean-square fluctuation has exponent . A fixed spatial observation box instead has number fluctuations, not fluctuating geometric volume. Finite size and non-Gaussian terms cut off the literal divergence; the approximation fails exactly at the critical point.
There are unlisted articles, also show them or only show them.