Source bundle pages 55–61. The cover identifies Trinity Term 2022, C7, despite the attachment's 2021 filename. Solutions use the conventions and figures on the original pages.
The bacterial RNA polymerase core associates with a sigma factor to form a holoenzyme. The sigma factor recognizes promoter features and helps position the DNA and stabilize its opening. Initial binding gives a closed promoter complex; local DNA unwinding creates an open promoter complex with the template accessible. Initial RNA synthesis can produce short abortive products while the RNA polymerase remains attached to the promoter, taking in downstream DNA by scrunching. Growth of the RNA eventually permits promoter escape and productive elongation. The sigma factor changes its interactions during this transition; immediate complete dissociation is not obligatory.
In magnetic tweezers, torsionally constrained DNA joins a surface to a magnetic bead. A field gradient applies upward force, rotation of the magnets controls the imposed DNA supercoiling, and optical tracking measures bead height. At suitable modest force, DNA supercoiling forms writhed loops, shortening the tether. Opening roughly one helical turn at fixed linking number makes the remaining DNA more positively twisted: . Thus opening lengthens a negatively supercoiled tether by removing some negative writhe, but shortens a positively supercoiled tether by adding positive writhe. This opposite sign distinguishes unwinding from ordinary compaction, which shortens both tethers. Height-versus-turn calibration converts the two extension changes into an unwinding angle and a compaction contribution. Repeated height transitions give opening and closing dwell times.[ref]
Promoter unwinding and promoter clearance by RNA polymerase: Detection by single-molecule DNA nanomanipulation by Andrey Revyakin and others. Figures 1–3: torsionally constrained tether, opposite-sign extension responses, and approximately one-turn unwinding
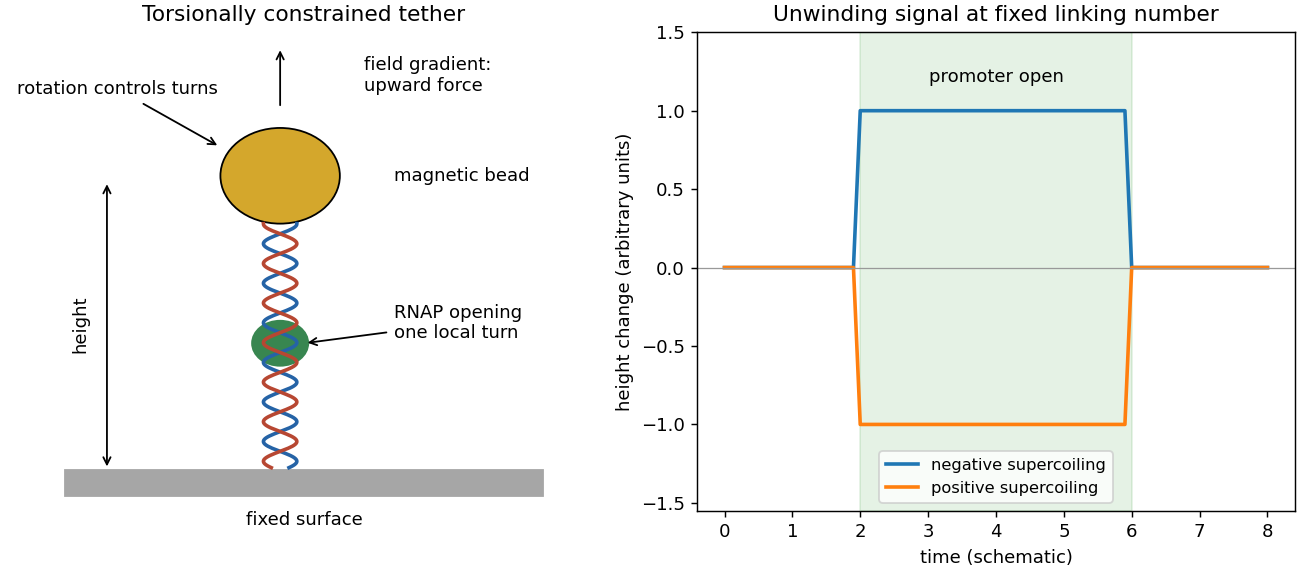
The sketch is a schematic prediction, not a copy of an experimental trace. Opening must be distinguished from promoter escape: an unwound DNA region can remain associated with an elongating RNA polymerase.
Treat the target as an absorbing sphere of effective capture radius , surrounded by a uniform dilute reservoir of RNA polymerase with number density . The steady diffusion equation, spherical symmetry, and boundary conditions giveBy Fick's laws, the inward capture rate per target is . Multiplying by the target number density and comparing with the bimolecular rate law therefore yields the Smoluchowski association rateIts units here are , since the concentrations count particles rather than moles. The absorbing boundary assumes every encounter is productive; orientation constraints would reduce the effective association rate constant.
The Stokes–Einstein relation, for RNA polymerase radius at an illustrative temperature , givesNeither cell volume nor the effective is specified, so a unique numerical time is unavailable. A representative Escherichia coli volume is . The -base pair target has a DNA contour extent of about ; using this as an order-of-magnitude capture radius gives . For independent searchers, the target's approximately constant encounter hazard is , henceUsing half the target's contour extent for instead gives about ; the spherical capture model is not exact target geometry. One searcher's mean would be about under the first convention, whereas the first arrival among is much faster.
If only a fraction of each searcher's time is available for three-dimensional diffusion, and nonspecific DNA binding neither scans nor delivers the target, the effective searching population is . Thus , about under the stated estimate. This assumes stationarity, well-mixed searchers and no additional target-access route; nonspecific binding alone is sequestration, not facilitated diffusion.
Write and . The search time is : it decreases from infinity at small positive , reaches one minimum, and increases without bound at large within this idealized model.
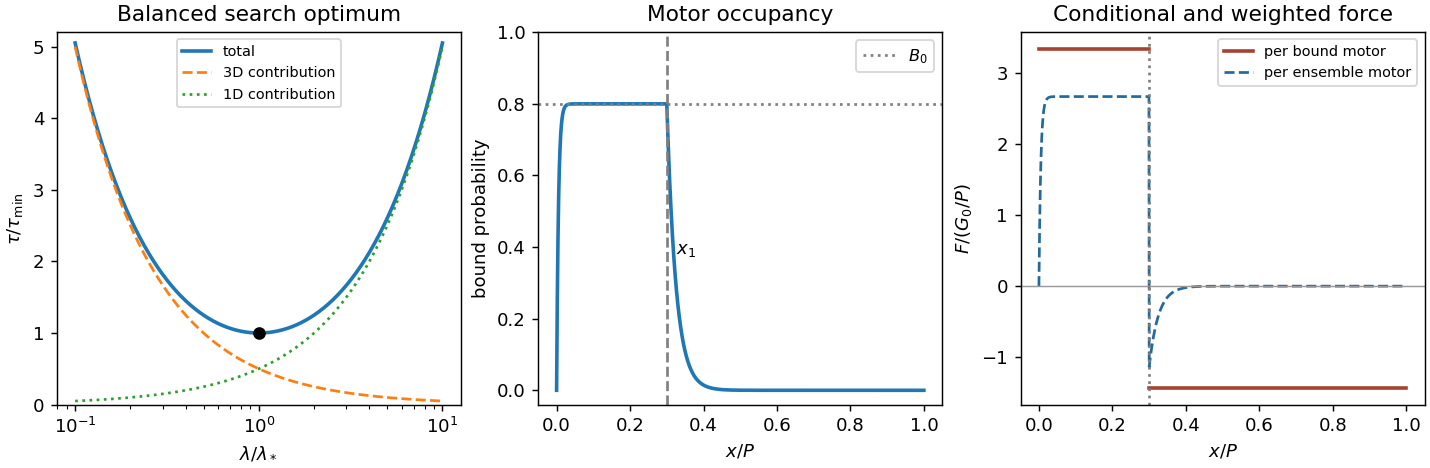
During a facilitated diffusion search, roughly separate DNA landing-and-sliding episodes sample a chromosome. A three-dimensional encounter with any chromosomal landing region has characteristic time , so the total bulk-search contribution is . Each one-dimensional diffusion excursion lasts order ; multiplying by gives . Longer sliding therefore reduces the number of bulk relocations but increases time spent repeatedly exploring local DNA. Numerical constants and overlap corrections are already omitted in the given model.
Differentiating and using the positive second derivative givesAt the two time contributions are equal. The optimum is meaningful only if lies between the microscopic capture scale and the available chromosomal contour length.
A decrease in DNA concentration means a decrease in , but its effect on the time is not determined by that ratio alone. At fixed chromosome length , dilution by increasing increases at fixed and increases as ; bulk relocation becomes slower. If instead decreases at fixed , while the target is retained, the stated model predicts a smaller sliding contribution and a smaller optimized time, proportional to . In both cases . This distinction prevents attributing a unique time trend to concentration without specifying how it changes.
Let be the donor's total decay rate without acceptors, including radiative and nonradiative decay, and let be its transfer rate to one acceptor. In weak excitation, independent equivalent acceptors supply additive transfer rates, so FRET efficiency isEliminating givesThis assumes the same Förster distance, equivalent donor–acceptor distances and unchanged donor decay, with no acceptor saturation or other transfer pathways affecting donor de-excitation.
For Förster resonance energy transfer, , henceHere the single-pair FRET efficiency would be , which indeed produces .
Use the logic approximation for gene regulation: production is either or zero, and every species has linear removal rate . Put and assume zero basal expression, inactive X before time zero, and all required thresholds strictly between and . The input is for and zero otherwise. The common ordinary differential equation is , with Boolean production gate . Both networks therefore havewhere the latter uses the stipulated attained steady state. Define the threshold-crossing delayBecause , . In both networks, stays zero until and then follows until the OFF response. Write for the activation threshold of on Z in diagram (a), and for the level of that blocks Y's repression in diagram (b); these thresholds were not supplied numerically.
Diagram (a). All three inputs X, Y and must permit Z production. Since Y has already crossed its Z threshold before starts, the final permission arrives atThus until and subsequently. Solving givesFor the frequently adopted but extra convention that both required thresholds are , this is . At the OFF step, X's direct AND input disappears, so immediately. Y also decays immediately. remains at while Y remains above ; it starts decaying at . This is a coherent feed-forward loop persistence response: activation is delayed, while removal of the direct required input switches production off promptly.
Diagram (b). The production gate is . Z initially rises, Y switches Z production off at , and restores production at . The continuous solution during the ON phase isThe derivative changes from positive to negative at , and from negative to positive at . Consequently the first temporary minimum following the initial pulse occurs atIts value is . At the OFF step Z again decays immediately because X is required for production, with Y and behaving as above. If a required threshold is unattainable, these late switching events do not occur; equal production and removal rates alone do not fix threshold values.
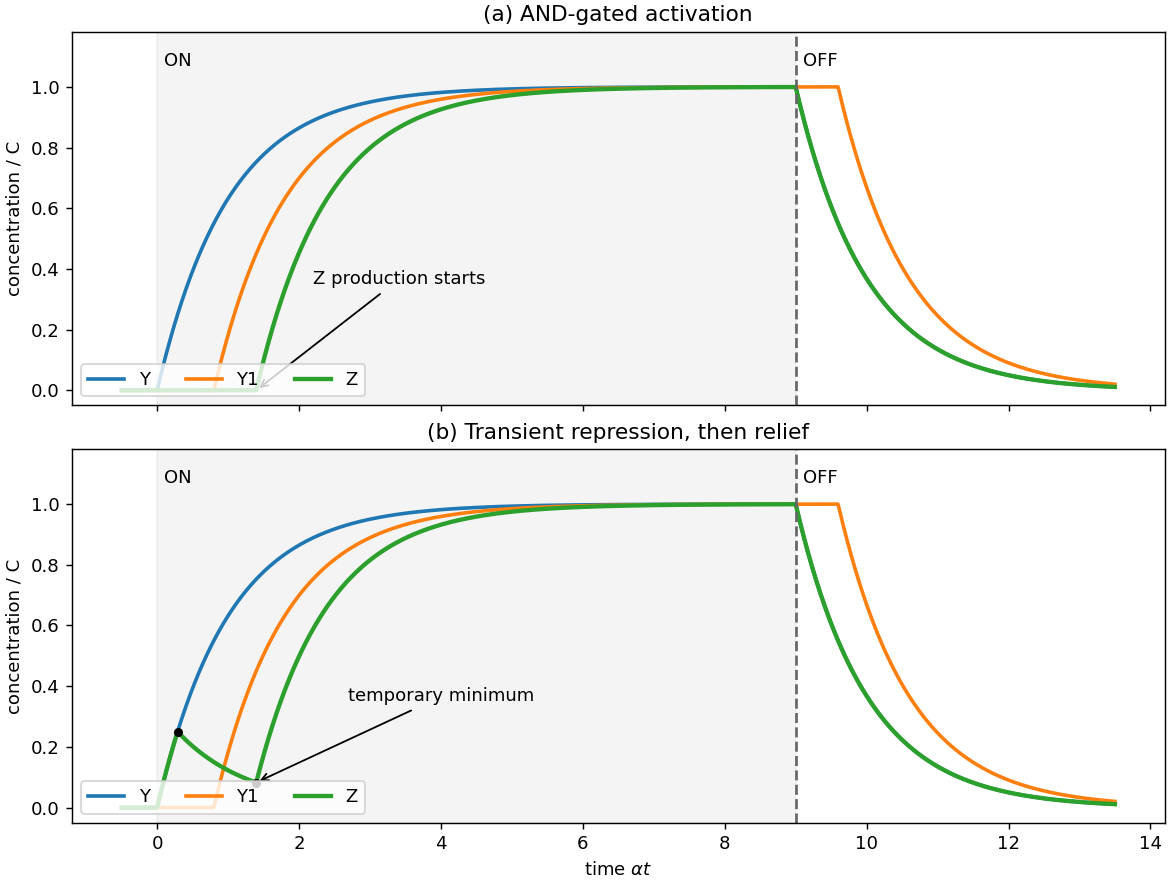


The plotted thresholds are explicitly illustrative, with , and .
The protein production rate is proportional to the current messenger RNA concentration, not an independently constant : . Setting the two coupled rate equations to zero givesWith first-order removal, a messenger RNA molecule has mean lifetime . At biological translation rate per molecule, it produces an expected proteins before its removal. Thus the translational burst size is a dimensionless mean number of offspring proteins per messenger RNA, not a concentration and not a fixed number produced in every event. When production and removal are independent Poisson events, mixing a Poisson number of biological translation events over an exponentially distributed lifetime makes the burst count geometrically distributed on the nonnegative integers. Its mean is and its variance is .
Convert number density into molecule count: . For the explicitly assumed representative cell volume , the two densities correspond to and . The concentrations alone do not fix fluctuation sizes without a volume.
For activation from zero messenger RNA and protein, solving the two mean rate equations givesThus all three normalized mean curves are almost identical. Sample paths differ. For Poisson transcription with biological translation bursts, the stationary Fano factor and squared coefficient of variation areOne way to obtain the fast-messenger RNA limit is to use burst arrivals at rate , a geometrically distributed burst with and , and independent unit protein degradation at rate . The first stationary moment gives ; the second gives .
At , typical relative fluctuations are and many small bursts make the trajectory smooth. At , they are ; individual bursts have mean normalized height , with only about bursts per protein lifetime. At , the relative fluctuations are again , but the typical burst height is and about bursts occur per lifetime. The latter two examples can look similarly noisy after normalization even though their mean molecule counts differ by two orders of magnitude. Burst arrival times and sizes fluctuate: a high-burst trace is not a periodic sawtooth.
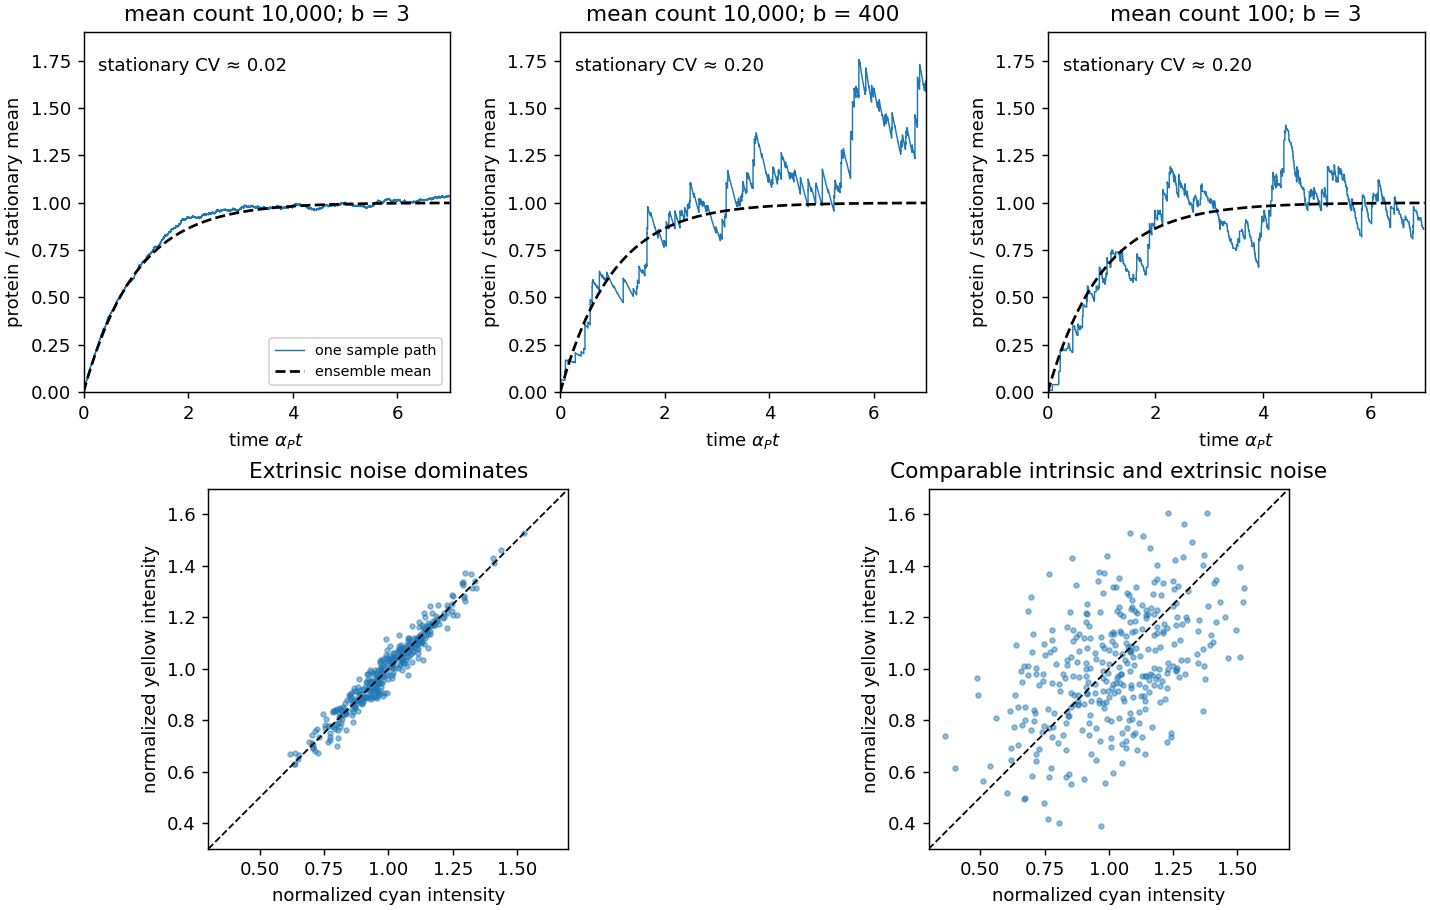
Stochastic gene expression trajectories and dual-reporter intrinsic gene-expression noise and extrinsic gene-expression noise
. Details. 
The upper panels are independently simulated burst-arrival and unit-removal processes, shown alongside the common mean. The lower panels illustrate d; their point clouds are schematic, not experimental data.
Normalize each reporter by its mean intensity, after correcting background and unequal brightness, so equal expression lies on . Write , , where the common fluctuation is extrinsic gene-expression noise and the independent reporter-specific fluctuations are intrinsic gene-expression noise. The extrinsic gene-expression noise includes shared variation in cell size, expression machinery and growth state; intrinsic gene-expression noise includes independent molecular production and removal events at each reporter.
If intrinsic gene-expression noise is much smaller, points form a narrow elongated cloud along : a cell that is bright in cyan is usually bright in yellow. If the two contributions have comparable magnitude, the cloud is still positively correlated but has substantial width perpendicular to , because the two reporters can differ within the same cell. With variance in and equal variance in each independent intrinsic term,Equal intrinsic and extrinsic variances therefore give correlation coefficient , rather than an uncorrelated circular cloud. For mean-normalized reporters, and . Measurement noise must be separately estimated before assigning perpendicular scatter to expression itself. These are the geometric diagnostics of the original dual-reporter experiment.[ref]
Stochastic Gene Expression in a Single Cell by Michael B. Elowitz and others. Figure 1 and definition of intrinsic and extrinsic noise: within-cell reporter differences versus correlated cell-to-cell variation
The lower panels of c show these two cases. Repeated observations of one cell can move both along and across the diagonal; a static population cloud alone does not determine the time scales of the fluctuations.
In the continuum cylindrical-pore estimate, the electrical resistance is , with radius , length and electrical resistivity . ThereforeUnrestricted approach from the reservoirs removes access barriers, but still permits a continuum spreading or access resistance of a circular pore. Including on each side givesThus the usual estimate neglecting the access contribution is about , or about with spreading resistance. A -ångström diameter is at the molecular scale, smaller than hydrated ions; bulk electrical resistivity cannot quantitatively describe dehydration, selectivity or discrete-ion transport. These values are the requested continuum estimates, not evidence that such a pore freely passes hydrated potassium ions.
The rising sigmoid shows activation by depolarization: is almost zero at very negative membrane potential, rises steeply around , and approaches about at positive membrane potential. The graph describes the fraction of time a single ion channel is open, not a continuously variable opening amplitude. A convenient phenomenological fit isHere refers to half the maximum, about , not absolute . The effective gating charge describes the steepness; a sigmoid alone does not identify the microscopic gating sequence or explain why the observed maximum is below one.
A voltage-gated potassium channel has four pore-forming subunits. Each canonical subunit contains an S1–S4 voltage-sensing domain and S5–S6 pore elements. Positive charges in S4 respond to the electric field; their displacement during depolarization changes the energetic preference of sensor conformations. Coupling through the sensor–pore interface favors opening of the intracellular pore gate. The potassium selectivity filter is structurally distinct from this voltage sensor.
Several independent observations support this account. Voltage clamp detects transient gating electric currents before pore conduction, even when ionic conduction is blocked: charge movement precedes opening. Charge-neutralization studies change total gating charge and voltage dependence, with contributions from charged S4 residues and an S2 residue. Accessibility and voltage-sensitive optical measurements support conformational motion rather than permeating potassium itself acting as the sensor. Structural measurements locate the charged sensor beside the pore. These observations constrain a coupled moving-sensor mechanism, while the exact displacement cannot be deduced from this curve alone.[ref]
Voltage-sensing residues in the S2 and S4 segments of the Shaker K+ channel by S. A. Seoh and others. Abstract: gating-charge measurements identify contributions from S2 and S4 charged residues
[ref]Crystal structure of a mammalian voltage-dependent Shaker family K+ channel by Stephen B. Long and others. Structure of Kv1.2: separate voltage-sensor and pore domains and their coupling
An open ion channel carries the electric currentThe macroscopic mean is , so is the mean number open, not the total number present. Reading from the original graph givesThe graph reading is approximate, so a precision of hundreds is appropriate. Only a few hundred active ion channels generate a nanoampere-scale cellular electric current; molecular discreteness and stochastic gating therefore matter. For independent identical ion channels, the open-count standard deviation is , corresponding to a coefficient of variation in electric current of about . This is an instantaneous ideal independent-gating estimate, before temporal filtering and other noise sources, and requires the single-channel recording to apply to the cellular recording conditions.
In ball-and-chain inactivation, also called N-type inactivation, a flexible intracellular N-terminal region carries an inactivation particle. Once a voltage-gated potassium channel opens, this tethered particle can enter and occlude the inner pore, stopping electric current even while the activation machinery favors an open configuration. Recovery requires the particle to leave, after which the activation gate can return to its resting conformation. This supplies an additional unavailable state, not merely reversal of activation.
The decisive evidence separates necessity from sufficiency. Removing the relevant N-terminal region greatly reduces fast ion-channel inactivation while preserving activation. Applying a peptide corresponding to the missing N-terminal region on the cytoplasmic side restores blocking with similar properties. Changes in the blocking region alter blocking kinetics, and altering the tether affects the rate at which the particle reaches the pore. Open-pore access and competition with intracellular pore blockers support occlusion of the inner cavity. A tether makes the particle's local effective concentration high, explaining rapid intramolecular block.[ref]
Biophysical and molecular mechanisms of Shaker potassium channel inactivation by Toshinori Hoshi and others. N-terminal perturbations separate rapid inactivation from activation
[ref]Restoration of inactivation in mutants of Shaker potassium channels by a peptide derived from ShB by William N. Zagotta and others. Cytoplasmic N-terminal peptide restores inactivation in deletion mutants
This mechanism is distinct from slower filter-associated C-type inactivation. An N-terminal particle is a mechanism for certain potassium ion channels, not a universal explanation of all ion-channel inactivation.
In a classical action potential, delayed activation of voltage-gated potassium channels supplies outward electric current that drives repolarization. In the Hodgkin-Huxley model, for example, and . Increasing the opening rate at depolarized membrane potential, other properties fixed, recruits outward electric current earlier: the action potential generally becomes narrower and may have a smaller peak. Slower opening delays repolarization and broadens the action potential.
Slower closing after repolarization retains excess potassium electrical conductance, lengthening the after-hyperpolarization and often the interval of reduced excitability. Faster closing shortens this tail and permits earlier recovery. If activation or the available electrical conductance is insufficient, normal repolarization may fail; changing rates can also change the steady open fraction. Duration is therefore determined by the whole balance of inward and outward electric currents, not by a closing rate in isolation.
Detailed balance means that at thermodynamic equilibrium each elementary transition and its reverse carry equal probability flux. For normalized state probabilities and ,With the printed convention , the sign is thereforeThe values are free energies per system, including internal degeneracies; for molar Gibbs free energies, replace by . If B has lower free energy, its forward-to-reverse rate ratio exceeds one, as it should.
For constant rates, conservation gives , so the master equation is . Its steady state is , and separation of the decaying deviation yieldsfor the specified initial state A. The relaxation time constant is .
Take and the displayed potential energy to be the position-dependent mechanical free energy of a bound motor. On the descending ramp , and on the ascending ramp . Thus the force conditional on being bound isIt is periodic, piecewise constant and undefined at idealized sharp corners; the corners have zero measure in averages. An unbound motor has zero force.
A cohort transported through position obeys . Its bound probability therefore satisfiesDefine , , , and . The exact periodic steady state includes a small carry-over :These expressions follow by solving each first-order ordinary differential equation, requiring continuity at , and imposing periodicity.
The stipulated implies , so the incoming bound fraction is exponentially small. Dropping it gives the simpler intended formsThe occupancy rises towards on the binding interval, then decays over length outside it. The mean force per member of the full ensemble at a given position is , distinct from the force per bound motor. The right panels of c show both the occupancy and the conditional force.
For a uniform distribution of phases along one period, average the ensemble force :Using the negligible-carry-over form in b givesConsequentlywhere . This is the printed expression to the accuracy justified by the velocity condition.
It is not an exact identity for the periodic problem at arbitrary . Keeping instead givesFor a concrete counterexample outside the small-velocity approximation, choose and . Then the exact periodic value is about , whereas the printed reset expression is about . The discrepancy is due to nonzero incoming occupancy, not an integration sign change.
As , both and diverge, and both formulas giveThe bound population occupies the downhill binding region, while occupancy on the uphill region is confined to a vanishing boundary layer. A nonzero limiting stall force is compatible with zero mechanical power . The spatially restricted binding and uniform unbinding do not obey local detailed balance for this sawtooth free energy: a passive equilibrium model would require to reflect the local energy difference and not vanish on an interval of finite energy. This is a driven or prescribed-kinetics motor model; the equilibrium relation in a cannot be imposed on it without an energy supply and additional states.
Write the end-to-end random vector as , with independent isotropically distributed unit vectors. At zero applied force, , , and for independence gives . ThereforeHere “size” is the root mean square end-to-end distance of a polymer chain. It is not the magnitude of the mean random vector, which is zero, nor the mean distance . In the long-chain Gaussian limit of the end-to-end distribution of a freely jointed chain, , illustrating why these definitions cannot be interchanged.
Each Cartesian component of one link has zero mean and variance , with zero cross-component covariance. By the multivariate central limit theorem, for large on the coil scale the vector probability density isIt is normalized with respect to ; the radial probability density is . The Gaussian limit of the end-to-end distribution of a freely jointed chain is an approximation, not the exact finite- law near .
At prescribed vector separation the configurational entropy is . The ideal chain has no extension-dependent internal energy, so its Helmholtz free energy isThe externally required force is , while the chain's restoring force has the opposite sign. ThusThe last equation also follows by multiplying by the Boltzmann factor and completing the square. This entropic spring resists extension because fewer link configurations realize a stretched chain. At the same small applied force, increasing temperature reduces extension; at the same extension it increases the required force. Do not differentiate to obtain the fixed-vector Hooke law, since that radial measure includes an additional geometric multiplicity. The low-force condition is , equivalently .
In atomic force microscopy, one end of the polyacrylic acid chain is attached to the substrate and the other to a compliant cantilever tip. Controlled separation displaces the cantilever; calibrated cantilever stiffness converts its deflection into force. The molecular extension is the tip–surface separation after correcting for cantilever deflection and instrumental offsets. A quasi-static interpretation requires relaxation to be fast compared with the pulling motion.
At low force a coiled polymer has many available configurations and extends mainly by changing segment orientations. This is the entropic spring regime. As the available contour is aligned, the loss of configurational entropy becomes steep. For an inextensible three-dimensional freely jointed chain,where is the Langevin function. The limiting extension is the polymer contour length ; the ideal model approaches it only as . Real polymer backbone stretching permits extension beyond the fitted rigid-link contour, explaining why the experimental curve lies on the more extensible side at high force.
The original trace has a sharp force drop after its peak. Finite contour length explains the steep preceding rise, but does not itself cause that drop: release of an attachment, desorption or mechanical failure ends tensile loading. The graph alone does not distinguish these possibilities. If the intact chain is released from tension, thermal motion restores a coil with characteristic end-to-end distance of a polymer chain of order , because this macrostate has many more configurations. Recoil is reversible for an intact equilibrating chain; irreversible chain scission or attachment loss can prevent repetition of the same pulling curve.
Identifying the fitted limiting extension with the polymer contour length givesThese are statistical links of the freely jointed chain, not necessarily chemical polymer repeat units. A measured maximum just before detachment need not equal the true contour length exactly, so the identification is itself an estimate.
The stated temperature request mixes two distinct quantities. At unchanged and , the true freely jointed chain maximum is geometric:In contrast, the low-force relation predicts a ratio at the same small force, not a new maximum:Formally multiplying by this ratio gives about , but is outside the small-extension domain, so that is not a justified maximum-extension prediction. A concrete internally consistent counterexample uses the same chain at : the low-force extensions are about and , while both contour lengths remain . Any temperature dependence of the segment length, solvent interactions, attachment strength or rupture force needs information absent from the model.
The rigid-link freely jointed chain stores extension entirely in orientation. It predicts and a divergent force as that limit is approached. Real chemical bonds and bond angles can deform, adding energetic compliance. This permits the measured chain to stretch farther at the same large force and removes the rigid-link vertical asymptote over the experimentally accessible range. Other limitations include segment correlations, solvent effects and eventual failure; a fit alone does not isolate their contributions.
Introduce one axial stretch modulus with units of force. A useful phenomenological extensible freely jointed chain law adds a linear strain contribution:Equivalently, if each aligned segment is a spring of stiffness in force per length, and the additional extension is . At high force, ; the extra term supplies finite axial compliance. At small force, the compliances add: .
This additive law is a simple requested one-term modification, rather than an exact angular average for harmonic links. Another common approximation is , which couples stretching to orientation. Neither should be extrapolated through bond rupture or claimed to predict a universal finite maximum for an extensible chain. A positive fitted could improve the high-force extension while leaving the entropic part largely intact.
Position from many photons. An isolated fluorophore produces a diffraction-broadened point spread function, but its unknown center can be inferred much more precisely than the width of that function. Fit a calibrated two-dimensional Gaussian function plus background to the detected photon positions or pixel intensities. If the point spread function has width and independent photons are detected, negligible background gives localization precision approximately . Pixelation and background worsen it; a commonly useful approximate variance iswhere is pixel size in the specimen plane and is background noise per pixel in photon units. Bright, isolated emitters can therefore have nanometre localization precision despite a spot hundreds of nanometres wide. Stage drift, finite exposure motion, incorrect fitting, label displacement and photobleaching can dominate the photon limit.[ref]
Precise nanometer localization analysis for individual fluorescent probes by Russell E. Thompson and others. Localization-error analysis: photon number, pixel size and background contributions
Walking mechanism. Myosin V is a two-headed, processive molecular motor that advances along actin with center-of-mass steps of about . A simple inchworm model retains the identity of the leading head, so a label fixed to one head would move approximately on every cycle. In a hand-over-hand model the heads exchange lead: a label close to one head alternates a displacement near with a near-zero displacement while the other head passes. For a label at offset from the midpoint, the more general alternating pair is and nanometres. The pair sums to ; individual steps need not always equal .
Single-label imaging records a moving spot on a camera while the motor travels along surface-associated actin. Fitting the spot in successive frames resolves plateaus and jumps much smaller than the diffraction width. The observed alternating displacements distinguish a passing-head mechanism from uniform inchworm steps. This experiment combines a specific geometric prediction with single-molecule fluorescence microscopy; the center-of-mass stride alone would not make that distinction.[ref]
Myosin V Walks Hand-Over-Hand: Single Fluorophore Imaging with 1.5-nm Localization by Ahmet Yildiz and others. Science 300, pp. 2061–2065: single-label tracking, 1.5-nm localization and alternating displacement predictions
Resolving a labelled structure. Accurate localization of one emitter does not automatically resolve two simultaneously overlapping emitters. Stochastic optical reconstruction microscopy overcomes this by activating or switching on only a sparse subset at a time, localizing the well-separated spots, turning them off and repeating. The accumulated coordinates reconstruct a densely labelled structure at scales below the diffraction limit. The original demonstration used repeated photoswitching and localization of individual dyes to reconstruct subdiffraction features.[ref]
Sub-diffraction-limit imaging by stochastic optical reconstruction microscopy (STORM) by Michael J. Rust and others. Nature Methods 3, pp. 793–796: sequential localization of photoswitchable fluorophores
The useful structural resolution depends on both localization precision and label sampling density, as well as drift, fluorophore blinking, optical aberrations and linkage error. Sparse activation separates emitters in time; it does not shrink the diffraction-limited point spread function. A reconstructed image must have enough independent labels to represent its finest claimed feature.
An ionic atmosphere. A negatively charged molecule attracts positive counterions and repels negative co-ions; signs reverse for a positive molecule. The resulting electric double layer partially screens the bare electric field. Far from an isolated molecule, the electrolyte recovers its neutral bulk composition. At thermodynamic equilibrium, spatial uniformity of each species' electrochemical potential requiresThe logarithm implicitly uses a common reference density. This result for Boltzmann ion densities in a symmetric electrolyte neglects ion correlations, finite size and nonideal activities, but shows immediately why equal concentrations of the two signs do not persist close to a charged surface.
Self-consistent screening. Insert these densities into Poisson's equation, with solvent permittivity and fixed charge density :This is the Poisson-Boltzmann equation. For a symmetric monovalent salt with bulk density of each sign, outside the fixed charge it becomesFor , linearizing and using bulk neutrality gives the Debye–Hückel approximationThus added salt shortens the Debye length: electrostatic screening becomes stronger over a shorter distance. The factor of two in a salt comes from two ionic species, not from double-counting the density of salt pairs.
For example, a charged sphere of radius and total charge has the exterior linearized solutionassuming fixed uniform surface charge and no ions inside. It follows from the decaying spherical solution and . At zero salt it reduces to the Coulomb potential; at finite salt it decays exponentially as well as geometrically. The excess mobile charge integrates to in an infinite neutralizing reservoir, although a finite sphere surrounding the molecule generally contains only part of that ionic atmosphere.
Biophysical scales and limitations. In water at room temperature, the monovalent formula is approximately , with the ionic strength. It gives about at and at . Consequently the same charged protein can exert very different long-range interactions mediated by electrostatics at different salt concentrations. Close to strongly charged DNA, the linear approximation fails; nonlinear screening, counterion condensation, ion-specific adsorption and changes of surface ionization through charge regulation may matter. Mean-field theory also misses strong multivalent-ion correlations and finite-size saturation: the exponential law cannot be extrapolated to arbitrarily large near-surface concentrations.
An ion channel can disturb cellular electrical activity by changing unitary electrical conductance, open probability, gating kinetics or the number delivered to the cell membrane. A useful organizing relation isHere outward electric current is positive. Altering one channel's biophysical behavior changes the balance governing membrane potential and hence the timing or recurrence of action potentials.
Long QT syndrome, type 3. Certain disease-associated SCN5A variants impair fast ion-channel inactivation of the cardiac voltage-gated sodium channel NaV1.5. Instead of vanishing promptly after the upstroke, a small persistent inward sodium electric current remains during the plateau and repolarization. Because in this phase, the residual electric current is inward and opposes the outward electric currents that would terminate the cardiac action potential. The ventricular action potential lasts longer, extending the QT interval on the electrocardiogram. Excessively prolonged or uneven repolarization permits early afterdepolarizations and dangerous ventricular rhythm disturbances.
Genetic association identifies the channel, while voltage clamp distinguishes defective ion-channel inactivation from a mere increase in channel abundance. Recordings of disease-associated channels show persistent or bursting openings; coupling measured mutant sodium electric current into an otherwise modeled cardiac membrane through dynamic clamp tests whether that kinetic defect prolongs the action potential. The phenotype is variant-specific: not every SCN5A variant increases late electric current or causes long QT syndrome.[ref]
Cardiac sodium channel mutations in patients with long QT syndrome, an inherited cardiac arrhythmia by Qing Wang and others. Human Molecular Genetics 4, pp. 1603–1607: familial variants affecting the inactivation machinery
[ref]Long-QT syndrome-related sodium channel mutations probed by the dynamic action potential clamp technique by Géza Berecki and others. Measured mutant-channel currents coupled to a ventricular-cell model test action-potential prolongation
Myotonia congenita. CLCN1 encodes the skeletal-muscle ClC-1 chloride channel, which normally supplies a large resting stabilizing electrical conductance. Because the chloride reversal potential is near the resting membrane potential, that pathway resists small depolarizing disturbances. Loss of functional channels, reduced electrical conductance, or a shift in opening toward more positive membrane potential reduces the resting electrical shunt. Potassium accumulation in the transverse-tubule space during activity can then produce larger depolarizing afterpotentials and trigger further muscle action potentials after the intended stimulus has ceased. Continued electrical firing sustains contraction and delays relaxation: this is myotonia, rather than a primary inability of the contractile apparatus to relax.
Patient-family linkage and variant analysis connect the disease to ClC-1. Functional recordings of disease-associated channels demonstrate shifted voltage dependence and reduced availability near resting membrane potential; single-channel and noise measurements also resolve two conductive protopores and their gating behavior. Different variants can act through different mechanisms, so a gating shift is an example rather than an explanation of every case.[ref]
The skeletal muscle chloride channel in dominant and recessive human myotonia by Manuela C. Koch and others. Science 257, pp. 797–800: familial disease linked to the muscle chloride-channel gene
[ref]Mutations in dominant human myotonia congenita drastically alter the voltage dependence of the ClC-1 chloride channel by Michael Pusch and others. Neuron 15, pp. 1455–1463: disease-associated changes in voltage dependence
[ref]The muscle chloride channel ClC-1 has a double-barreled appearance that is differentially affected in dominant and recessive myotonia by Caterina Saviane and others. Single-channel and fluctuation analysis of ClC-1 and myotonia-associated gating changes
These examples connect contrasting current defects to their consequences: persistent inward sodium electric current prolongs cardiac action potentials, whereas loss of stabilizing resting chloride electrical conductance permits repetitive skeletal-muscle action potentials. Both causal chains require functional channel measurements in addition to a disease-associated sequence change.
Articles by others on the same topic
There are currently no matching articles.