The dated cover identifies 22 June 2019 despite the public bundle filename. All optional branches are solved. Graph readings are approximate; conflicting printed chain parameters and kinetic assumptions are distinguished explicitly below.
In bacterial transcription initiation, the RNA polymerase holoenzyme uses a promoter-specific sigma factor to recognize promoter elements and form a closed DNA-bound complex. Subsequent local DNA melting opens a transcription bubble, positioning the template strand in the active site: this is an open promoter complex. The enzyme can then initiate RNA synthesis and escape into elongation. LacI, the lac repressor, binds the lac operator overlapping or close to the promoter and can prevent productive promoter binding or its progression to an open complex; operator arrangement and DNA looping can strengthen repression. One should not assume every repressor acts at exactly the same microscopic step.
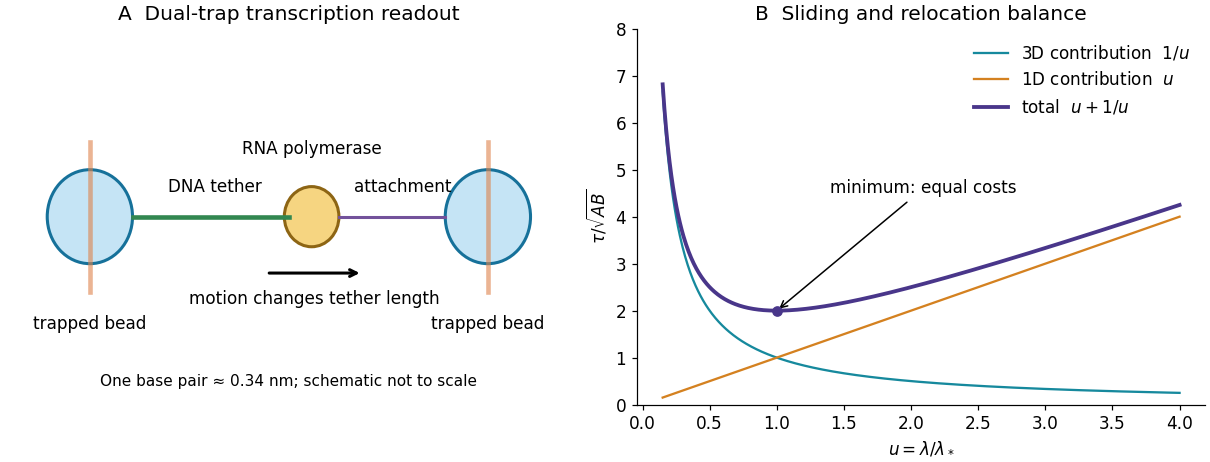
A high-resolution optical tweezers assay mechanically connects one trapped bead to RNA polymerase and another bead to an upstream or downstream DNA handle. Polymerase motion changes the tether length; measuring bead displacement and the calibrated restoring force reports elongation under a known load. A feedback force clamp can keep that load approximately constant. Reversing the tether geometry permits assisting and opposing loads. The left panel below shows the mechanical arrangement rather than a copied apparatus image.
A base-pair advance is only about along B-form DNA. Resolving that increment requires exceptional mechanical stability, suppression of drift and laser-pointing noise, calibration of trap and tether compliance, and sufficient temporal sampling to separate steps from thermal bead fluctuations. Position histograms, dwell detection and their spatial correlations can expose a repeated increment; one should also test nucleotide-dependent motion, pauses and backtracking. Stabilized dual-trap measurements combined with transcription-product analysis established approximately one base-pair advance per incorporated nucleotide.[ref]
Direct observation of base-pair stepping by RNA polymerase by Elio A. Abbondanzieri and others. Single-molecule displacement measurement and independent gel analysis supporting one-base-pair stepping

Treat the target as a stationary perfectly absorbing sphere of reaction radius , surrounded by an effectively uniform reservoir of protein number density . At steady state the radial diffusion equation givesThe inward capture rate per target is the integral of the Fick's first law:For dilute independent targets of number density , the volume association rate is , soThis is the Smoluchowski association rate, in volume per time because the concentrations are number densities. If the target also diffuses, use the relative diffusion coefficient . Orientation constraints, incomplete absorption and chromosome geometry can reduce the actual association rate relative to this ideal collision limit.
The given sphere has radius . The Stokes–Einstein relation at an illustrative givesFor well-mixed independent searchers in cell volume , the target-arrival rate is . The corresponding mean first arrival time isThe source does not fix , the reaction radius or temperature. For an order-of-magnitude estimate, a bacterial volume around and reaction radius – give about –. A 20-base-pair B-form site is about long, supporting a nanometre-scale capture radius but not uniquely defining its spherical value. The estimate is the ideal diffusion-limited time, not a measured intracellular search time: nonspecific binding, orientational matching, crowding and limited accessibility are excluded.
If the outcome is the first successful binding to any operator, ten well-separated functionally independent unoccupied targets give ten times the total capture rate. Henceor roughly – for the estimates above. This assumes nonoverlapping capture zones and no significant depletion before the first event. The first-arrival time at one designated operator is not divided by ten merely because other sites are added, and filling all ten sites is a different occupancy problem.
The term is the bulk-diffusion search cost: increasing the effective length of DNA searched after each encounter enlarges the useful capture region and reduces this contribution. The term is the accumulated sliding cost. Approximately DNA landing-and-sliding episodes, each taking order , give . These are scaling estimates; geometric constants and correlated revisits are omitted by the supplied model.
Thus the facilitated target search is slow as , because too little sequence is examined per encounter, and slow at very large , because sliding and repeated local exploration take too long. A finite intermediate minimum balances 1D scanning against 3D relocation. The right panel of the figure in solution shows the two contributions and their sum. The model requires a useful range of sliding lengths below the full chromosome length, finite positive diffusion coefficients and effective relocation between episodes; it is not a claim that arbitrarily large is physically available.
Write and . Then , soThereforeAt the optimum, the two contributions are equal. Expressing the optimal sliding length directly in terms of the minimum time givesThese relations concern the optimal point; a general nonminimal time can correspond to two different sliding lengths. A geometric or kinetic restriction on the allowed sliding length can instead place the optimum at a boundary.
Use a short inducer pulse to release DNA-bound fluorescent LacI, then remove extracellular IPTG rapidly and start the search clock after washout. The supplied entry, binding and dissociation times imply a synchronization uncertainty of order a few tenths of a second, which must be measured and separated from the search latency. If rebinding is faster than that dead time, the protocol alone cannot resolve the true mean without a kinetic correction or faster triggering.
Image individual cells rapidly enough to distinguish freely diffusing proteins from a persistent immobilized fluorescent spot at the single operator. Prelocate that locus from an independent position marker or a previous binding event. Score the first specific capture after each reset; controls lacking a functional target distinguish stable operator binding from nonspecific DNA residence. Correct for localization error, bleaching, blinking, missed brief events and target motion, and verify that the fluorescent tag does not substantially change the search kinetics.
With four independent freely searching molecules, each having an approximately exponential single-molecule target-arrival time of mean , the first-arrival survival isThus report both the observed first capture among four and the inferred mean for one searcher. If the number of visible available molecules varies, use and account for censoring rather than blindly multiplying by four. Repeated resets and many cells estimate the distribution; deviations from an exponential test the independent well-mixed approximation. The rapid inducer manipulation defines a synchronization strategy, not an assumption that all subsequent intracellular search paths are identical.
Take . Equality of electrochemical potentials for a monovalent cation gives the Nernst equilibrium potentialAt , . ThereforeThe signs refer to the stated electrode convention, not to the direction of current at every voltage. Activities are approximated by concentrations and the bulk ionic concentrations are treated as fixed during a single spike.
The intracellular recording by Alan Hodgkin and Andrew Huxley shows the membrane voltage rising from a negative resting value to a positive overshoot, with the outside held at zero reference. The action potential therefore does more than transiently abolish a resting polarization: it reverses the sign across the membrane. A simple hypothesis that excitation only makes an otherwise potassium-dominated membrane equally leaky cannot explain that positive overshoot.
The result helped motivate a transient, selective change in membrane permeability, later resolved into rapid inward sodium current followed by outward potassium current. The positive sodium equilibrium potential calculated above makes the overshoot physically plausible, while potassium conductance favours a negative resting voltage and repolarization. The 1939 voltage trace itself did not identify individual channel proteins or establish the full later voltage-dependent gating mechanism; those conclusions required ionic substitution and voltage-clamp evidence.[ref]
Action Potentials Recorded from Inside a Nerve Fibre by Alan Hodgkin and Andrew Huxley. 1939 intracellular recording and reversal of membrane voltage during excitation
Panel B steps the membrane from approximately to and holds it there. The sodium current becomes inward, peaks rapidly, and decays almost to zero despite maintained depolarization. At the sodium driving force is negative, consistent with the negative current convention. A conductance description iswhere is channel number, single-channel conductance and the open probability. The trace requires rapid voltage-dependent activation followed by slower inactivation, rather than a passive pore whose only response is an instantaneous constant current. Recovery normally requires repolarization, helping produce a refractory period and directional propagation of excitation.
A typical eukaryotic voltage-gated sodium channel contains four homologous membrane-spanning domains in one large pore-forming protein. Charged S4 helices sense voltage; pore-associated regions form a selective pathway and activation gate. Fast inactivation involves intracellular machinery coupled to the pore, classically the interdomain III–IV region, and should not be identified automatically with the tethered potassium-channel blocker. The pore permits rapid downhill electrochemical transport while maintaining selectivity against other ions.
Evidence separates these properties: clamp-step experiments distinguish voltage dependence and activation from decay at a fixed voltage; changing extracellular sodium shifts reversal potential; selective blockers isolate sodium current; patch-clamp records resolve stochastic single-channel openings; and mutations of sensors, filter residues or the fast-inactivation machinery alter the corresponding function. A single macroscopic trace alone cannot uniquely determine all microscopic rate constants.
Add an unavailable nonconducting inactivated state to the two-state gating scheme, for exampleThe probabilities obeyDepolarization increases activation, initially raising ; subsequent transfer to reduces current while voltage is held constant. Slow recovery at the depolarized voltage permits most channels to become unavailable. Repolarization promotes recovery and deactivation. More closed states and closed-state inactivation may be needed for quantitative data, but this minimal extension already explains the rise followed by decay that fixed-rate gating cannot produce from a closed population.
A sodium-channel gain-of-function mechanism in Long QT syndrome can reduce the inactivation rate or increase recovery/reopening from inactivated states, leaving a small persistent open population. The resulting late inward sodium current opposes repolarizing outward currents while , prolonging the cardiac action potential. Slower entry into would also extend the typical conducting episode relative to its normal duration. The altered effect is prolonged sodium entry, not reversal of sodium's charge or a pump-driven uphill flux through the channel.
The precise rate change depends on the mutation: the clinical label alone does not uniquely specify one transition constant. Long QT syndromes also include other channel mechanisms; the question here concerns its stated sodium-channel variant.[ref]
Cardiac sodium channel mutations in patients with long QT syndrome, an inherited cardiac arrhythmia by Qing Wang and others. Sodium-channel defects associated with the inherited repolarization phenotype
The original Panel A is readable: the baseline is roughly and the peak about , giving a voltage excursion near . Using the specific membrane capacitance and surface area,A coarser spike estimate gives ions, illustrating the precision appropriate to the graph. These are the net monovalent charges needed to charge the capacitor if sodium supplies the inward charge; simultaneous opposing currents can make the actual sodium influx larger.
The cell contains intracellular sodium ions. The capacitive estimate adds only about , or . Thus a spike does not equilibrate bulk concentrations. The sodium-potassium ATPase maintains the gradients over many spikes, exporting three sodium ions per two potassium ions imported per ATP; the estimated sodium load alone corresponds to at least about pump cycles. Rapid repolarization itself comes mainly from changing channel conductances, while sustained fast firing requires adequate energy supply and gradient restoration. The small stated volume and large area are used as supplied, without assuming a particular cell geometry.
Let the common production and removal constants be and , so an unrepressed protein approaches . A simple constructive motif isChoose thresholds , , and . The logic approximation for gene regulation gives , , , and . These unequal thresholds are permitted in this part; the production and degradation rates remain equal.
After input onset, . Production of and begins at , at , and at . Thus the required on-order is obtained. Take an input long enough that all these events occur, for example .
At input termination, , where . The higher direct threshold is crossed first: production stops at , and and production stop at . At that instant , so stops later at . For the example, the delays after are approximately , and in units of :Protein concentrations rise or decay continuously after these switches; “off” denotes cessation of production, not instantaneous disappearance. The first panel below marks the thresholds and the resulting concentrations.
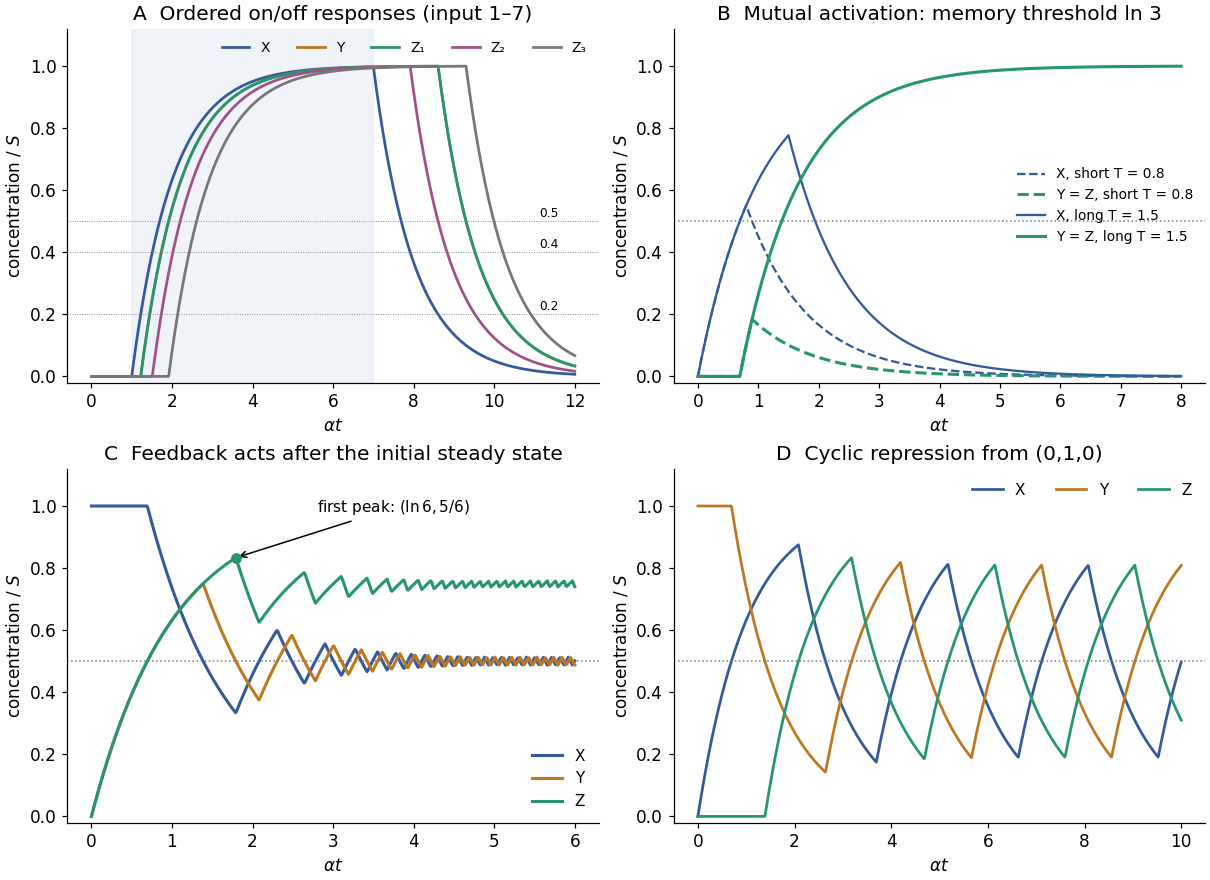
Threshold circuits implement ordered responses, persistent memory, a first output peak and cyclic repression
. Original normalized solutions of the logic models in question 3. All concentrations are divided by and time by ; illustrative common thresholds in panels B–D are . Details.
Put , require , and use the dimensionless time . While X is produced, ; afterwards . X crosses the activation threshold on its rising branch atSymmetry keeps . They initially receive production through X alone and need another interval of active input to reach . If this happens while X is still above threshold, their mutual OR activation sustains production permanently. X remains above untilThe persistence correction to a gene-circuit pulse threshold uses the limiting latch condition is , yieldingFor , and cross their common threshold and approach even after X decays away. For they either remain zero or make a subthreshold pulse and return to zero. Exact equality is sensitive to the convention for the ideal threshold, so robust switching requires a strict excess. At , , whereas and cross at in absolute time.
The shorter required production duration reflects X's persistence after production stops. Requiring would incorrectly discard that tail when all activating ligands remain present. If , no finite pulse reaches the required feedback-active state. The second panel of the figure in solution contrasts pulses shorter and longer than .
For the dynamically regulated interpretation, take , , and let X production respond to Y repression after the ligand appears. Define . Initially active X drives both Y and Z, giving . Y reaches at and switches X production off. X then decays from to , reaching it atUntil , X remains active and Y keeps being produced. Thus . At , Y production stops, but Y still activates Z. Its subsequent decay crosses atImmediately afterwards both inputs to the Z OR gate are below threshold, so Z production stops and its derivative changes from positive to negative. Since Z has been continuously produced from zero until ,For , and . Y repression is lifted at , but X must first rebuild from a subthreshold value, so Z has a genuine first local maximum before any later response.
Wording qualification: if “X is always present at its steady state concentration” is read as an external clamp maintaining after ligand arrival, it overrides Y's repression and changes the problem. Then rises monotonically, with no finite first maximum. The finite-peak result uses the consistent initial-steady-state interpretation in which the stated negative feedback can act.
Write , , , and . The repressilator in the stated logic approximation isAssume . Initially low Z allows X production; high Y blocks Z; and Y is initially at its unrepressed steady level. X first rises through at , turning Y production off. Y then decays through at , where , allowing Z to rise. Z reaches at and switches X production off. At this point , so X falls through at and releases Y production.
Y's rise then switches Z off, Z's fall releases X again, and the sequence repeats. Every segment is exponential relaxation towards one if its production gate is on, or towards zero if off. For a rising segment starting at , the next threshold time is ; for a falling segment starting at , it is . These rules determine the whole trace without pretending the concentrations are square waves. X, Z and Y peak in sequence after the stated initial condition; the last panel of the figure in solution gives an illustrative trajectory.
The delayed sequence of three inhibitory links supplies negative feedback with finite response times. Equal rates make the cycling symmetric after the initial transient, not simultaneous. If , repression is never reliably engaged and the proteins approach their unrepressed levels instead; oscillation is not implied for arbitrary thresholds or for every smooth regulatory law replacing the ideal relay.
A fluorescent reporter associated with one phase of the repressilator should show repeated rises and falls in a tracked cell, with the same underlying oscillatory period but generally delayed and smoothed relative to instantaneous promoter activity. If mature GFP is fused to a repressor and is sufficiently fast to mature, fluorescence approximately tracks that protein's abundance. If GFP is a separately expressed reporter, its own production, maturation, degradation and dilution introduce an additional filter.
For example, converts a periodic gate into a periodic, phase-lagged concentration. Very stable GFP can accumulate a large baseline and obscure oscillations rather than reproducing the regulator trace exactly; maturation delay and bleaching also matter. Biological noise and cell-to-cell phase differences can make individual cycles irregular and wash out oscillations in a population average. The appropriate sketch is therefore a delayed, rounded oscillatory fluorescence trace, with amplitude and baseline depending on reporter turnover, rather than an unqualified copy of a Boolean gate.
At equilibrium, detailed balance requires zero net probability current along each reversible link: . The equilibrium probabilities satisfy , where each state free energy includes its internal degeneracy. ThereforeIn the source sketch B is lower, and the labelled vertical drop is naturally . With that drop convention the ratio is . If instead means the conventional reaction change , the exponent has the minus sign. For example a drop of gives a forward/backward ratio , not .
Write for the probability of state B, so . Gain minus loss givesWith , the solution isIt rises monotonically from zero, initially with slope , towards on time scale . The first panel of the original figure below shows this shape for illustrative equilibrium probability .
The other equilibrium probability is , and their ratio is . Applying detailed balance from part (a) giveswhich is precisely the two-state Boltzmann distribution. It fixes the ratio but not the sum of the rates, so equilibrium measurements alone do not determine the relaxation time.
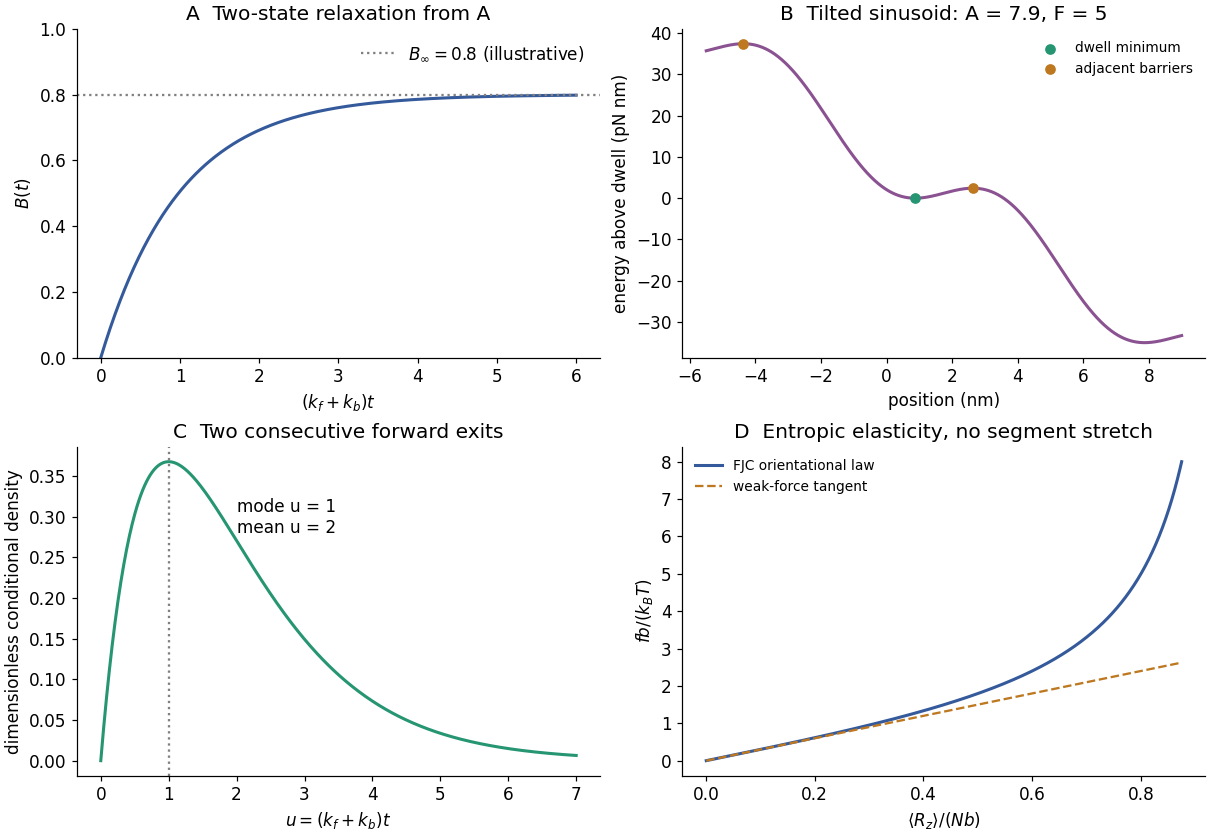
Two-state equilibration, a tilted periodic motor, sequential-step times and freely jointed chain elasticity
. Original model plots, not reconstructions of the source graphs. The motor potential uses sinusoidal coefficient and forward tilt ; other panels use dimensionless axes. Details.
Take forward as increasing , and specify the sinusoidal amplitude convention byThus the unforced barrier is , not . Let and . Stationary points exist because . A minimum is at and its forward saddle at . The distances and activation barriers areUse an Arrhenius estimate with the supplied distance-squared waiting-time scaling, . Calibrate at with and rate in each direction. At the explicit room-temperature estimate , , givingApplying the same distance rule separately backwards gives and hence the literal scaling-model estimateThermodynamic qualification: for isothermal diffusion in this translated tilted potential, adjacent wells differ by , so local detailed balance instead requires . The two separate distance prefactors introduce an extra factor , inconsistent with that requirement. Keeping the forward estimate while enforcing the proper ratio givesBoth interpretations are shown because the supplied distance heuristic is not, by itself, a thermodynamically consistent prescription for both directional prefactors. Additional hidden chemical driving would require its own affinity, not an unexplained prefactor asymmetry. A common transition-state prefactor, as in a consistent Kramers model, preserves the Boltzmann rate ratio. Moreover the forward barrier is only about , so rare-escape exponential dwell kinetics and the numerical rate should be regarded as rough estimates. If “amplitude” meant the entire unforced barrier height, the maximum restoring force would be only and no dwell wells would survive at ; the amplitude convention is therefore essential.
Assume identical dwell states and memoryless forward/backward exits with constant rates and ; put . The probability density for the first exit to be forward at is . For the very next exit also to be forward at time , multiply by and integrate over the unobserved first time:This density integrates to , the probability that both directions are forward. Conditional on that event, the normalized total-time density is the Erlang distributionIts mean is , so the most probable time is not the mean. Since both backward-rate conventions in part (c) have , neglecting backwards steps gives the usual approximation and mode . If “two forward steps” instead permits intervening backwards events, thinning independent Poisson exits gives that latter rate- distribution directly; it describes a different conditioning. The low barrier noted in part (c) limits the physical accuracy of all these memoryless dwell assumptions.
In a tensile atomic force microscopy measurement, a DNA tether connects the cantilever tip and a surface. Moving the support stretches the molecule, and calibrated cantilever deflection supplies the tensile force; extension must be corrected for cantilever deflection and any linkers. At low force, extension mainly straightens an initially fluctuating coil, giving approximately linear entropic elasticity. At higher force the available conformations become increasingly aligned, so additional extension costs progressively greater force. The readable source curve then continues beyond the nominal inextensible-model contour length, which signals a failure of that simple model or of the stated parameter interpretation, rather than negative elasticity.
An inextensible freely jointed chain of links of Kuhn length has contour length and cannot be extended beyond it at any finite force. There is an explicit numerical contradiction in the printed parameters:The discrepancy is present in the original page, not introduced by digitization. To obtain with links requires ; to obtain it with requires . No single inextensible FJC can satisfy all three stated numbers. The graph's much larger extension is an immediate counterexample to treating the literal as an accurate global fit.
Separately, accepting the graph's nominal contour as an effective low-force model, its continuation to is about beyond that contour. An inextensible ideal chain contains orientational entropy only; it excludes stretching of segments, energetic compliance of bonds, changes in helix structure or base pairing, and heterogeneous attachments. An extensible freely jointed chain or a semiflexible-chain model with appropriate energetic terms can describe some departures. Calibration or contour-length assignment can also be wrong. The graph alone does not identify which mechanism contributes, and its displayed moderate forces do not justify assigning a specific high-force DNA structural transition. Arithmetic inconsistency in is not explained away by these physical mechanisms.
Let the applied force be . A segment with polar angle has energy . Independent 3D orientations give the one-link partition functionTaking the force derivative of yields the mean end-to-end projection,For , , soIsotropy supplies the vector relation. It is the mean vector or its projection, not the mean magnitude of a fluctuating chain; at zero force while remains positive. The last panel of the model figure in solution shows the exact orientational response and its weak-force tangent.
The weak-force spring constant isUsing the literal printed , at givesThis is a calculation with the quoted parameters, not a self-consistent fit to the plotted contour. If instead and are retained, then and . Retaining and gives . These distinct alternatives quantify the unresolved parameter inconsistency rather than silently choosing a correction.
The restoring force is entropic. Stretching selects a small fraction of the many disordered orientations, reducing conformational entropy. The Gaussian chain free-energy cost is , whose gradient gives the Hooke-law coefficient above. In an ideal inextensible chain, individual bonds need not change their length to generate this force.
At fixed and , the entropic spring constant is proportional to absolute temperature, because the free-energy penalty for a given loss of conformational entropy is . ThereforeFor the literal printed chain this is . The same factor multiplies either alternative contour-consistent spring constant from part (d), provided its Kuhn length is held fixed. Real DNA's persistence length, base pairing and solvent interactions can themselves vary with temperature and salt; then contributes through at fixed segment count, or if the physical contour is instead held fixed. The simple linear temperature result belongs to the specified ideal-chain model.
After the load is removed, a reversibly stretched DNA molecule relaxes towards a thermally fluctuating coil, releasing stored free energy as heat through the surrounding fluid. There are many more disordered chain conformations than strongly aligned ones, so entropy favours retraction; viscous drag sets how rapidly it occurs. At long times an unconstrained ideal chain has zero mean end-to-end vector but a nonzero typical size, ; it does not contract to a point.
At finite temperature the chain continues fluctuating, and an anchored or otherwise constrained molecule need not regain an isotropic ensemble. If stretching broke attachments, denatured the DNA or caused irreversible structural changes, recovery can be incomplete or hysteretic. Those outcomes cannot be decided from the ideal FJC alone.
The hydrophobic core of a lipid bilayer makes transfer of a hydrated ion into bare lipid energetically costly. An ion channel supplies a water-accessible route across that barrier. Its narrow selectivity filter presents coordinating chemical groups that compensate for loss or rearrangement of the ion's hydration shell. Selectivity depends on the free-energy balance of hydration, coordination, electrostatics and geometry, rather than a sieve that passes all smaller ions.
A potassium-channel filter presents backbone carbonyl oxygens in a geometry favourable for potassium; smaller sodium does not automatically gain the same energetic compensation. Sodium and calcium channels use different filter architectures: charged side chains and their coordination environments favour particular ions, with ion occupancy and competing species also affecting permeation. In canonical vertebrate voltage-gated sodium channels, the DEKA selectivity ring illustrates chemical discrimination distinct from potassium-channel carbonyl coordination. The precise mechanism therefore depends on the channel family.
Rapid flux requires low successive free-energy barriers, not permanent binding of the preferred ion. Several occupied sites, nearby water and ion–ion interactions can facilitate passage without requiring the ion to cross the lipid. For scale, a open channel driven by carries , approximately monovalent ions per second. A nanometre-scale route with favourable coordination can support such rapid, thermally driven motion. An ion channel is not an ATP-driven pump: net flux follows the electrochemical potential difference,which vanishes at the species' Nernst equilibrium potential. ATP-consuming pumps maintain the gradients that make sustained channel currents possible.
Permeation selectivity and opening probability are separate properties. Voltage-sensor movement, ligand binding or mechanical tension can regulate access to the pore, while inactivation can terminate conduction during a maintained stimulus. Patch-clamp unitary currents establish discrete conducting states; reversal potentials under changed ionic compositions quantify selectivity. Structure determination locates the filter and gates, and mutations or specific blockers test their functional roles. Agreement between these measurements is stronger evidence than structure or current shape alone.
A charged biological molecule attracts counterions and repels ions of the same sign. Thermal diffusion opposes complete localization, producing a mobile ionic atmosphere whose charge partly cancels the molecule's electric field at larger distances. Solvent polarization also reduces the field through its permittivity, but that dielectric response is distinct from the mobile-ion screening cloud.
For an ideal electrolyte in equilibrium at temperature , an ion of valence has local number densityFor , linearization about an electroneutral bulk givesThis is the Debye length. Here counts each species separately and is the absolute solvent permittivity. For a point charge , outside its immediate molecular environment the linearized solution isIt is a screened potential, not a claim that the molecular charge has disappeared.
In terms of ionic strength with in , the density sum is , soIn water near , : about at and at . Increasing ion density or valence shortens the range; temperature and solvent permittivity also matter. The displayed temperature dependence holds at fixed permittivity, which itself changes with temperature in water.
The derivation assumes dilute mobile ions, a continuum uniform dielectric and weak potentials. Near highly charged DNA or protein surfaces, nonlinear Poisson-Boltzmann equation behaviour, counterion condensation, finite ion sizes, specific binding and correlations can matter. At physiological salt the predicted length approaches molecular scales, so the formula is a useful far-field scale with limited microscopic accuracy, rather than a complete account of the first hydration layer.
Fluorescence localization precision can be much finer than the image width: a fluorescent molecule produces a diffraction-broadened point spread function, but the centre of that distribution can be estimated much more precisely than its width. Fit the measured camera counts to a calibrated point-spread model with position, brightness and background parameters. For an ideal Gaussian image of standard deviation and independent detected photons, the centroid precision scales asPixelation and background worsen this limit. A useful approximate variance for square pixels of width and background rms noise photons per pixel isThis estimate requires a correctly specified isolated image and appropriate noise model. Drift, optical aberration, dye motion, linkage offset, bleaching and motion blur introduce further errors; localization precision alone does not guarantee absolute positional accuracy.[ref]
Precise nanometer localization analysis for individual fluorescent probes by Russell E. Thompson and others. Photon number, pixel size and background dependence of localization uncertainty
In the Myosin V measurements, total internal reflection fluorescence microscopy reduced background and a two-dimensional Gaussian fit localized a single dye attached to a light chain with roughly precision. The motor's centre advances about per cycle. A hand-over-hand mechanism instead moves the rear head about past the stationary front head, exchanging their roles. A label displaced by from the midpoint therefore gives alternating displacements and nm; near a head this tends towards alternating and nm. An inchworm model would give approximately uniform nm label displacements. Resolved unequal alternating steps therefore distinguish the mechanisms, with interpretation depending on the label geometry.[ref]
Myosin V Walks Hand-Over-Hand: Single Fluorophore Imaging with 1.5-nm Localization by Ahmet Yildiz and others. Single-light-chain fluorophore localization, alternating displacements and hand-over-hand interpretation; Science 300, 2061–2065 (2003)
For sub-diffraction imaging, arrange that only a sparse, spatially separable subset of fluorophores emits in each frame, localize those emitters, then combine many frames into a map. Photoactivation or reversible stochastic switching provides the sparse subsets. Distinct nearby molecules can then be localized at different times, circumventing overlap of their simultaneously emitted diffraction patterns. The achievable structural resolution depends on photon-limited precision, label density and linkage, repeated blinking, drift correction and specimen motion; arbitrarily many fits to the same dye do not supply missing labels elsewhere. This is the principle behind PALM and STORM, with their different switching strategies.[ref]
Sub-diffraction-limit imaging by stochastic optical reconstruction microscopy (STORM) by Michael J. Rust and others. Sequential sparse activation and localization of fluorophores to reconstruct a super-resolution image
Articles by others on the same topic
There are currently no matching articles.