Mathematical biology uses mathematical models to connect biological mechanisms with quantitative predictions. Differential equations can track changing quantities, while population dynamics, enzyme kinetics and gene regulatory networks ask how growth, reactions and feedback shape living systems. A useful mathematical model states its assumptions and units: a simple chemostat, for example, reveals how nutrient supply and removal jointly determine whether a culture persists.
The system , combines logistic prey growth, saturating predation and a predator carrying level proportional to prey density. Its unique positive equilibrium is , where . Its Jacobian matrix has determinant and trace . The positive trapping construction for the Leslie-Gower model gives a compact positive region and a limit cycle whenever this equilibrium is a repeller.
A rectangular upper bound , , is inward pointing for the Leslie-Gower predator-prey model. To avoid the singular edge , use and the inequality , obtained by completing a square. Choose sufficiently small and . Then , , is a compact forward-invariant set in the positive quadrant. Removing an outward-flow neighborhood of a repelling equilibrium leaves a trapping region without equilibria, so the Poincaré-Bendixson theorem yields a periodic omega-limit orbit.
In a biological competition model, increasing one population reduces the growth of another. A two-species example is , , with both cross-effects negative. This asymmetric example has self-limitation only in ; disappearance of therefore permits unbounded growth of . For its positive coexistence equilibrium is a saddle whose stable manifold separates exclusion outcomes.
For the population map , extinction is a superstable fixed point. Below , two positive fixed points exist. Their multipliers are , making the lower one a threshold and the upper one attracting. A saddle-node bifurcation removes them at ; above it for every positive population, so every nonnegative orbit tends to extinction.
The mathematical description of elastic bodies whose stress-free material state changes through growth or remodelling. A multiplicative decomposition of the deformation gradient separates the growth tensor from the elastic accommodation . The relaxed grown configuration need not be globally compatible, so even an unloaded body can develop internal stress.
For , these Lotka-Volterra equations describe two populations limited by their own density and depressed by the other population. The nonnegative quadrant is invariant. Positive equilibria are intersections of the non-axis nullclines and ; their existence and stability distinguish stable coexistence, competitive exclusion, and bistability. Positive solutions have no periodic orbits: multiplying the vector field by the Dulac function makes its divergence , so the Bendixson-Dulac theorem applies. Boundedness, boundary equilibria, and their stable manifolds must still be checked before concluding convergence to one particular equilibrium.
For , , choose and weights . Then , strictly negative away from coexistence. The function diverges at the positive-quadrant boundary and at infinity, keeping trajectories in compact interior level sets. This proves global convergence for positive initial states, while boundary-axis data retain their single-species dynamics.
The FitzHugh-Nagumo model represents an excitable cell by a fast activation variable and a slower recovery variable. A common nondimensional form is , . Its cubic activation response and recovery feedback can produce an excitable resting state or sustained oscillations through bifurcations. Particular reductions and travelling-wave equations can have additional state variables; their signs and parameter conventions must be stated separately.
For the scalar reaction-diffusion equation with and , an exact decreasing travelling wave isIndeed , and substitution into leaves the factor , proving the speed formula. A zero speed gives the Maxwell balance for a scalar reaction-diffusion front. In a FitzHugh-Nagumo model this calculation requires treating the recovery variable as frozen externally: retaining with exactly constant forces to be constant.
A recovery variable represents feedback that reduces activation after an excitation in a FitzHugh-Nagumo model. Its equation must be specified separately from the activation equation. Holding it externally constant gives a scalar reduction; requiring it to remain constant while keeping its original evolution equation generally imposes an additional constraint and need not permit the same solutions.
For , , set . Intersections of the nullclines solve . Three simple equilibria are possible precisely when and , where . To prove this, observe that has two real zeros exactly when ; monotonicity on the three resulting intervals counts the intersections. At either endpoint there are a double and a simple root, and at , there is one triple root.
An epidemic is a period of growing infection incidence in a population. Compartmental models describe transmission, recovery and depletion or renewal of susceptible hosts. An epidemic invasion threshold concerns growth after a small introduction; a final size relation for an epidemic concerns the total susceptible depletion of a closed outbreak. These are distinct from an endemic equilibrium with continuing transmission.
A metapopulation describes occupied habitat patches with local colonization and extinction. The patch occupancy variable differs from population abundance within a patch.
This model couples deterministic underdominant allele-frequency dynamics in equal-sized habitats by global migration. Starting with pure habitats of one allele and of the other preserves two within-class frequencies , reducing the system to , with . Migration is conservative in the mean, but selection need not conserve global allele frequency.
With equally many initially pure habitats of each allele, symmetry preserves . The heterogeneous equilibrium exists for . Its full-system eigenvalues are in the mean-frequency direction and in the antisymmetric direction, so it attracts general nearby perturbations only for . Exact symmetry can preserve both alleles beyond this robust range; at stronger migration it approaches the unstable uniform midpoint.
In the two-class globally coupled underdominant metapopulation, the rectangle , is forward invariant under the displayed bound. On its inner edges, selection points inward with magnitude while outward migration is at most or ; the outer edges also point inward. Thus prescribed initial state cannot approach global allele fixation when . Maximizing gives at , making the bound optimal within this particular symmetric worst-case rectangle argument, not a universal sharp migration threshold.
Colonization of empty habitat at rate and extinction of occupied habitat at rate give the displayed patch-occupancy equation. The positive equilibrium is when . Competition can be incorporated through replacement fluxes between patches occupied by different species.
A resident trait occupies fraction when its colonization rate exceeds fire extinction. With net competitive replacement given by ability difference , a rare mutant has the displayed per-capita growth. The selection gradient is . A singular trait with negative mutant-fitness curvature is a strict local evolutionarily stable strategy. Global strict uninvadability requires that be smaller than its resident value for every other trait. Monotonicity alone does not specify the shape or existence of an optimum.
An Allee effect makes per-capita growth less favorable at low abundance. A strong effect permits a stable zero state and a stable positive state separated by a finite threshold. Cooperative infections can exhibit the same positive-feedback structure: neither disease invades alone, but sufficiently many joint infections sustain both.
A food web records resource-consumer interactions among species. A linear food chain is a special case. Positive interaction coefficients alone do not imply persistence: the per-capita growth balances must admit feasible positive long-term mean abundances.
Two consumers with different break-even requirements cannot both have bounded persistent abundance on a single well-mixed limiting resource when their per-capita growth is linear in that resource. For and , differentiation of gives the nonzero constant when their break-even levels differ. This excludes simultaneous bounded persistence without assuming convergence to an equilibrium. Additional resources, environmental variation or different interactions can invalidate the simple one-resource argument.
A food chain orders species so that each consumer feeds on the level below and may be eaten by the level above. Basal resource growth, consumer mortality, conversion efficiency and density regulation determine whether all levels can persist.
For an unregulated exponential basal resource and nearest-neighbor Lotka-Volterra equations, the weighted interaction matrix is skew-symmetric matrix. An even chain has an invertible tridiagonal interaction matrix; its positive equilibrium, when feasible, fixes all long-term means. An odd chain has a null direction and requires a special balance between resource growth and mortality to permit bounded full coexistence. For a three-level chain, . A positive even-chain equilibrium gives a conserved coercive relative-entropy-type function, proving every species remains bounded above and away from zero.
A network describing how gene products affect the production of other gene products. Positive and negative regulatory interactions can generate multistability, oscillations, and noise-sensitive transitions.
// Target: mathematical-biology.bigb
A repressilator is a cyclic negative-feedback gene regulatory network in which three repressors inhibit one another in sequence. In a normalized logic approximation for gene regulation, , , . For , threshold crossings successively switch production and can generate sustained oscillations. A rise from reaches threshold after ; a decay from reaches it after in units of the common decay time.
A gene product reduces its own production. This negative feedback can stabilize its abundance and shorten the approach to a regulated level. In the strong logic approximation for gene regulation, production switches off near a self-repression threshold; a smooth repression law avoids artificial infinitely rapid switching at that threshold.
At a Hill equation equilibrium with , differentiating gives the displayed logarithmic sensitivity. It approaches one without effective feedback and under strong repression. Threshold pinning in the logic approximation for gene regulation instead gives approximately zero production sensitivity while the threshold is held fixed.
Neglecting the one in a strongly repressed Hill equation gives . The substitution makes this a linear ordinary differential equation. It yields and half-response time . The singular initial slope is an artifact of the approximation, whose range is not uniform at arbitrarily large and fixed production/degradation ratio.
A threshold approximation in which a regulatory input permits or blocks production according to whether a transcription factor exceeds a specified concentration. With first-order removal, and . A zero-initialized rising response reaches at . Boolean rules must specify how several inputs combine; equal rate constants do not determine thresholds.
Suppose an input is produced for time , then decays, and activates two identical mutually activating OR-gated outputs. Write and . The input remains above threshold until . Each output reaches threshold at if input remains available. Equating these times gives the limiting pulse duration . Exact equality depends on the ideal gate's boundary convention; a robust latch requires a longer pulse. Treating cessation of production as immediate removal incorrectly discards the input's residual lifetime.
A feed-forward loop has regulatory paths and . The two inputs are combined at the target gene using a specified regulatory rule.
In an incoherent feed-forward loop, the direct path from an input to an output and the indirect path through a second transcription factor have opposite net signs. Their different response times can generate a pulse or adaptation. A nonzero basal production rate makes the final adapted output nonzero, so its logic and response time must be calculated from the actual gene regulation rule rather than assumed from a Boolean label.
In the I4 incoherent feed-forward loop, an input activates the output but represses an intermediate activator of that output. Decay of the intermediate can interrupt an initial output pulse. Residual production and signal dependence must be retained when specifying the gene regulation rule.
In the I1 incoherent feed-forward loop, an input activates both an intermediate regulator and the output, while the intermediate represses the output. Delayed accumulation of the intermediate can therefore interrupt an initial output pulse. The precise steady state depends on the actual gene regulation rule and thresholds.
Let an output start at zero, degrade at rate , and switch from production to at time , with . Its final level is . Writing , its first crossing of occurs at if ; otherwise it occurs at . This follows by solving the two linear differential equations before and after the switch. A large F alone does not make the first formula uniform in arbitrarily short pulse durations.
The direct path and the indirect path of a coherent feed-forward loop have matching overall signs. The all-activating case with an AND rule can delay activation while allowing rapid removal of the production signal when the direct input disappears.
The all-activating feed-forward loop combines direct activation of an output with indirect activation through an intermediate. Under AND logic the intermediate's accumulation delays production and can reject brief inputs. Removal of direct activation stops production immediately, while the output concentration still has its own decay time.
A persistence detector responds strongly to a sustained input and weakly to short isolated inputs. In an activating coherent feed-forward loop, an intermediate protein accumulates toward a threshold while the target also requires the direct input. Eliminating that intermediate by an instantaneous quasi-steady-state approximation removes its accumulation delay.
The interacting regulatory system built from pair-rule genes. Its interactions can change with developmental time rather than forming one static circuit.
An oscillatory developmental regulatory system associated with repeated segment formation. Oscillation, intercellular synchronisation and fixation of boundaries are distinct processes.
Two components mutually repress when each inhibits the other's production. With decreasing , the two negative interactions create a positive feedback loop. Sufficiently strong repression can produce two stable states: high , low , and the reverse.
// Target: mathematical-biology.bigb
For and , subtraction of the equilibrium conditions gives . The symmetric state solves . Two asymmetric positive states exist precisely for : , . Their Jacobian matrix has eigenvalues , both negative; the symmetric state is then a saddle point. For only the attracting symmetric state remains.
For , , the equilibrium slope product is . A value gives a saddle separating attracting alternatives. Both exponents greater than one allow this at sufficiently large common . If both are at most one it is impossible. If , define as the unique positive solution of and set . All equilibria are parameterized by , whose derivative is . Thus multistability for some common strength occurs exactly when . For the maximum is . Consequently alone is not sufficient when the two synthesis strengths are required to coincide.
For positive , this mutual repression system can display bistability for some exactly when both and . If either exponent is at most one, it has a unique stable equilibrium for every . To prove the less obvious case , put and at equilibrium. Equality of the two expressions for gives . The loop gain is then bounded by , whose maximum is . Swap the two components for the other case. If both exponents exceed one, sufficiently large yields two stable equilibria with and . The weaker condition is sufficient to exclude multistability, but does not exhaust all exclusions when the same production prefactor is imposed.
// Target: mathematical-biology.bigb
At an equilibrium , , the Jacobian matrix has eigenvalues . Its product of repression gains is also . Product below one gives a stable node, above one a saddle, and equality the threshold for a zero eigenvalue. Robust multiple stable equilibria require an intervening unstable equilibrium; a gain exceeding one alone is not a sufficient global criterion for a particular pair of repression functions.
// Target: mathematical-biology.bigb
The Monod equation is an empirical saturating law for the specific growth rate of a culture limited by one nutrient. Write for its residual nutrient concentration, for the limiting specific growth rate, and for the nutrient concentration at half that rate:Here and have units of inverse time, whereas has the same units as . The notation in the title denotes the same growth function, with , and . For , ; for , approaches . Its derivative is positive: more nutrient increases the specific growth rate, with progressively smaller increments.
For example, take and . Nutrient concentrations of , and give specific growth rates , and . In a chemostat with dilution rate , the intersection selects the residual nutrient concentration , provided the feed can supply enough nutrient for a positive biomass concentration.
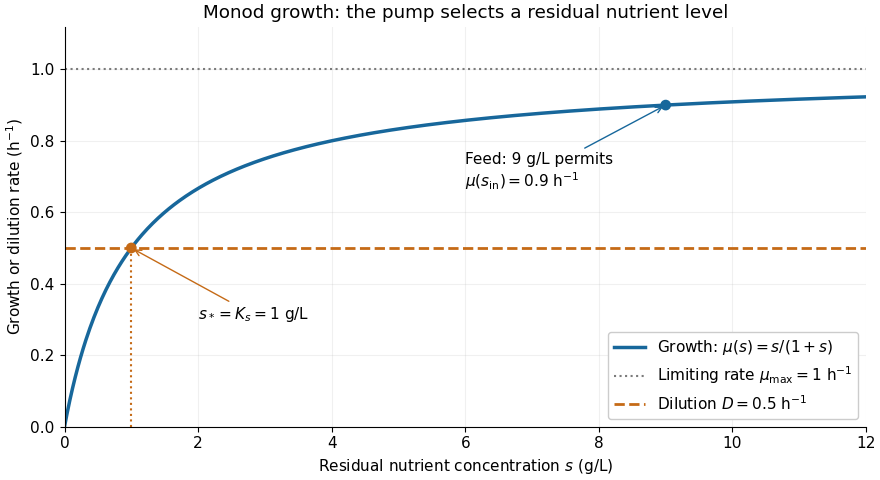
The Monod equation is useful because two measurable parameters describe both nutrient scarcity and saturation. It assumes the other conditions affecting growth remain controlled and does not represent inhibition at high nutrient concentration. Although its formula resembles the Michaelis-Menten equation, a whole culture's specific growth rate combines many processes; the resemblance alone does not derive it from Michaelis-Menten kinetics or identify with a Michaelis constant.
In his 1949 review, Monod presents the hyperbolic rate law as an empirical fit in equation (2), pp. 383-384, and discusses the difficulty of identifying a single growth-controlling reaction. His reported division rates use doublings per unit time; the natural-exponential specific growth rate used here is that division rate multiplied by . [ref]
https://garcialab.berkeley.edu/courses/papers/Monod1949.pdf. Jacques Monod, The Growth of Bacterial Cultures, Annual Review of Microbiology 3 (1949), 371-394, DOI: 10.1146/annurev.mi.03.100149.002103
.The specific growth rate is biomass production per unit existing biomass per unit time. For biomass concentration with growth alone, and . A constant positive specific growth rate produces exponential growth, , with doubling time . In a chemostat, removal makes the net rate , rather than itself.
A chemostat maintains a well-mixed culture at constant volume by feeding fresh nutrient solution and removing culture at the same volumetric flow . Its dilution rate is . Mixing makes the outflow's nutrient concentration and biomass concentration equal to those inside the vessel; continuous replacement supplies nutrient and also removes growing cells.
The simplest one-nutrient chemostat uses nutrient concentration , biomass concentration , constant feed nutrient concentration , and constant biomass yield . Assume a cell-free feed, one growth-limiting nutrient, constant volume, and no cell retention, death or additional nutrient consumption for maintenance. With specific growth rate , its ordinary differential equations areThe nutrient balance contains inflow , outflow , and consumption ; the biomass balance contains production and removal . If is in grams of nutrient per litre and in grams of dry biomass per litre, is grams of dry biomass produced per gram of nutrient consumed. Thus both balances have units of their respective concentration per time. The Monod equation supplies an empirical choice of ; the balances themselves express the stated production, consumption and transport assumptions.
The appeal of a chemostat is that, at a positive chemostat steady state, adjusting the pump sets the specific growth rate to . The residual nutrient concentration then adjusts to that rate, and the available nutrient together with biomass yield sets the biomass concentration. This gives a controlled way to compare cultures at selected growth rates and a simple quantitative warning of chemostat washout.
Two 1950 publications on continuous culture are Novick and Szilard's Description of the Chemostat, Science 112(2920), 715-716, dated 15 December, and Monod's La technique de culture continue. Théorie et applications, Annales de l'Institut Pasteur 79, 390-410. The latter's original bibliographic details are reproduced in the contents of Monod's collected papers. These references identify contemporary publications without establishing priority between them. [ref]
https://doi.org/10.1126/science.112.2920.715. Aaron Novick and Leo Szilard, Description of the Chemostat (1950)
. [ref]https://api.pageplace.de/preview/DT0400.9780323142632_A23647608/preview-9780323142632_A23647608.pdf. Monod's 1950 original, listed in Selected Papers in Molecular Biology by Jacques Monod, contents p. vi
.The biomass concentration is the mass of biological material per unit culture volume; here it is measured as dry cell mass in . A biomass concentration differs from a cell count per unit volume because cell sizes can change. In the ideal chemostat, biomass leaves the vessel at rate , giving a removal term in the ordinary differential equation for .
The biomass yield converts nutrient consumption into biomass production: consuming nutrient mass produces dry biomass mass under the assumed constant conversion. For , consumption of of nutrient produces of dry biomass. Its numerical value depends on the measurement conventions; it is not a fraction of all feed mass converted into cells. With no separate maintenance consumption, biomass production requires nutrient consumption in the chemostat balance.
A chemostat steady state has constant nutrient concentration and biomass concentration even while nutrient and cells flow through the vessel. It is an equilibrium of the chemostat ordinary differential equations, rather than a culture in which all growth has stopped. Assume and the Monod equation. Setting both derivatives to zero gives the always-existing chemostat washout equilibrium . A positive biomass concentration instead requires growth to balance removal, , whenceThe positive chemostat steady state exists exactly whenThe weaker condition only makes the denominator positive; it does not ensure or . Because the Monod equation is increasing, the feed must permit a specific growth rate greater than . At a positive chemostat steady state, increasing feed nutrient concentration at fixed increases the biomass concentration without changing , within the one-nutrient assumptions.
For a concrete chemostat, let , , and . At ,The nutrient supply minus outflow is , matching nutrient consumption . Biomass production and removal both equal . The chemostat washout threshold is . For example, formally gives and , which cannot describe a physical culture.
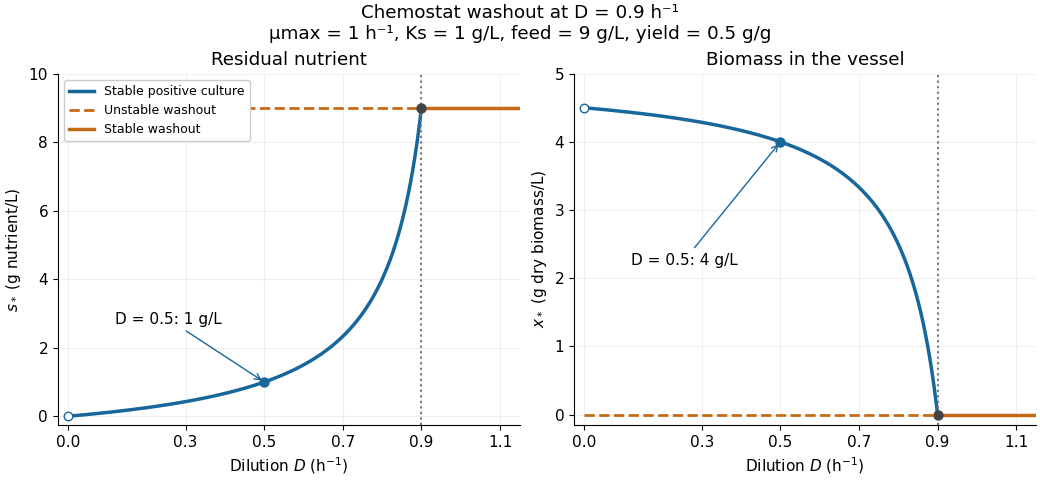
There is a useful exact simplification: the nutrient-equivalent concentration satisfies , so . This combines dissolved nutrient and the nutrient equivalent of biomass; it does not assert that these two variables account for every chemical constituent. In coordinates , the Jacobian matrix at the positive chemostat steady state has eigenvalues and , both negative. Hence the positive chemostat steady state is locally asymptotically stable. In the worked example the eigenvalues are and .
Chemostat washout means the culture's biomass concentration tends to zero because growth cannot sustain replacement of the cells leaving the vessel. In the ideal Monod equation chemostat with , its equilibrium is . Its Jacobian matrix has eigenvalues and : a small inoculum grows when , whereas chemostat washout is locally asymptotically stable when . For nonnegative initial concentrations, chemostat washout occurs for ; the boundary case also loses biomass asymptotically.
At the positive chemostat steady state meets the chemostat washout equilibrium, and one eigenvalue is zero, so linearization alone does not decide the boundary case. On the invariant nutrient-equivalent balance , small positive obeys : nutrient consumption lowers the specific growth rate below , leading to slow decay rather than a positive biomass concentration. The continued mathematical branches exchange stability in a transcritical bifurcation; the positive-biomass branch becomes physically inadmissible beyond .
For a dimensionless chemostat with Monod equation kinetics,the total nutrient equivalent satisfies . The positive equilibrium is , , provided and . The Jacobian matrix has eigenvalues and , so the positive equilibrium is locally asymptotically stable.
The dilution rate is the fraction of a constant-volume chemostat replaced per unit time: volumetric flow divided by culture volume . For and , . A well-mixed constituent with no source and absent from the feed has concentration , since . Thus is the time for its concentration to fall by a factor , not the time by which all original material has left.
At a positive chemostat steady state, the specific growth rate equals the dilution rate; the biomass concentration stays constant because production balances outflow. For , growth alone would have doubling time , even though the vessel's biomass concentration does not double. Raising the dilution rate beyond causes chemostat washout; comparing it only with misses the nutrient limitation imposed by the feed.
A seed-producing population with first-season and second-season recruitment leads to nonnegative recurrence coefficients . Its characteristic roots are . The nonnegative dominant root is below one precisely when , giving deterministic decay of every finite initial population. This is a mean-population model; literal integer extinction requires a stochastic interpretation or a separate integer-population argument.
A population model has density dependence when its per-capita recruitment, survival or growth depends on population abundance relative to habitat or resource scale. Negative density dependence reduces per-capita growth as crowding increases. In a discrete-generation model, a strong enough decline can make the next total population decrease as the present total increases, producing overcompensation and possible alternating generations. The ecological mechanism and the mathematical stability calculation should be distinguished.
Overcompensation occurs when a larger present population produces a smaller total population in the next generation over part of the relevant range. It is stronger than a decline of per-capita growth alone. For with , the large-abundance response decreases with abundance. Stronger feedback can drive a fixed-point multiplier through minus one, but that local threshold alone does not establish chaotic behaviour.
A per-capita mortality rate means that the death flux from a biological population of size is . With constant rate and no other transfers, gives exponential survival . In an epidemic model this can specify mortality from the infective compartment rather than mortality of the entire population.
Constant harvest effort removes individuals at rate proportional to their current population, with fixed coefficient . Its continuous model subtracts from the growth rate, while a discrete model may use . This differs from constant-quota harvesting, which subtracts a population-independent amount. A discrete rule must remain nonnegative on its physical state range, or require a separately specified truncation.
For and with , extinction changes stability at , while the upper stable population and an unstable separator merge at . If , an interval of efforts supports stable extinction and a stable positive population simultaneously; at the positive state collapses. If the thresholds have the opposite order, the high-population pair disappears before the lower stable branch reaches extinction. At a positive equilibrium stability follows from the sign of .
For and strict concavity, per-capita recruitment strictly decreases because . Thus a positive fixed point is unique if it exists. A slope makes extinction unstable but does not guarantee a positive intersection: stays above the identity. A large-population restriction supplies existence; the local fixed-point stability condition remains .
The rate of addition through birth to a specified biological population. State whether a rate is absolute or per capita and specify its time unit.
A stage-structured population model tracks distinct life stages, such as juveniles and adults, with separate reproduction, survival and transition terms. A matrix update describes the linear case; density-dependent reproduction gives a nonlinear discrete dynamical system.
A carrying capacity is an abundance scale at which a specified environment's net population growth vanishes. In the logistic growth equation, positive unharvested populations approach . It depends on the species, resources and environment rather than being an immutable universal population limit.
The useful distinction is between a growth rate and a sustainable abundance. In a logistic differential equation, controls how quickly a population responds, while the carrying capacity sets the positive equilibrium point. Increasing with fixed accelerates approach without raising that equilibrium. Increasing changes the destination. The logistic differential equation diagrams show populations approaching the same carrying capacity from below and above.
In ecological use, the carrying capacity describes what a particular environment can support under specified conditions. Nutrient supply, available space, and accumulated waste can change those conditions; it is not a permanent property of a species alone. A population temporarily above a carrying capacity is possible. In the simplest constant- logistic growth equation, its net growth becomes negative; real population dynamics can include delays, seasonal variation, and changing resources that the basic mathematical model omits. [ref]
https://openstax.org/books/biology-2e/pages/45-3-environmental-limits-to-population-growth. Clark, Douglas and Choi, Biology 2e, §45.3: carrying capacity and environmental limitations
.The Nicholson-Bailey model describes seasonal host-parasitoid interaction. Hosts surviving random attacks reproduce, while parasitoid offspring are proportional to attacked hosts. For , its positive equilibrium is , . Counting attacked rather than surviving hosts makes its predator reproduction law different from the annual pulse-breeding predator-prey model.
At the positive Nicholson-Bailey model equilibrium, lies between one and two, and the displayed determinant exceeds one. These follow from for . The discriminant is therefore negative, and the conjugate eigenvalues have moduli greater than one. Nearby annual samples spiral outward rather than approach coexistence.
Two populations grow at the same per-capita rate and each loses members at a rate proportional to their product. On the invariant diagonal , the logistic differential equation gives for and positive rates. The positive symmetric equilibrium is stable along that diagonal but unstable transversely: , while the Jacobian matrix has eigenvalues . Thus an exactly symmetric deterministic solution can relax toward coexistence while a small imbalance grows. A corresponding density-dependent Markov jump process has a controlled fluid limit on each fixed finite interval, rather than uniform control for all time.
The logistic growth equation applies the logistic differential equation to population dynamics. For positive growth rate and carrying capacity , an initial condition gives , where . Its per-capita growth falls linearly with abundance, and a trajectory starting below reaches an inflection point when . The exact solutions of a differential equation and their diagrams are developed under logistic differential equation. A translated and scaled logistic function has the same form. In nonlinear regression for biological size, an analogous saturation curve need not imply that circumference itself obeys a mechanistic population law.
For a fixed catch rate , natural logistic growth can replace the catch at two abundances if . The upper equilibrium attracts, and the lower is an unstable survival threshold. They meet in a saddle-node bifurcation at , . Above this catch every positive population declines to zero. Below it a population initially under also becomes extinct. A constant catch is stopped at extinction to avoid negative abundances; it is distinct from per-capita harvesting proportional to .
The Ricker population map models density-dependent reproduction with a declining per-capita growth factor. Its nonzero equilibrium is , with multiplier . It loses stability through a period-doubling bifurcation at . Every population after the first update is bounded by , the maximum of the update function on nonnegative populations.
For and , a nonzero second-iterate fixed point satisfies . A genuine pair has the displayed form, and its periodic-orbit multiplier is . At , the pair is exactly , with periodic-orbit multiplier . For large its upper point is asymptotic to and the pair periodic-orbit multiplier to , so eventual instability follows despite the small derivative at the upper point.
Here is the low-density per-generation multiplication factor and sets the inverse crowding scale. The positive fixed point is when ; its derivative lies strictly between minus one and one, so it is locally asymptotically stable. The map reaches its maximum at and decreases thereafter. Stability follows from the derivative, not from assuming that every overcompensating population map undergoes period doubling.
Starting at with , the next two iterates are the maximum and its image . Since and the squared-denominator population map decreases on , its image there lies in . Thus the displayed interval is invariant after the initial step, and both bounds are attained. The initial value itself is below , so it must not be included in the lower-bound assertion.
Roots of unity among the linearization multipliers give periodic linearized perturbations but do not by themselves prove a branch of nonlinear periodic solutions. For the normalized delayed recurrence , the multipliers at are . Nevertheless, with , its sixth iterate has leading displacement , where and . The identity obstructs cancellation for small nonzero . Indeed any putative local six-cycle requires by the norm equation, and then its determinant equation would read , impossible. This is a concrete caution against promoting a linear resonance to a nonlinear bifurcation assertion.
The density of individuals at age evolves by transport with unit ageing speed and loss rate . New individuals enter at age zero through the integral birth boundary. Exponential separated profiles lead to the Euler-Lotka equation.
For with , integrating the age-structured population equation replaces its exit integral by . For one-to-one transition from stage one to stage two and two-to-one reproduction from stage two to stage one, the population matrix is . This follows by integrating the age derivative and substituting the incoming boundary conditions. Exact time-independent positive profiles also force a constant stage ratio and common exponential growth through those boundary conditions. Thus the constant-coefficient closure is not an exact transient description for arbitrary age-dependent hazard functions and arbitrary initial conditions; constant hazard functions are an important exception for the integrated populations.
A cell-cycle age density counts biological cells per unit time spent in one specified phase of the cell cycle. Its integral over phase age is the population in that phase. Phase age resets on entry into the next phase, so it differs from chronological age since birth. A phase-exit hazard function supplies loss from the phase and incoming flux to the next phase.
The mean lifetime number of offspring is the birth rate integrated against the probability of surviving to each age. For a continuous age model it is . The Euler-Lotka equation compares this with one to locate positive population growth.
A fixed-size neutral population evolves by reproduction events in which one individual replaces another. Types are copied along directed reproduction arrows. Backward ancestral lineages merge when one such arrow joins them; the coalescence rate depends on the chosen time normalization.
Randomness in individual births, deaths and maturation makes a finite population fluctuate even in a fixed environment. Near a deterministic extinction threshold it can drive the population into an absorbing extinct state.
Mathematical epidemiology uses mathematical models and statistical inference to study the occurrence, transmission, and control of disease in populations.
An irreversible serocatalytic model describes the transition from seronegative to seropositive after infection. If the force of infection is and detectable antibodies persist, the seronegative fraction satisfies , hence seroprevalence is when . Antibody loss needs a reverse transition, and imperfect testing needs a separate observation model.
Seroprevalence is the proportion of a specified population with a positive result for a specified antibody assay. Its biological interpretation depends on assay diagnostic sensitivity, diagnostic specificity and the persistence and origin of the measured antibodies. It is not itself the incidence rate of new infection.
Each undirected cross-group partnership is counted once from each group's contact total. Thus group size times per-person contact rate times cross-group fraction must agree. If one group occupies fraction while its cross-group per-person rate stays fixed, aggregate cross-group contact is order and the other group's cross-contact fraction is order . Assigning both per-person rates independently generally breaks this balance.
A macroparasite burden model tracks the distribution of within-host parasite burdens and couples it to transmission or environmental infectious stages. Mean burden alone is insufficient when worm mating, nonlinear fecundity, immunity or host mortality depend on that distribution.
For sexually reproducing worms, an infected host need not contain both sexes. Independent random sexes split a Poisson total burden of mean into independent male and female Poisson distributions of mean , giving the displayed probability of a fertile mixed-sex burden. For an arbitrary burden probability generating function , this probability is . Its low-burden behaviour can introduce an Allee effect in transmission, so an asexual mean-burden invasion calculation is not automatically valid.
If host-specific equilibrium mean burden has a gamma distribution, conditional Poisson distributions produce a Poisson-gamma mixture, hence a negative binomial distribution. With mean and shape , its zero-burden probability is . Decreasing increases aggregation: a smaller infected-host prevalence can accompany the same mean burden and more heavily infected individuals.
Independent worm acquisition at rate and loss at rate produce a birth-death process for within-host parasite burden. Summing its forward equations against gives . At constant exposure, detailed balance yields a Poisson distribution with mean . Heterogeneous acquisition rates change the pooled burden distribution even when each individual host follows this model.
A stochastic epidemic model represents infection and recovery as random events. A continuous-time Markov chain can track integer counts, while a stochastic SIR model illustrates random fade-out and finite-population outbreak variability that a deterministic limit does not show.
In a continuous-time epidemic model, a constant recovery rate gives an exponential distribution of infectious duration with mean . Other duration distributions require additional stages or infection-age structure.
Quarantine restricts contacts of exposed individuals whose infection status is uncertain, with monitoring to detect illness. It differs from isolation of recognized infected or ill individuals. An incubation period quantile can enter a duration calculation, but assumptions about exposure time, symptom detection and infectiousness are needed before the calculation describes transmission risk.
Before isolation, the closed SIR model has first integral . If quarantine occurs at the first crossing , the corresponding susceptible count is the root on the outbreak branch of . Immediate prevention of further transmission makes the number infected among the initial susceptible class equal to .
When exposed animals remain in a not-yet-infective compartment for a fixed incubation period , stopping all new exposure does not cancel the pending case transfers. At isolation time , their number is for smooth profiles. Eventual cases therefore include this pipeline in addition to case transfers already completed by . The interpretation depends on the compartment definition: a strictly unexposed susceptible compartment would instead lose these animals at exposure.
The incubation period is the interval from infection to symptom onset in a person who develops symptoms. Its probability distribution describes onset times, not the full timing of infectiousness. Exposure may only be known to fall in an interval, requiring a corresponding observation model when estimating this distribution.
Observed symptom-onset intensity is the convolution of past infection intensity with the incubation delay density: . Back-calculation infers the infection history from that relation. Include pre-observation infections unless their absence is known.
For equal-width time bins and infections assigned to bin-end time , let . The next onset-bin mean is . Assigning infections instead to bin starts shifts the index by one. Bin probabilities integrate a delay density; they are not the density itself.
Articles were limited to the first 100 out of 460 total.
Articles by others on the same topic



Mathematical biology is a field that applies mathematical methods and models to understand biological systems and phenomena. It integrates concepts from mathematics, biology, and often computer science to address questions related to biological processes. The objectives of mathematical biology can vary widely and might include: 1. **Modeling Biological Processes**: Developing mathematical models to describe biological phenomena, such as population dynamics, disease spread, ecological interactions, and cellular processes.